


Carbohydrate metabolism, glycolysis, glycogenesis and gluconeogenesis
Carbohydrates are classified in several groups, namely:
1). Monosaccharides are carbohydrates that cannot be hydrolyzed into simpler
carbohydrates, for example glucose.
2). Disakarida is a condensation product of two monosaccharide units, for
example lactose, maltose and sucrose.
3). Oligosaccharide is a product of three to ten monosaccharide condensation. 4).
Polisaccharides are more than ten monosaccharide condensation products, for
example starch and dextrin which may be linear or branched polymers.
Carbohodrat metabolism
Glucose is the most important carbohydrate, most carbohydrates in food are
absorbed in bloodstream as glucose formed through hydrolysis of starch and
disaccharides in food and other sugars are converted into glucose in the liver.
Glucose is the main metabolic fuel in mammals (except Biak Hamat) and
universal fuel for the fetus.
Metabolism is a term used to explain the interconversion of chemical
compounds in the body. The path taken by each molecule, inter-molecular
relations, and mechanisms that regulate the flow of metabolites through
metabolic pathways. Metabolic routes are classified into three categories,
namely:
1). The anabolic path is a path that plays a role in a greater and more complex
compound synthesis of smaller precursors, for example protein synthesis of
amino acids. Anabolic routes are endothermic.
2). Katabolic pathways, namely the path that plays a role in decomposition of
large molecules, often involves oxidative reactions, this path is exothermic,
which produces reducing equivalent and especially through the respiratory
chain, ATP.
3). The amphibolic route is the path that takes place at the intersection of
metabolism, works as a liaison between the parallel and anabolic path, for
example the Krebs cycle.
Glycolysis
Glycolyhof also called the Embenden Meyerhof line is a metabolic pathway used
by most autotrophic and heterotrophic organisms, both aerobic and anaerobes,
to begin to break down glucose. The name of the glycolysis literally means glyco
means sugar while the lysis means solution.
Glycolysis is a metabolic pathway and is an anaerobic energy source used by
almost all types of organisms. This process requires oxidation of glucose
molecules, the only most important organic fuel in plants, microbes, and
animals. Most cells prefer glucose (there are exceptions, such as acetic acid
bacteria that prefer ethanol). In glycolysis per glucose molecule it will use 2 ATP
molecules and produce 4 ATP, 2 NADH, and 2 pyruvate. Pyruvate can be used in
the Krebs cycle, or serves as a precursor for other reactions.
Steps - the glycolysis path of the Embenal-Meyerhof path consists of:
1. Change of glucose into 6-phosphate glucose (G6-P)
a. This reaction is catalyzed by the hexocine enzyme using ATP
b. The reaction is irreversible and glucose trapped efficiently in cells,
because the compound between phosphorylated does not easily penetrate
the cell membrane
2. G6-P to FRUKTOSA 6-phosphate (F6-P)
a. This reaction is catalyzed by phosphoisoglukoisomerase
b. This enzymatic stage prepares the C-1 atom for phosphorylation
c. Is a back and forth reaction, governed by the substrate levels (stikiometric
settings)
3. F6-P becomes fructose 1.6-diphosphate (F1,6-DP)
a. This reaction is catalyzed by phosphosruktokinase
b. The reaction is irreversible
c. Phosphosruktokinase in some networks is the glycolysis rate of boundary
enzyme. This enzyme is the main regulator enzyme glycolysis path.
4. F1.6-DP Becomes Dihidroxial Phosphate (DHAP) and 3-phosphate
glysticdehyde (G3-P).
a. The first stage of glycolysis (hexose into triosa phosphate) ends in this
reaction that is catalyzed by an aldolase.
b. Fructose 1.6 diffosphate is broken down into two 3-carbon molecules, one
of which is the Metabolit of Precursors.
c. The entire glucose c atoms can end as pyruvate, because there is a
balance between DHAP and G3P, catalyzed by Triosa Phosphate
Isomerase. With the use of G3P for further glycolysis reactions, the C Din
atom is converted to G3P.
5. G3-P to 1.3 diffosphoglyerates (1.3 DPG).
a. This reaction is catalyzed by glyceraldehyde 3 phosphate degodrogenase
(G3PD), requires nicotinamid adenin dinucleotides (NAD) as electron
wildeners.
b. In this reaction phosphorylation occurs over the use of inorganic
phosphate (PI) and is an example of the oxidative phosphorylation of the
substrate level.
6. 1.3-DPG into 3-phosphoglyerates (3-PG)
a. This reaction is catalyzed by phosphoglyerating kinase
b. This reaction is the first ATP formation in glycolysis. This is another
example of the substrate level oxidation phosphorylation.
7. 3-PG into 2-phosphoglyerates (2-PG)
a. This reaction is catalyzed by phosphoglyerating mutase
b. This reaction requires 2.3 diffosphoglyerates (2.3 DPG) in a low level as a
cofactor.
c. In almost all 2.3 cells there are low levels
d. Conversely in red blood cells 2.3 DPG levels approximately 4mm (the
same as hemoglobin molarity) in red blood cells, where 2.3 DPG acts as an
oxygen transport regulator, strengthens the form of hemoglobin
deoxygenation
8. 2-PG becomes phosphoenolpiruvat [pep].
a. This channel is catalyzed by enolation
b. Phosphoenol bonds are high energy phosphate bonds
9. Pep becomes pyruvate
a. This reaction is catalyzed by pyruvate kinase
b. The formation of ATP from ADP by using high-energy phosphoenol bonds
from PEP is another example of the oxidative phosphorylation of the
substrate level
c. Formed 2 pyruvate molecules per initial glucose molecule. So the clean
ATP formed per glucose molecule in the formation of pyruvate is +2 (-2 + 2
+ 2)
Kreb Cycle Reaction
The Krebs cycle was taken from the name German biochemist Hans Krebs, who
identified its steps in the late 1930s, metabolized a two-carbon unit called the
acetyl group to CO2 and H2O. It is also called a tricarboxylic acid cycle, because
some molecules in the cycle have three carboxyl (COOH) groups, or citric acid
cycles, because citric acid is an important substance. Before pyruistic acid
(glycolysis results) can enter the krebs cycle, pyruvate acid must first be
converted into acetyl-koa. This complex reaction involves the disappearance of
one co2 molecule, electron transfer to NAD, and the addition of coenzyme A
(KOA). In Prokarota, this reaction occurs in the cytoplasm; In eukaryotes, they
occur in the mitochondrial matrix.
Oxidative decarboxylation
Pyruistic acid is a aerobic glycolysis final product must be transported into the
mitochondria before it can enter the Krebs cycle. This can be done by specific
pyruvate transporters who will help Pyruvate past the inner Mirokondria
membrane. Once pyruvate has reached the matrix, Pyruvate will be converted
into the acetyl of the KOA by the Pyruvat Dehydrogenase complex which is a
complex multienzyme. The pyruvate dehydrogenase complex is actually not a
part of the Krebs cycle, but is the main source of coA-substrates containing two
carbons for cycles. The pyruvate dehydrogenase complex is a collection of
multimolecules consisting of three enzymes and five coenzymes. Three
enzymes namely pyruvate dehydrogenase (E1) are also called decarboxylase,
dihydroPoat transasetilage (E2), and dehydrolipoat dehydrogenase (E3). Five
coenzymes work as a carrier or oxidant for reaction of intermediates. E1
requires pyrophosphate thiamine, E2 requires lipoatic acid and coenzyme A and
E3 requires FAD and NAD +.
Krebs cycle
The Krebs cycle plays a role in the metabolic process. This cycle is the last
pathway where carbohydrate oxidative metabolism, amino acid meetings and
fatty acids and changing the carbon frame becomes CO2 and H2O. This
oxidation process provides energy for the establishment of most of the ATP in
charge of animals including humans.
Steps - Krebs line steps like;
1. Synthesis of citrate from acetyl koa and oxaloacetate
a. The Krebs cycle starts from the acetyl condensation of KOA and
oxaloacetate to form citrate, catalyzed by citrate synthase
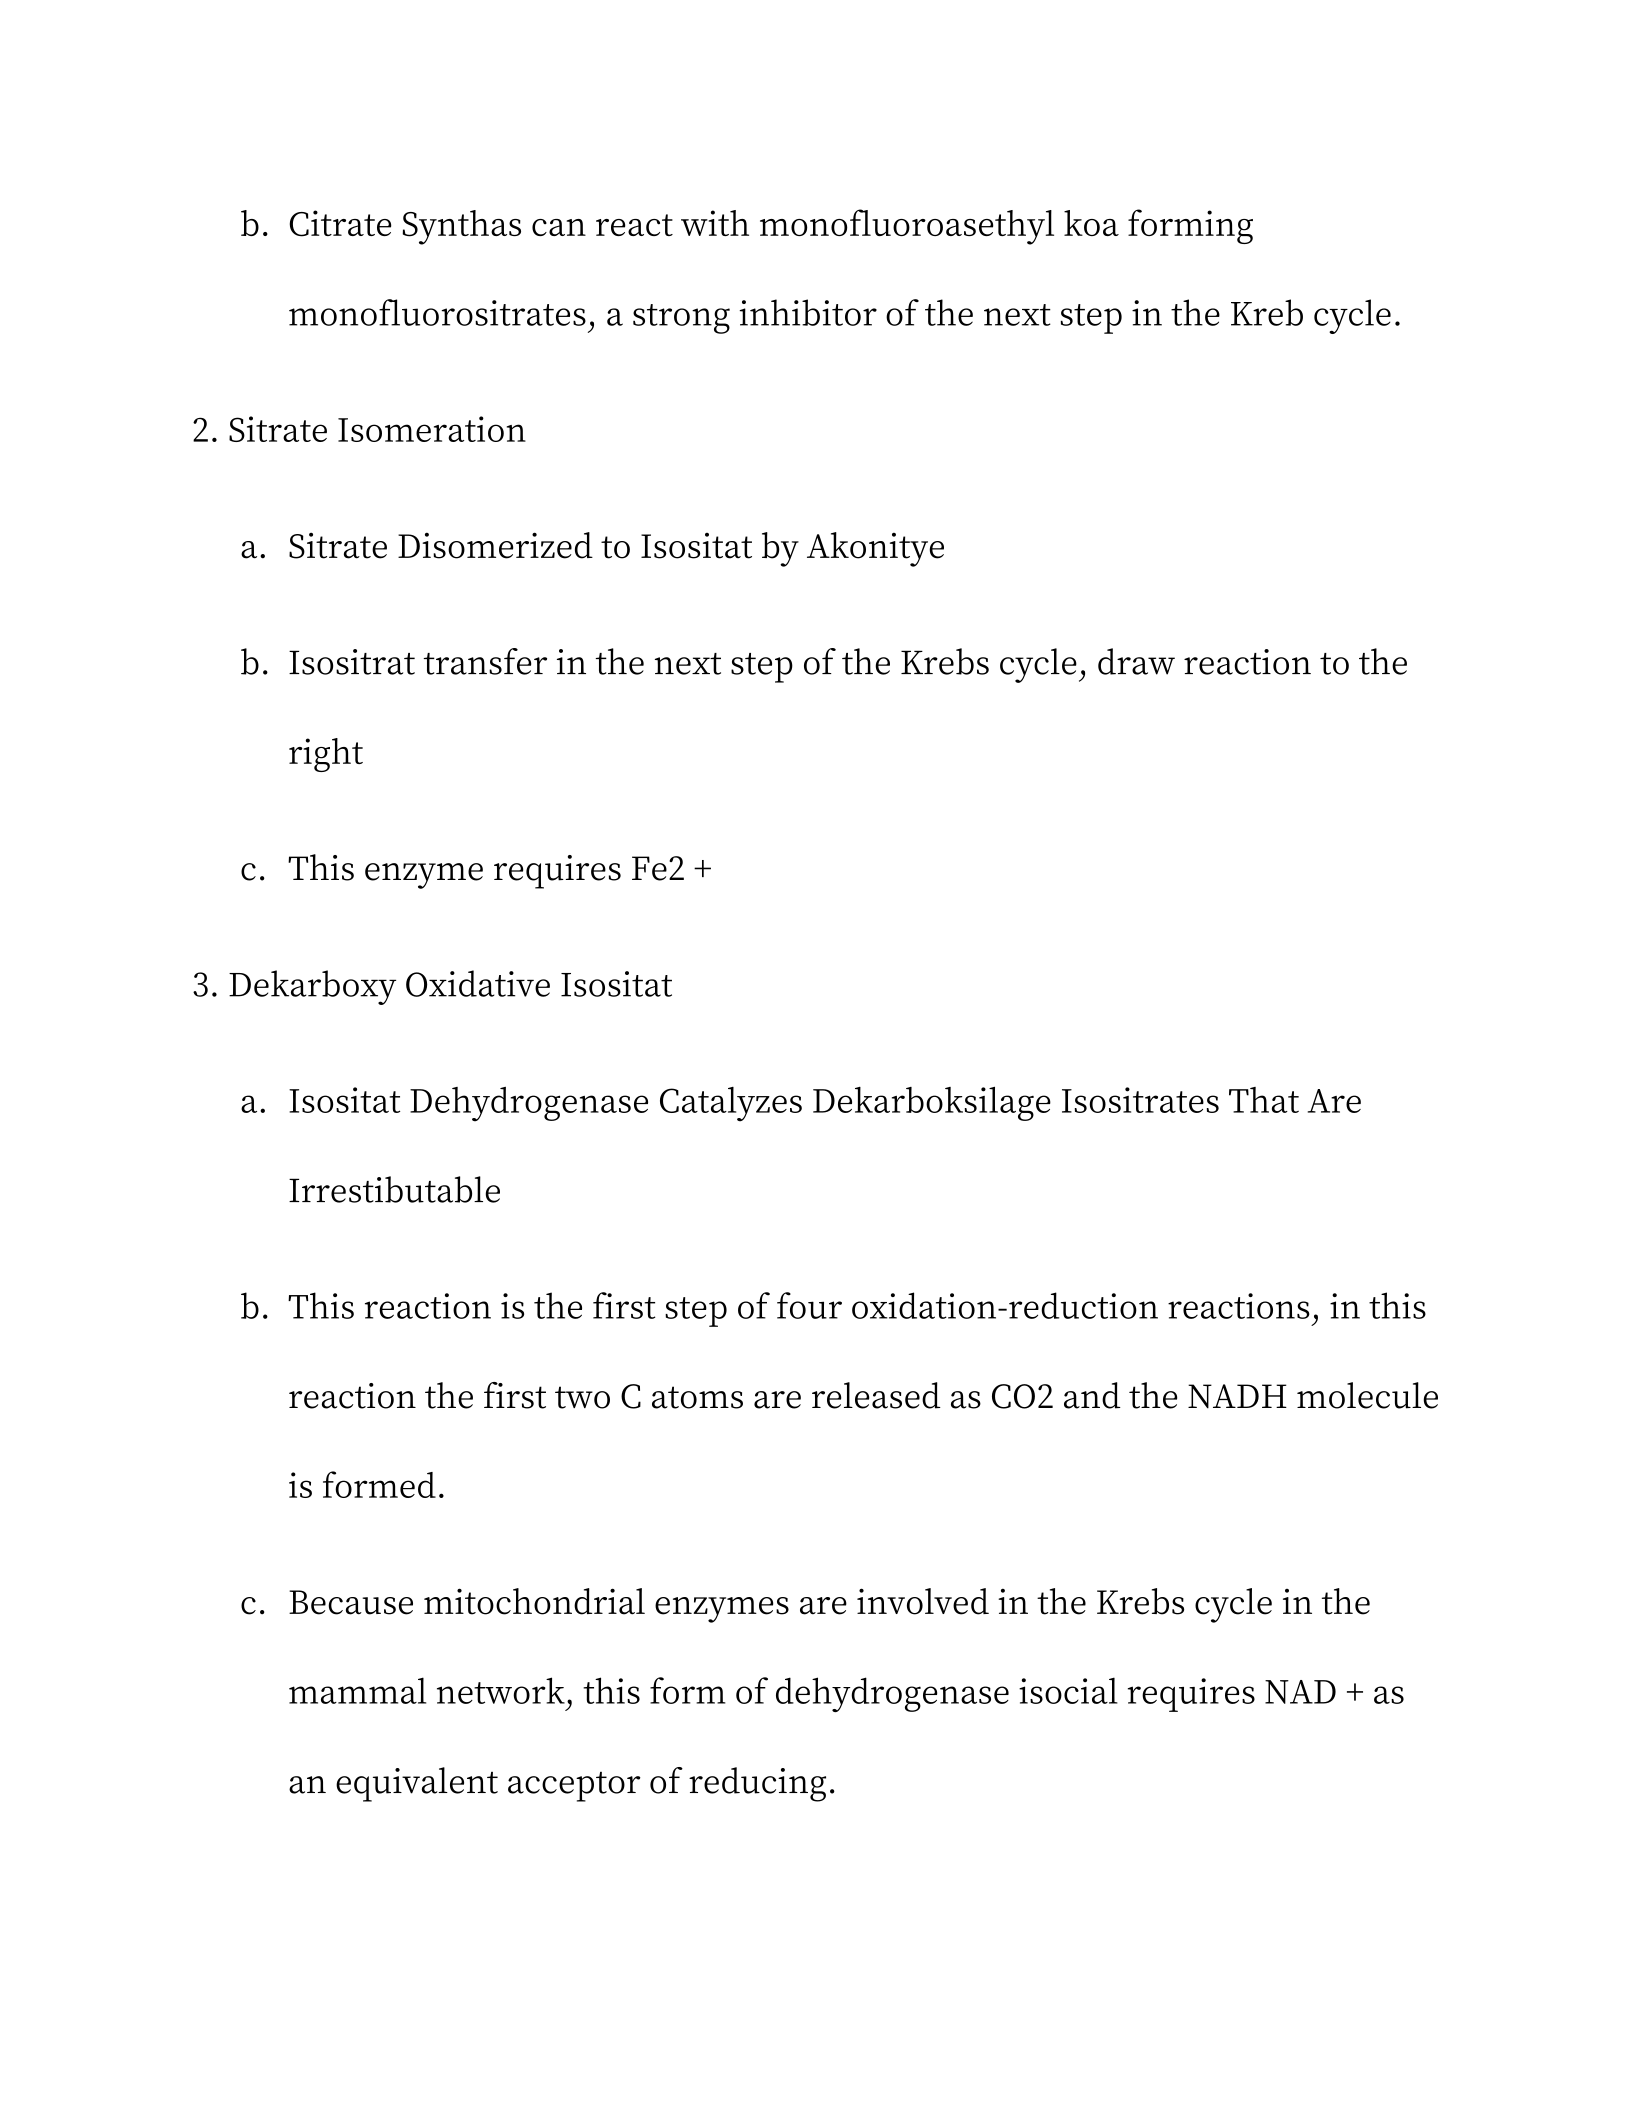
b. Citrate Synthas can react with monofluoroasethyl koa forming
monofluorositrates, a strong inhibitor of the next step in the Kreb cycle.
2. Sitrate Isomeration
a. Sitrate Disomerized to Isositat by Akonitye
b. Isositrat transfer in the next step of the Krebs cycle, draw reaction to the
right
c. This enzyme requires Fe2 +
3. Dekarboxy Oxidative Isositat
a. Isositat Dehydrogenase Catalyzes Dekarboksilage Isositrates That Are
Irrestibutable
b. This reaction is the first step of four oxidation-reduction reactions, in this
reaction the first two C atoms are released as CO2 and the NADH molecule
is formed.
c. Because mitochondrial enzymes are involved in the Krebs cycle in the
mammal network, this form of dehydrogenase isocial requires NAD + as
an equivalent acceptor of reducing.
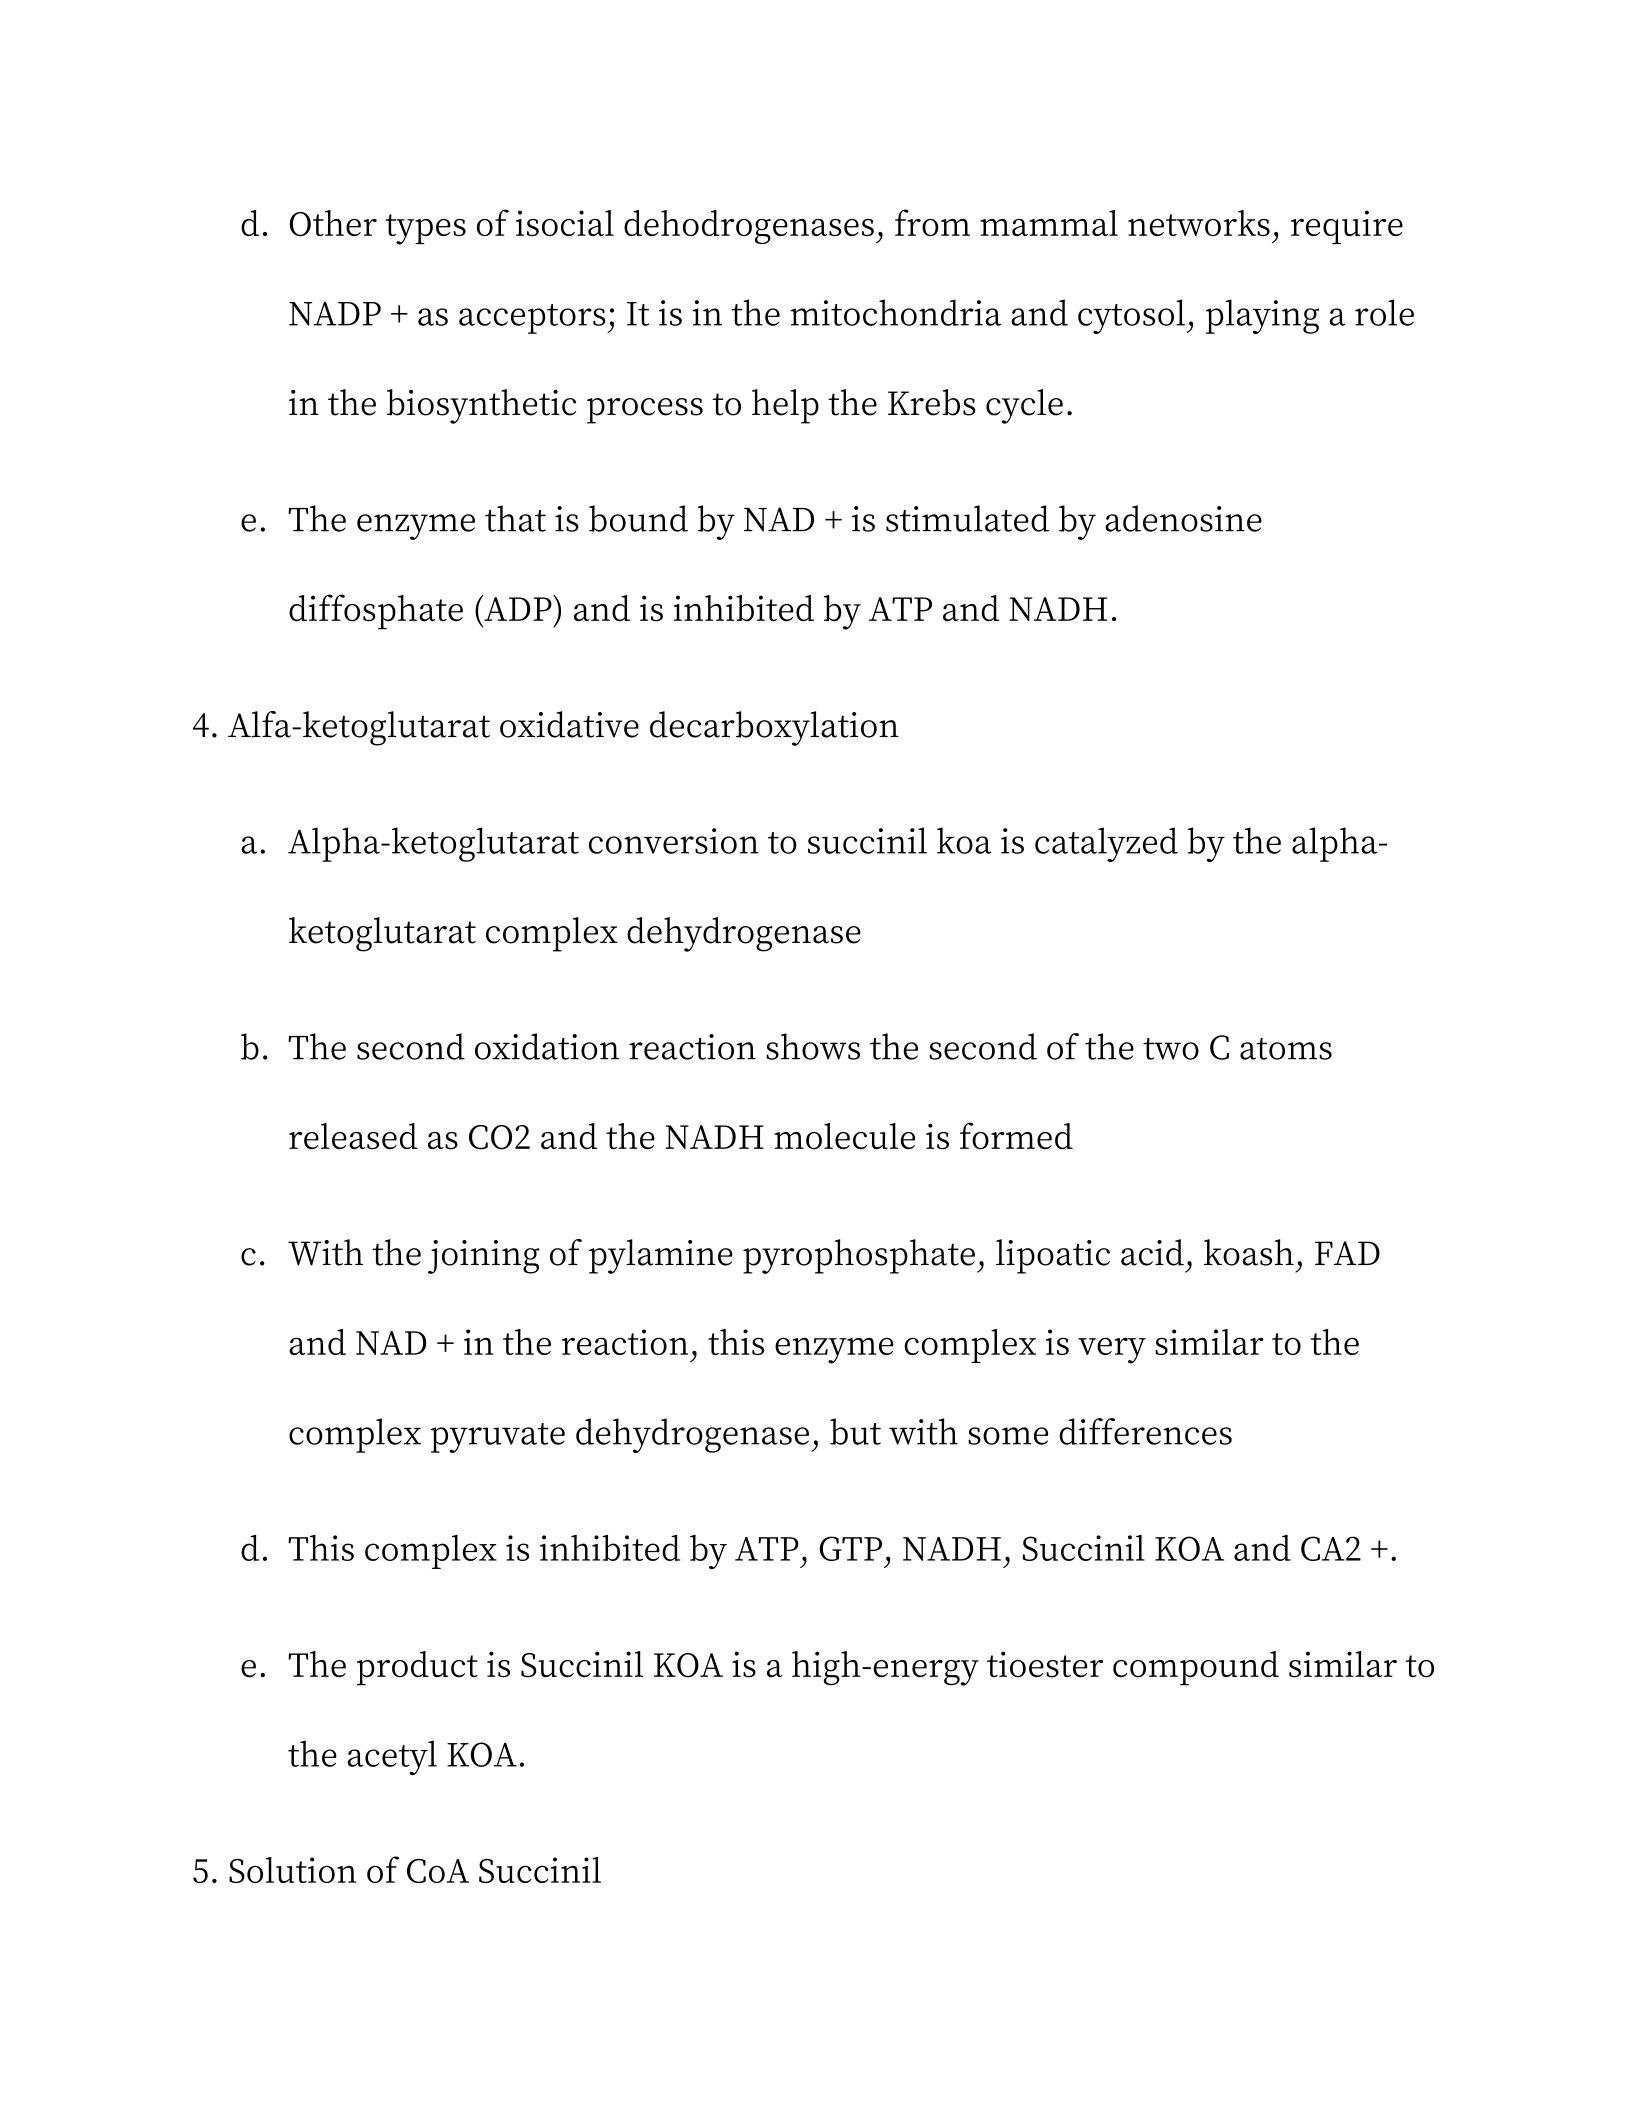
d. Other types of isocial dehodrogenases, from mammal networks, require
NADP + as acceptors; It is in the mitochondria and cytosol, playing a role
in the biosynthetic process to help the Krebs cycle.
e. The enzyme that is bound by NAD + is stimulated by adenosine
diffosphate (ADP) and is inhibited by ATP and NADH.
4. Alfa-ketoglutarat oxidative decarboxylation
a. Alpha-ketoglutarat conversion to succinil koa is catalyzed by the alpha-
ketoglutarat complex dehydrogenase
b. The second oxidation reaction shows the second of the two C atoms
released as CO2 and the NADH molecule is formed
c. With the joining of pylamine pyrophosphate, lipoatic acid, koash, FAD
and NAD + in the reaction, this enzyme complex is very similar to the
complex pyruvate dehydrogenase, but with some differences
d. This complex is inhibited by ATP, GTP, NADH, Succinil KOA and CA2 +.
e. The product is Succinil KOA is a high-energy tioester compound similar to
the acetyl KOA.
5. Solution of CoA Succinil
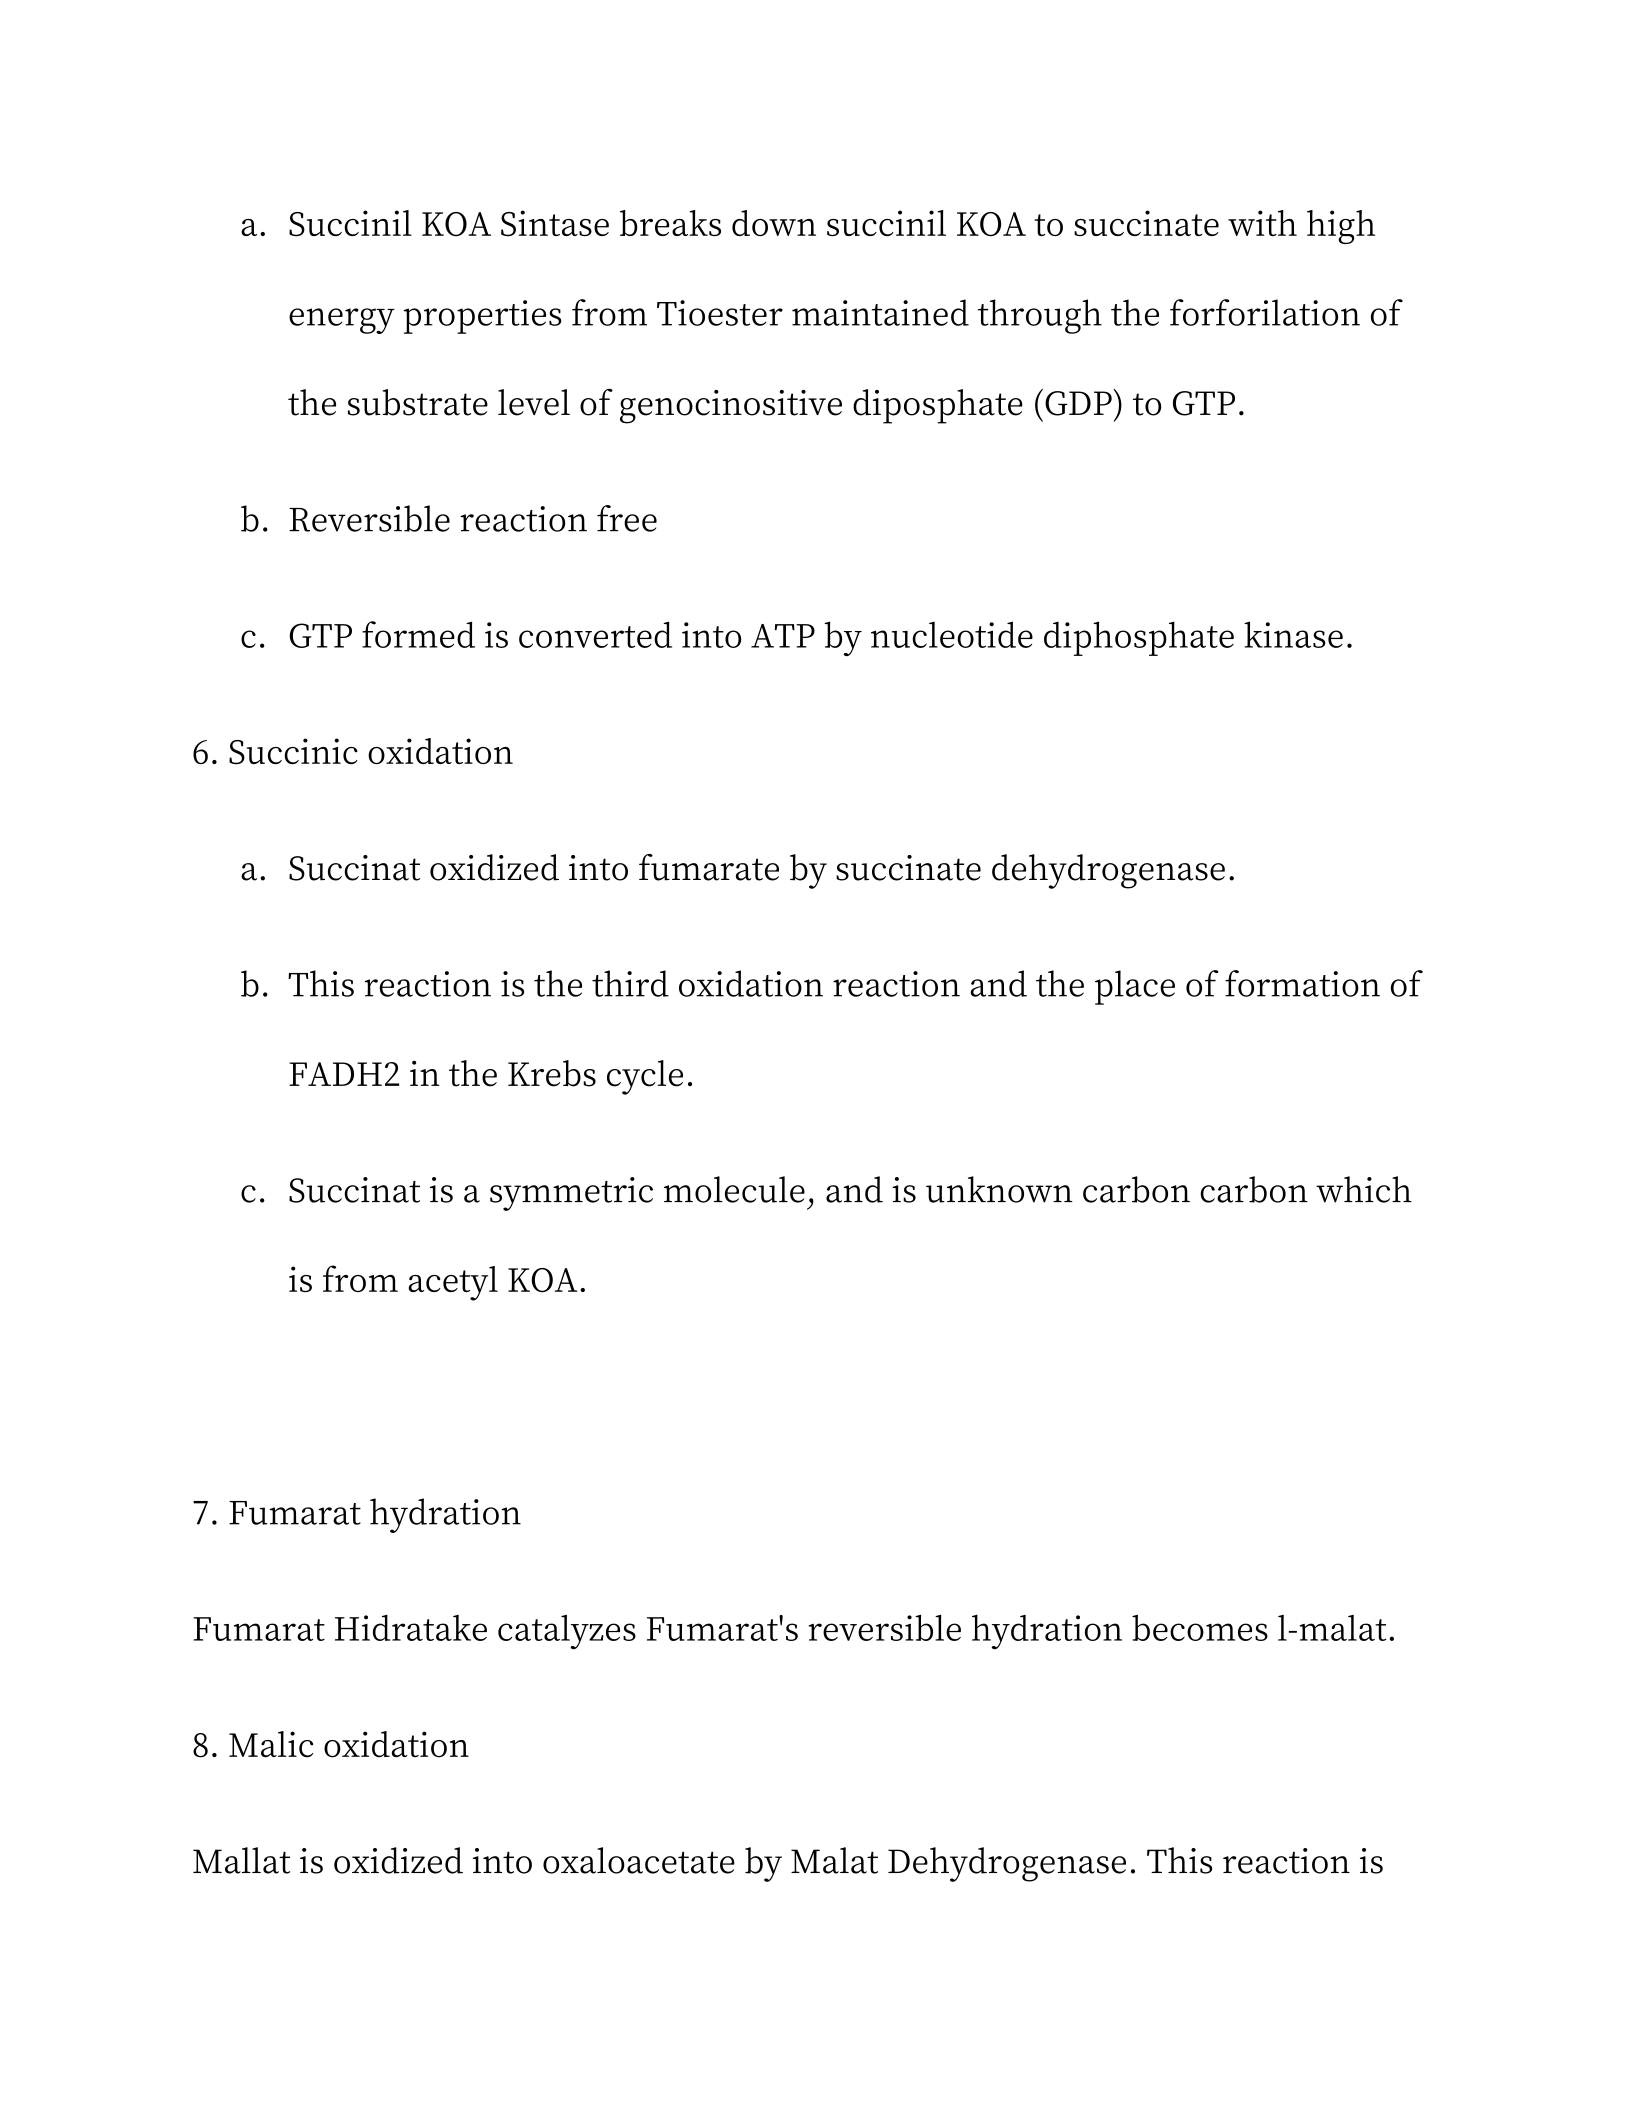
a. Succinil KOA Sintase breaks down succinil KOA to succinate with high
energy properties from Tioester maintained through the forforilation of
the substrate level of genocinositive diposphate (GDP) to GTP.
b. Reversible reaction free
c. GTP formed is converted into ATP by nucleotide diphosphate kinase.
6. Succinic oxidation
a. Succinat oxidized into fumarate by succinate dehydrogenase.
b. This reaction is the third oxidation reaction and the place of formation of
FADH2 in the Krebs cycle.
c. Succinat is a symmetric molecule, and is unknown carbon carbon which
is from acetyl KOA.
7. Fumarat hydration
Fumarat Hidratake catalyzes Fumarat's reversible hydration becomes l-malat.
8. Malic oxidation
Mallat is oxidized into oxaloacetate by Malat Dehydrogenase. This reaction is
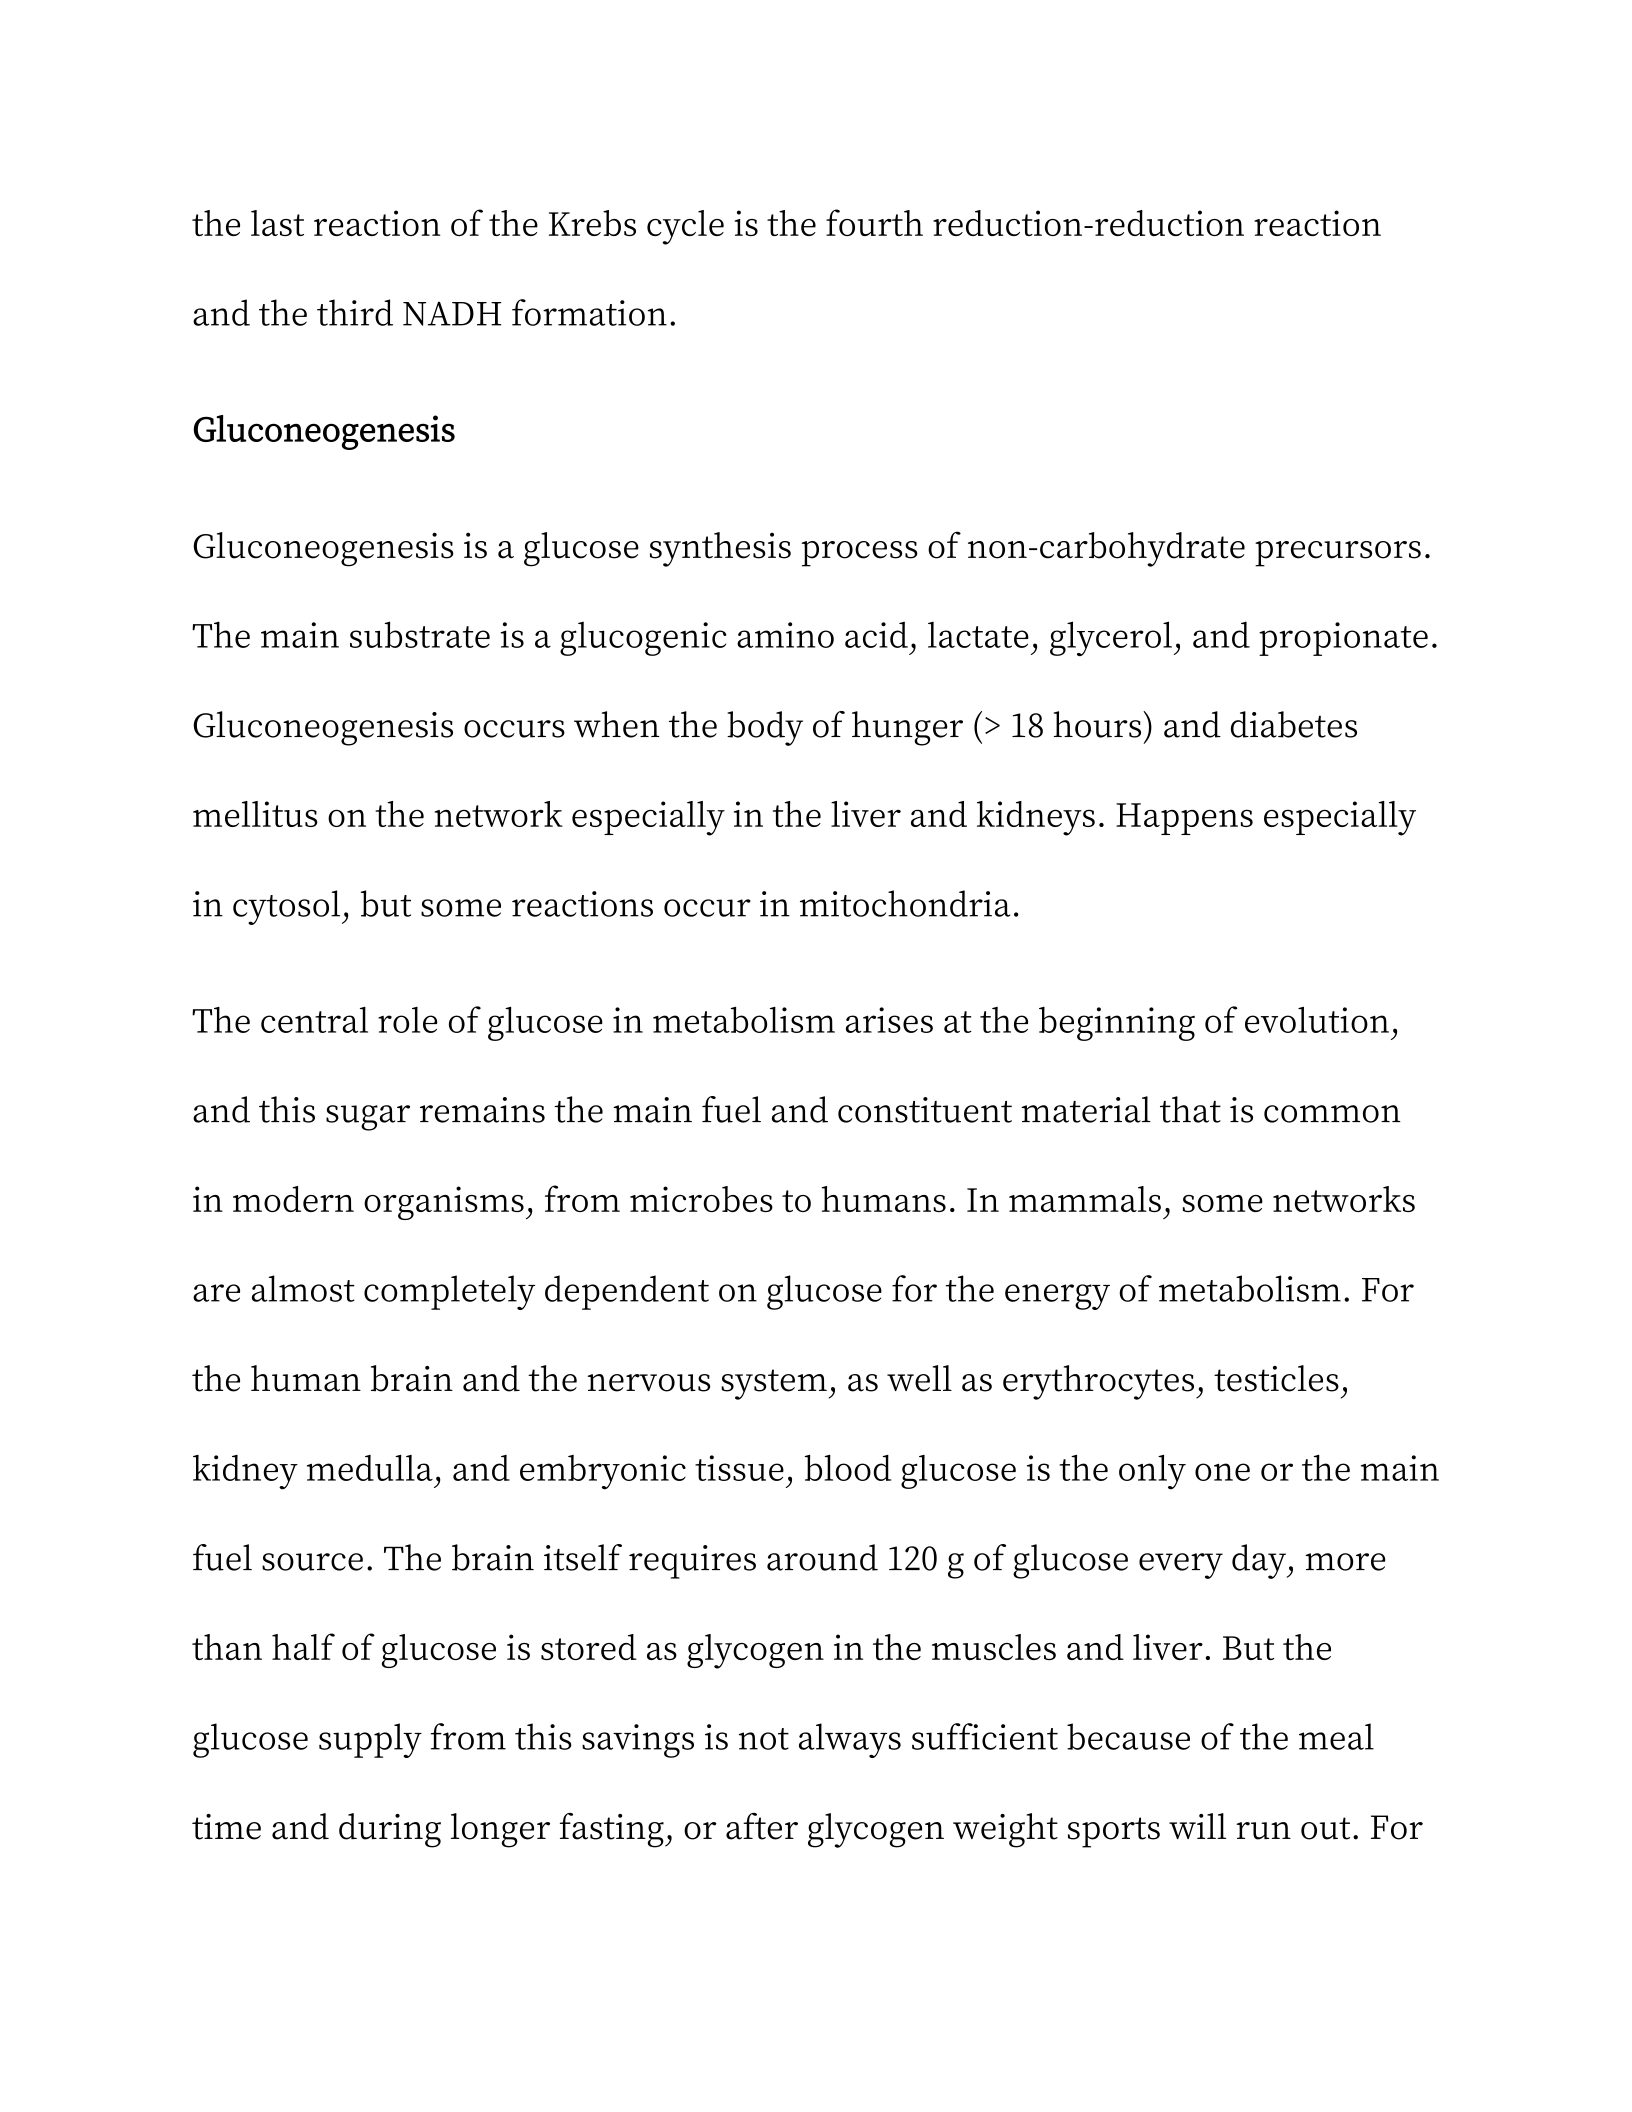
the last reaction of the Krebs cycle is the fourth reduction-reduction reaction
and the third NADH formation.
Gluconeogenesis
Gluconeogenesis is a glucose synthesis process of non-carbohydrate precursors.
The main substrate is a glucogenic amino acid, lactate, glycerol, and propionate.
Gluconeogenesis occurs when the body of hunger (> 18 hours) and diabetes
mellitus on the network especially in the liver and kidneys. Happens especially
in cytosol, but some reactions occur in mitochondria.
The central role of glucose in metabolism arises at the beginning of evolution,
and this sugar remains the main fuel and constituent material that is common
in modern organisms, from microbes to humans. In mammals, some networks
are almost completely dependent on glucose for the energy of metabolism. For
the human brain and the nervous system, as well as erythrocytes, testicles,
kidney medulla, and embryonic tissue, blood glucose is the only one or the main
fuel source. The brain itself requires around 120 g of glucose every day, more
than half of glucose is stored as glycogen in the muscles and liver. But the
glucose supply from this savings is not always sufficient because of the meal
time and during longer fasting, or after glycogen weight sports will run out. For
this reason, organisms need a method for synthesizing glucose from
nonkarbohydrate precursors called gluconeogenesis.
Step - step of the gluconeogenesis line:
1. Change of pyruvate into phosphenol pyruvat [PEP]. Pyruvate will be
dikarboxylated by pyruvate carboxilase into oxaloacetate which is then
converted into PEP through the work of PEP carboxychy.
2. Pep becomes F1.6-DP. PEP changes to F1.6-DP occur through the opposite
path of the glycolysis enzyme, which is set strictly by the levels of substrate and
product.
a. Pep is converted into 2-phosphoglyerates (2-PG) by enolation
b. 2-PG is converted into 3-foffogliserates (3-PG) by 2.3-mutase
phosphoglyerates
c. 3-PG was converted to 1.3 diffosphoglyerates (1.3-DPG) by 1.3-
phosphoglyerating kinase, using one high-energy phosphate bond.
d. 1,3-DPG is converted into 3-phosphate glysticdehyde (G3-P) by
glyceraldehyde 3 phosphate dehydrogenase (G3-PD)
This step requires Nadh Daan to produce NAD + and inorganic phosphate
(PI) as a product /. 1.3 DPG + NADH + H- G3P + NAD + + PI
NADH can come from the reaction of lactic changes to pyruvate, if lactate
is a substrate for gluconeogenesis
Hey. The G3P is in a balance with phosphate (DHAP) dihydroxation (DHAP)
through triosa isomerase and aldolase work, will be converted to F1.6-DP.
3. F1.6-DP Becomes a 6-phosphate Fructose (F6-P).
a. This change cannot be catalyzed by phosphruktokinase which is a
reversible reaction in the condition in cells
b. Liver cells, kidneys and intestinal epithelium containing fructose 1.6
diffosphatase (F1,6-DPAse), which can break down F1.6-DP to F6-P and PI.
This reaction is a slow stage in the sequence of gluconeogenesis reactions,
but it is not the main rate of pace management.
c. FDPase is an alosteric enzyme with ATP as a positive modulator and amp
as a negative modulator
4. F6-P into glucose
a. F6P is converted into glucose 6 phosphate (G6-P) by reversible
phosphoglucoisomerase
b. The formation of free glucose from the G6-P cannot occur through the
reverse reaction of glucokinase or hexocinase
Gluconeogenesis of amino acids
The carbon framework of glucogenic amino acids produces pyruvate formation
or the krebs cycle intermediary which ultimately produces glucose synthesis.
Gluconeogenesis of lactate
Lactic acid is the main final product in the muscles in anaerobic glycolysis.
Muscle tissue is not able to synthesize glucose from lactate. Conversion occurs
all in the heart. Muscle lactate is transported to the heart by blood. At heart, it is
converted into glucose and glycogen by enzymes involved in gluconeogenesis.
The liver glycogen is converted into glucose that is brought back to muscles by
blood. Conversion of muscle lactate into glucose in the liver and re-enter into
the muscles called "Cori Cycle".
Gluconeogenesis of glycerol
With fat hydrolysis, glycerol is released on the adipose network. Glycerol kinase
enzymes contained in the liver and kidneys activate glycerol into 3-phosphate
glycerol which is converted into a phosphate acetone hydroxy by glycerol 3-
phosphate dehydrogenase. Dihidroxy phosphate acetone is an intermediary in
glycolysis and can be easily used for glucose production.
Gluconeogenesis of propionate
Three carbon propionyl KOA is produced by odd chain fatty acid oxidation and
solving some amino acids such as methionine and isoleusin. Propionil KOA KOA
works on this with the presence of ATP and biotin and turns it into methyl
malonil koa which is then converted into succinil KOA with the existence of vit.
Coenzyme B12. Succinil KOA formed from propionyl KOA enters
gluconeogenesis through citric acid cycles
Glikogenesis
Glycogenesis is a process of forming the glycogen of
α
-d-glucose molecules. The
process occurs in cytosol, and requires energy supplied by ATP (for glucose
phosphorylation) and trifosphate uridine (UTP) (Harvey & Ferrier, 2011).
The steps of the inner glycogen synthesis (Harvey & Ferrier, 2011) as in Figure
4.4 consist of;
1. UDP-glucose synthesis
The
α
-d-glucose attached to diffosphate uridine (UDP) is the source of all
glucosyl residues added to the growing glycogen molecules. UDP-glucose is
synthesized from 1-phosphate glucose and UTP by pyrophosphorylase UDP.
High-energy bonds in pyrophosphate (PPI), the second product of the reaction,
hydrolyzed into two inorganic phosphates (PI) by pyrophosphates, which
ensure that the UDP-glucose pyrofosforilage reaction continues towards
production UDP-glucose. 6-phosphate glucose is converted into glucose 1-
phosphate by phosphoglukomutase. 1.6-bisphosphate glucose is a mandatory
intermediary in this reaction.
2. Primary synthesis to start glycogen synthesis
The glycogen synthase is responsible for making
α
(1
→
4) bonds in glycogen.
This enzyme cannot start the synthesis of chains using free glucose as a glucose
molecular acceptor from UDP-glucose. Instead, it can only extend the existing
glucose chain. Therefore, a glycogen fragment can function as a primer in cells
whose glycogen deposits are not exhausted at all. In the absence of glycogen
fragments, the protein called glycogenin can function as a glucose residual
acceptor of the UDP-glucose. The hydroxyl group of side chains from certain
tyrosine serves as a place where the initial glucosil unit is installed. The reaction
is catalyzed by glycogenin itself through autoglukocylation. Thus glycogenin is
an enzyme. Glycogenin then catalyzes the transfer of some of the next glucose
molecules from UDP-glucose, produces a short glucosyl chain connected with
α
(1
→
4). This short chain serves as a primer that can be extended by the glycogen
synthase.
3. Glycogen chain length
Glycogen chain lengthening involves transfers of glucose from UDP-glucose to
the end of the growth chain that does not reduce, form a new glycosidic bond
between carbon anomicically hydroxyl 1 of active glucose and carbon 4 of
glucosyl residues Recipient.
4. Establishment of branches in glycogen
Synthesis of branches carried out by the enzyme branching Amilo
α
(1
→
4)
→
α
(1
→
6) -Trans glucosidase.
Glikogenolisis
Glycogenolysis is a glycogen solving process, occurs in the heart when blood
glucose levels decrease and in the muscles during contractions. The process
occurs in cytosol and this is not the opposite of glycogenesis.
Steps - steps of the glycogenolysis path consist of;
Chain shortening
Glycogen phosphorylase splitting bond
α
(1
→
4) Glycosidat between glucosyl
residue at the end of the noneduction of the glycogen chain with with simple
phosphorolysis so that the four glucosil units remain in every chain in front of
the branching point.
Branches
Branches are discarded by two enzyme activities. First Oligo-
α
(1
→
4)
α
(1
→
4) -
Awry the transferase throw away three outermost glucosyl residues of four
glucosyl residues attached to a branch. Furthermore, the enzyme transfers three
of the outermost glucosil residues to the end of the end of the other chain and
extend it accordingly. The result of the
α
(1 bond
→
4) Disconnected and balance
α
(1
→
4) formed. Furthermore, the single glycose residue that is left behind is
connected to an
α
(1 bond
→
6) Screened hydrolylyly by Akitivity amylo-
α
(1
→
6) -
Glucosidase, which releases free glucose.
Glucose 1 phosphate becomes glucose 6 phosphate
Glucose 1 phosphate produced by glycogen phosphorylase is changed in cytosol
to glucose 6 phosphate by phosphoglukomutase. A reaction that produces
glucose 1.6 bisphosphate as a substance between temporary but essential. In the
heart of glucose 6-phosphate is transferred into the endoplasmic reticulum (Re)
by glucose 6-phosphate translocase. The resulting glucose was then moved out
of Re to the cytosol. Hepatocytes issue glucose from glycogen into the blood to
help maintain blood glucose levels to the gluconeogenesis path producing
glucose actively.

