


INSTRUCTIONS
Length of assignment: Minimum length is 3 pages.
*Each of the 6 sections (explained below) must contain no fewer than 100
words.
*Format: The assignment must be double spaced using Times New
Roman font in size 12 and written in APA format.
*Citations: No additional citations other than the article chosen to review
is required.
*Acceptable sources: Each article must be a primary research study
published within the last 10 years in a peer-reviewed research journal.
*Important: Article Review assignment must contain the following:
I.The article title, author(s), journal title, volume, issue, year, and page
numbers, all written in current APA format.
II.Include the following 6 sections (include section headings, do not
include instructions).
a. Objectives: Include background information on the topic and the goal
or purpose of the article.
b. Methods:Include how many subjects participated (male/female, age,
medical history if applicable), what biomechanical tools were used in the
study, and what statistics were used by the author(s).
c. Results: Explain key observations and/or findings in the article.
d. Summary:Include a synopsis of the discussion and conclusions of the
article and was free of direct quotes.
e. Critique:Include an opinion, explanation, and biblical integration.
III. Question/Application: This section must include 1 question pertaining
to how the article relates to another research article performed on the
research topic. Secondly, provide two facts you have learned from your
article review that would be interesting to share with a coach or a
clinician who is an expert in their field.
ORIGINAL RESEARCH
published: 08 August 2019
doi: 10.3389/fbioe.2019.00193
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 1August 2019 | Volume 7 | Article 193
Edited by:
Veronica Cimolin,
Politecnico di Milano, Italy
Reviewed by:
Francesco Travascio,
University of Miami, United States
Andrew D. Nordin,
University of Florida, United States
*Correspondence:
Emily J. Cushion
emily[email protected]
Daniel J. Cleather
Specialty section:
This article was submitted to
Biomechanics,
a section of the journal
Frontiers in Bioengineering and
Biotechnology
Received: 20 December 2018
Accepted: 24 July 2019
Published: 08 August 2019
Citation:
Cushion EJ, Warmenhoven J,
North JS and Cleather DJ (2019)
Principal Component Analysis Reveals
the Proximal to Distal Pattern in
Vertical Jumping Is Governed by Two
Functional Degrees of Freedom.
Front. Bioeng. Biotechnol. 7:193.
doi: 10.3389/fbioe.2019.00193
Principal Component Analysis
Reveals the Proximal to Distal
Pattern in Vertical Jumping Is
Governed by Two Functional Degrees
of Freedom
Emily J. Cushion 1
*, John Warmenhoven 2, Jamie S. North 1and Daniel J. Cleather 1
*
1Faculty of Sport, Health and Applied Science, St Mary’s University, Twickenham, United Kingdom, 2Exercise and Sports
Science, Faculty of Health Sciences, The University of Sydney, Lidcombe, NSW, Australia
The successful completion of motor tasks requires effective control of multiple degrees
of freedom (DOF), with adaptations occurring as a function of varying performance
constraints. In this study we sought to compare the emergent coordination strategies
employed in vertical jumping under different task constraints [countermovement jump
(CMJ) with arm swing-CMJas and no arm swing-CMJnas]. In order to achieve this,
principal component analysis (PCA) was conducted on joint moment waveform data
from the hip, knee and ankle. This statistical approach has the advantage of analyzing
the whole movement within a time series and reduces multidimensional datasets to
lower dimensions for analysis. Both individual and group analyses were conducted.
For individual analysis, PCA was conducted on combined hip, knee, and ankle joint
moment data for each individual across both CMJnas (thirty-eight participants), and
CMJas (twenty-two participants) conditions. PCA was also performed comparing all
data from each individual across CMJnas and CMJas conditions. The results revealed a
maximum of three principal components (PC) explained over 90% of the variance in the
data sets for both conditions and within individual and group analyses. For individual
analysis, no more than 2PCs were required for both conditions. For group analysis,
CMJas required 3PCs to explain over 90% of the variance within the dataset and CMJnas
only required 2PCs. Reconstruction of the original NJM waveforms from the PCA output
demonstrates a greater loading of hip and knee joint moments to PC1, with PC2 showing
a greater loading to ankle joint moment. The reduction in dimensions of the original data
shows the proximal to distal extension pattern in the sagittal plane, typical of vertical
jumping tasks, is governed by only 2 functional DOF, at both a group, and individual
level, rather than the typically reported 3 mechanical DOF in some forms of jumping.
Keywords: principal component analysis, vertical jumping, degrees of freedom, constraints, proximal to distal
pattern
Cushion et al. PCA of Vertical Jumping
INTRODUCTION
In both day-to-day and sporting contexts, human
beings consistently perform complex motor actions. Whether
this is walking up and down flights of stairs at home or
performing jumping actions in sport, people are able to perform
such skills with relative ease. Yet underpinning these observable
actions is a need to coordinate and control multiple degrees
of freedom (DOF), referred to as “the degrees of freedom
problem” by Bernstein (1967). With so many DOF within
the motor system, there are an almost limitless number of
coordination patterns available to the performer. However,
according to theoretical principles from ecological psychology,
and dynamical systems theory, it is proposed that the performer
seeks to satisfy the goal of the task whilst operating under
continually interacting task, environmental, and organismic
constraints, through which coordinated patterns of behavior
emerge (Newell, 1986; Hristovski et al., 2006; Orth et al., 2018).
Critical, therefore, in successfully completing such tasks is the
need to control the “redundant” DOF (Bernstein, 1967; Latash,
2000). These “redundant” DOF, however, provide important
functionality as they enable adaptation of emerging actions
to the varying performance constraints under which they are
operating. For example, Chow et al. (2008) demonstrated that
participants adapted their use of limb segments to continue
successfully performing a soccer chipping task whilst the task
constraints (which we define here as goals or rules which are
imposed that influence the movement) were manipulated.
Such a finding evidences how the redundant DOF allow for
functional variability and for performers to adapt to ever
changing performance constraints. Whilst there has been much
work within this area it is common for only kinematic changes
under varying constraints to be considered (e.g., Ketcham et al.,
2002; Seifert et al., 2007; Majed et al., 2017). However, analyzing
kinetic factors, such as forces and joint moments, would provide
a more complete understanding of how emerging behaviors are
shaped as a function of the task constraints under which the skill
is performed.
Explaining the control strategies adopted by performers has
been a topic within the motor control literature for many
years (see Dufek et al., 1995; Bates, 1996; James and Bates,
1997; James et al., 2003, 2014; Nordin and Dufek, 2019). It
has been suggested that certain movement features are more
important to satisfy the goal of the task, and therefore these
features are less likely to show variance between repetitions
or from person to person (Scholz and Schoner, 1999; Scholz
et al., 2000). This has been demonstrated using several tasks
(see Button et al., 2003; Seifert et al., 2011; Nordin et al.,
2017). For instance, elbow angle at ball release in a basketball
shooting task showed lesser variability between individuals of
varying skill levels, compared to other features such as wrist
angle at ball release (Button et al., 2003), which indicates that
elbow angle at ball release is an important movement feature
for successful performance in this task. Identification of such
movement features aids in developing our understanding of
motor control strategies employed to govern movements under
varying task constraints.
Traditional approaches to the study of human movement
have typically relied on selecting discrete data points for
analysis. However, these methods may not provide a complete
representation of the complexities of motor actions due to
data being discarded outside of those discrete points. Instead,
methods which analyse data across the full temporal cycle of the
movement, such as principal component analysis (PCA), may
prove more informative (Richter et al., 2014). The attraction
of PCA is that large amounts of data across movement cycles
can be analyzed whilst reducing the dimensionality of data to
features of importance (Daffertshofer et al., 2004). This statistical
approach has been used to determine key characteristics of
movement tasks (see for example Soechting and Flanders, 1997;
Kollias et al., 2001; Lamoth et al., 2006; Dona et al., 2009;
Witte et al., 2010; Federolf et al., 2013; Nordin and Dufek,
2016a) as well as determining similarities and differences between
groups through data filtering (see for example Deluzio et al.,
1997; Deluzio and Astephen, 2007; Laffaye et al., 2007; Lee
et al., 2009; Federolf et al., 2013; Verrel et al., 2013). Despite
the growth of PCA in sports sciences recently, its application
is still in its relative infancy. In particular, fewer researchers
have used this approach to determine coordination patterns
within movements or to compare movements under differing
task constraints (see Forner-Cordero et al., 2005; Lee et al.,
2009; Nordin and Dufek, 2016b; Majed et al., 2017 for some
exceptions). Therefore, applying a statistical approach such as
PCA can be useful in reducing large datasets to key movement
features and may be more effective in showing how movement
emerges under changing constraints.
Vertical jumping is an interesting motor task to study as
it requires the effective coordination of the upper and lower
limbs to raise the center of mass vertically, with a clear goal
of jumping for height (Raffalt et al., 2016). Vertical jumping
also represents a task which can be easily manipulated to
provide insight into how emergent behaviors adapt to differing
conditions. Analysis of movements under constrained conditions
can lead to a better understanding of the key mechanisms for
efficient movement, such as the requirement to keep balance in
a sit to stand task (Scholz et al., 2001) or the accommodation
strategies with increased task demands (Nordin and Dufek,
2016b, 2017). With this in mind, this study used a vertical
jumping task and asked participants to complete this action
under two different task constraints (with arm swing and without
arm swing), with the aim of understanding how motor control
strategies, and emergent coordination patterns were affected
by manipulation of these constraints. To fully understand
these coordination strategies and overcome the limitations
associated with traditional analysis methods, we employed PCA
to determine the principal components (PCs) that characterize
vertical jumping movement patterns both between and within
individuals and across the two task constraints. Specifically, we
aimed to answer the question of the number of PCs expected
to describe either a single jump, repetitions of a jump from an
individual, and across the whole group. Typically, lower limb
coordination in jumping tasks is described as an extension of
the lower limbs in a proximal to distal fashion, with the peak
moment progressing temporally from hip, to knee, and then
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 2August 2019 | Volume 7 | Article 193
Cushion et al. PCA of Vertical Jumping
ankle (Bobbert and van Ingen Schenau, 1988). A moment curve
is typically bell-shaped and unimodal (examples can be seen in
Figures 6,7). If the timing of peak moments and the shape of
the moment curves are independent of one another it would be
expected that 3 PCs would be required to represent the 3 moment
curves of a particular jump (that is 3 functional DOF). If the peaks
of the 3 moment curves occur at different time points along the
curve, then there needs to be more than one PC score.
MATERIALS AND METHODS
Participants
Thirty-eight healthy individuals (males =24, females =14)
volunteered to take part in this study (mean ±SD; age =
27 ±5 years, height =174.4 ±9.0 cm, body mass 78.1 ±
14.1 kg). Participants were free from musculoskeletal injuries and
were provided with details of the study before written informed
consent was obtained. The experimental procedure was approved
by the ethics sub-committee at the institution where the research
took place.
Procedure
Participants were required to attend one data collection session.
This involved the collection of anthropometric measures (height
and weight), before each participant was provided with a
standardized shoe according to their shoe size. Eighteen
reflective markers were placed on the pelvis and on the right
lower limb. Data from the right limb was used for further
analysis in accordance with previous work from Cleather et al.
(2013). Markers were placed on the right and left anterior
superior iliac spine and posterior superior iliac spine, lateral
and medial femoral epicondyle, apex of lateral and medial
malleolus, posterior aspect of calcaneus, tuberosity of fifth
metatarsal, and head of second metatarsal. Three additional
markers placed on rigid plates were attached to the mid-
thigh and anterior tibial shaft, with an additional marker
attached to the top of the foot. Kinematic data was collected
using a Vicon motion capture system (Vicon MX System,
Nexus 2.2 software, Vicon Motion Systems Ltd, Oxford, UK)
with 14 LED cameras tracking the reflective markers at a
sampling frequency of 200 Hz. Kinetic data was collected via
two force plates positioned flush to the laboratory floor (Kistler
Type 9287BA, Bioware 3.24 software, Kistler Instruments Ltd,
Hampshire, UK), at a rate of 1,000 Hz and synchronized with the
Vicon system.
Participants completed a standardized warm-up (bodyweight
squats, lunges, inchworms, hip rotations, and vertical jumps)
prior to completing any vertical jumps. Thirty-eight participants
performed a vertical jump task (countermovement jump with no
arm swing—CMJnas). For this task, participants were instructed
to keep hands in contact with the hip throughout the jump,
and to land with one foot on each force plate. Participants were
required to complete five maximal effort trials with a self-selected
recovery period between each jump to reduce any effects of
fatigue. Twenty-two of the participants carried out an additional
jumping task. For this task, participants performed a vertical
jump with the use of an arm swing (CMJas). Participants were
instructed to use an arm swing to aid in jumping performance
and were required to land with one foot on each force plate. For
these participants the order of completion of the two tasks was
counterbalanced to prevent order effects. Participants were given
a 2 min recovery period between the two tasks.
Data Analysis
All data was filtered using a 5th order Woltring filter with a
cut off frequency of 10 Hz. The propulsive phase of the vertical
jump was used for analysis and was defined as being from
the point where the right anterior superior iliac spine marker
moved below stationary height until take-off (which was defined
as the point where the ground reaction force fell to zero).
Net joint moments (NJM) in the sagittal plane were calculated
for hip, knee, and ankle during this phase using a standard
inverse dynamics calculation (Winter, 2005) within the FreeBody
software (Cleather and Bull, 2015). Each jump trial therefore had
the 3 mechanical DOF described by the NJM.
As trial length varied across each participant, data was spline
interpolated and time normalized from 0 to 101 data points.
Maximal jump height was analyzed through calculation of the
change in displacement of the right anterior superior iliac spine
when standing, to the maximum height achieved during the jump
(Chiu and Salen, 2010).
PCA Calculation
PCA was used in this study to extract common patterns of
moment production during the vertical jump under two task
constraints. Using this approach has the advantage of retaining
the spatiotemporal pattern in the time series data whilst detecting
coordination patterns both within and between individuals. The
fundamental purpose of a PCA is to find a linear transformation
that maps the raw data described in its original coordinate
frame to a new coordinate frame with orthonormal bases. In
the context of data analysis, the coordinate frame for the raw
data is defined by the measured variables, but these variables
may have some degree of correlation with one another. The
new coordinate frame that is given by the PCA will be defined
by a set of new uncorrelated variables called the principle
components (PC). For instance, for a dataset consisting of p
variables observed at ndifferent time-points the raw data can
be described by the n×pmatrix Xwhere the columns of
Xare the individual variables, and the rows represent each
observation (time-point). The transformation Uthen maps the
raw data to the new coordinate frame defined by the PCs,
such that the raw data in the new coordinate frame Z, is given
by Z=XU.
In biomechanics, PCA has sometimes been used to compare
time-normalized waveforms. For instance, a waveform can be
described by the value of a variable sampled at 1% intervals over
the course of a movement. Typically, we have multiple waveforms
(cases) for one particular biomechanical variable which we want
to compare—for instance, if we want to compare the curves
of different individuals. In this instance, as outlined extensively
in Deluzio and Astephen (2007), the individual time-points
have often been considered as variables and cases (observations)
considered to be the individual curves being analyzed. Thus if
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 3August 2019 | Volume 7 | Article 193
Cushion et al. PCA of Vertical Jumping
we had pdifferent curves for a given variable, that each consists
of 101 time-points, we would perform the PCA on the p×101
raw data matrix XT. In the present study we have adopted a
more intuitive approach to study waveforms that is closer to
the traditional description of PCA. We have treated the time
normalized intervals as observations, and the individual curves
(cases) as variables. Thus, for our pdifferent curves for a given
biomechanical variable sampled at 101 time-points we perform
the PCA on the 101 ×praw data matrix X. This approach has
been used previously (see Borzelli et al., 1999).
It should be noted that in the method of Deluzio and Astephen
(2007), a separate PCA is performed for each of the measured
variables. In contrast, in this study we have included all of
the measured variables within the same PCA. For instance, in
this study, for an individual subject we have time-series for 3
biomechanical variables (hip, knee, and ankle NJM) measured in
5 different jumps. Using the method of Deluzio and Astephen
(2007) we would perform 3 PCAs on the 3 5 ×101 matrices
representing each joint. Instead, in this study we perform only
one PCA on the 101 ×15 matrix which includes all of the
individual’s data.
One common application of PCA is to reduce the
dimensionality of the data being analyzed—that is to reduce the
number of variables under consideration to a smaller set which
describe the majority of the variance in the data. The advantage
of the method we have adopted here is that the coordinate frame
in which the data is described is defined by all of the cases for all
of the measured joints (NJM). This means that the PCA produces
a reduced new coordinate frame that can be used to describe
all cases and joints. This therefore means that the reduced
coordinate system represents the number of functional degrees
of freedom that are present in the movement being analyzed.
Conventional approaches to using PCA would require each
variable (e.g., hip NJM, knee NJM, ankle NJM) to be analyzed
separately. This would limit the ability to effectively interpret the
functional DOF describing the movements. Thus, for the present
study PCA was used in this manner to extract common patterns
of moment production during the vertical jump under two task
constraints. Only those PCs that cumulatively explained over
90% of the variance in the data set were retained and used in
further analysis (Jolliffe, 2002).
Prior to running the PCA, all data was normalized to the
peak hip joint moment of each trial (Jolliffe and Cadima, 2016).
Analysis of the data was performed on both an individual (termed
analysis 1), and group (termed analysis 2) basis (as has previously
been conducted within the literature, e.g., Nordin and Dufek,
2016a,b, 2017) and the PCs from the individual (PCi), and group
(PCg) analyses are indicated by subscripts as shown. For the
individual analysis a PCA was carried out for each individual
separately, which contained hip, knee and ankle NJM data
combined (101 ×15 matrix for each individual containing 15
columns representing 5 hip, 5 knee, and 5 ankle joint moment
time series with 101 data points). This was performed for both
CMJnas and CMJas conditions. For the group analysis, all NJM
data from each participant were combined and subjected to a
PCA (CMJnas: 101 data points ×567 joint moment time series,
CMJas: 101 data points ×330 joint moment trials). A further
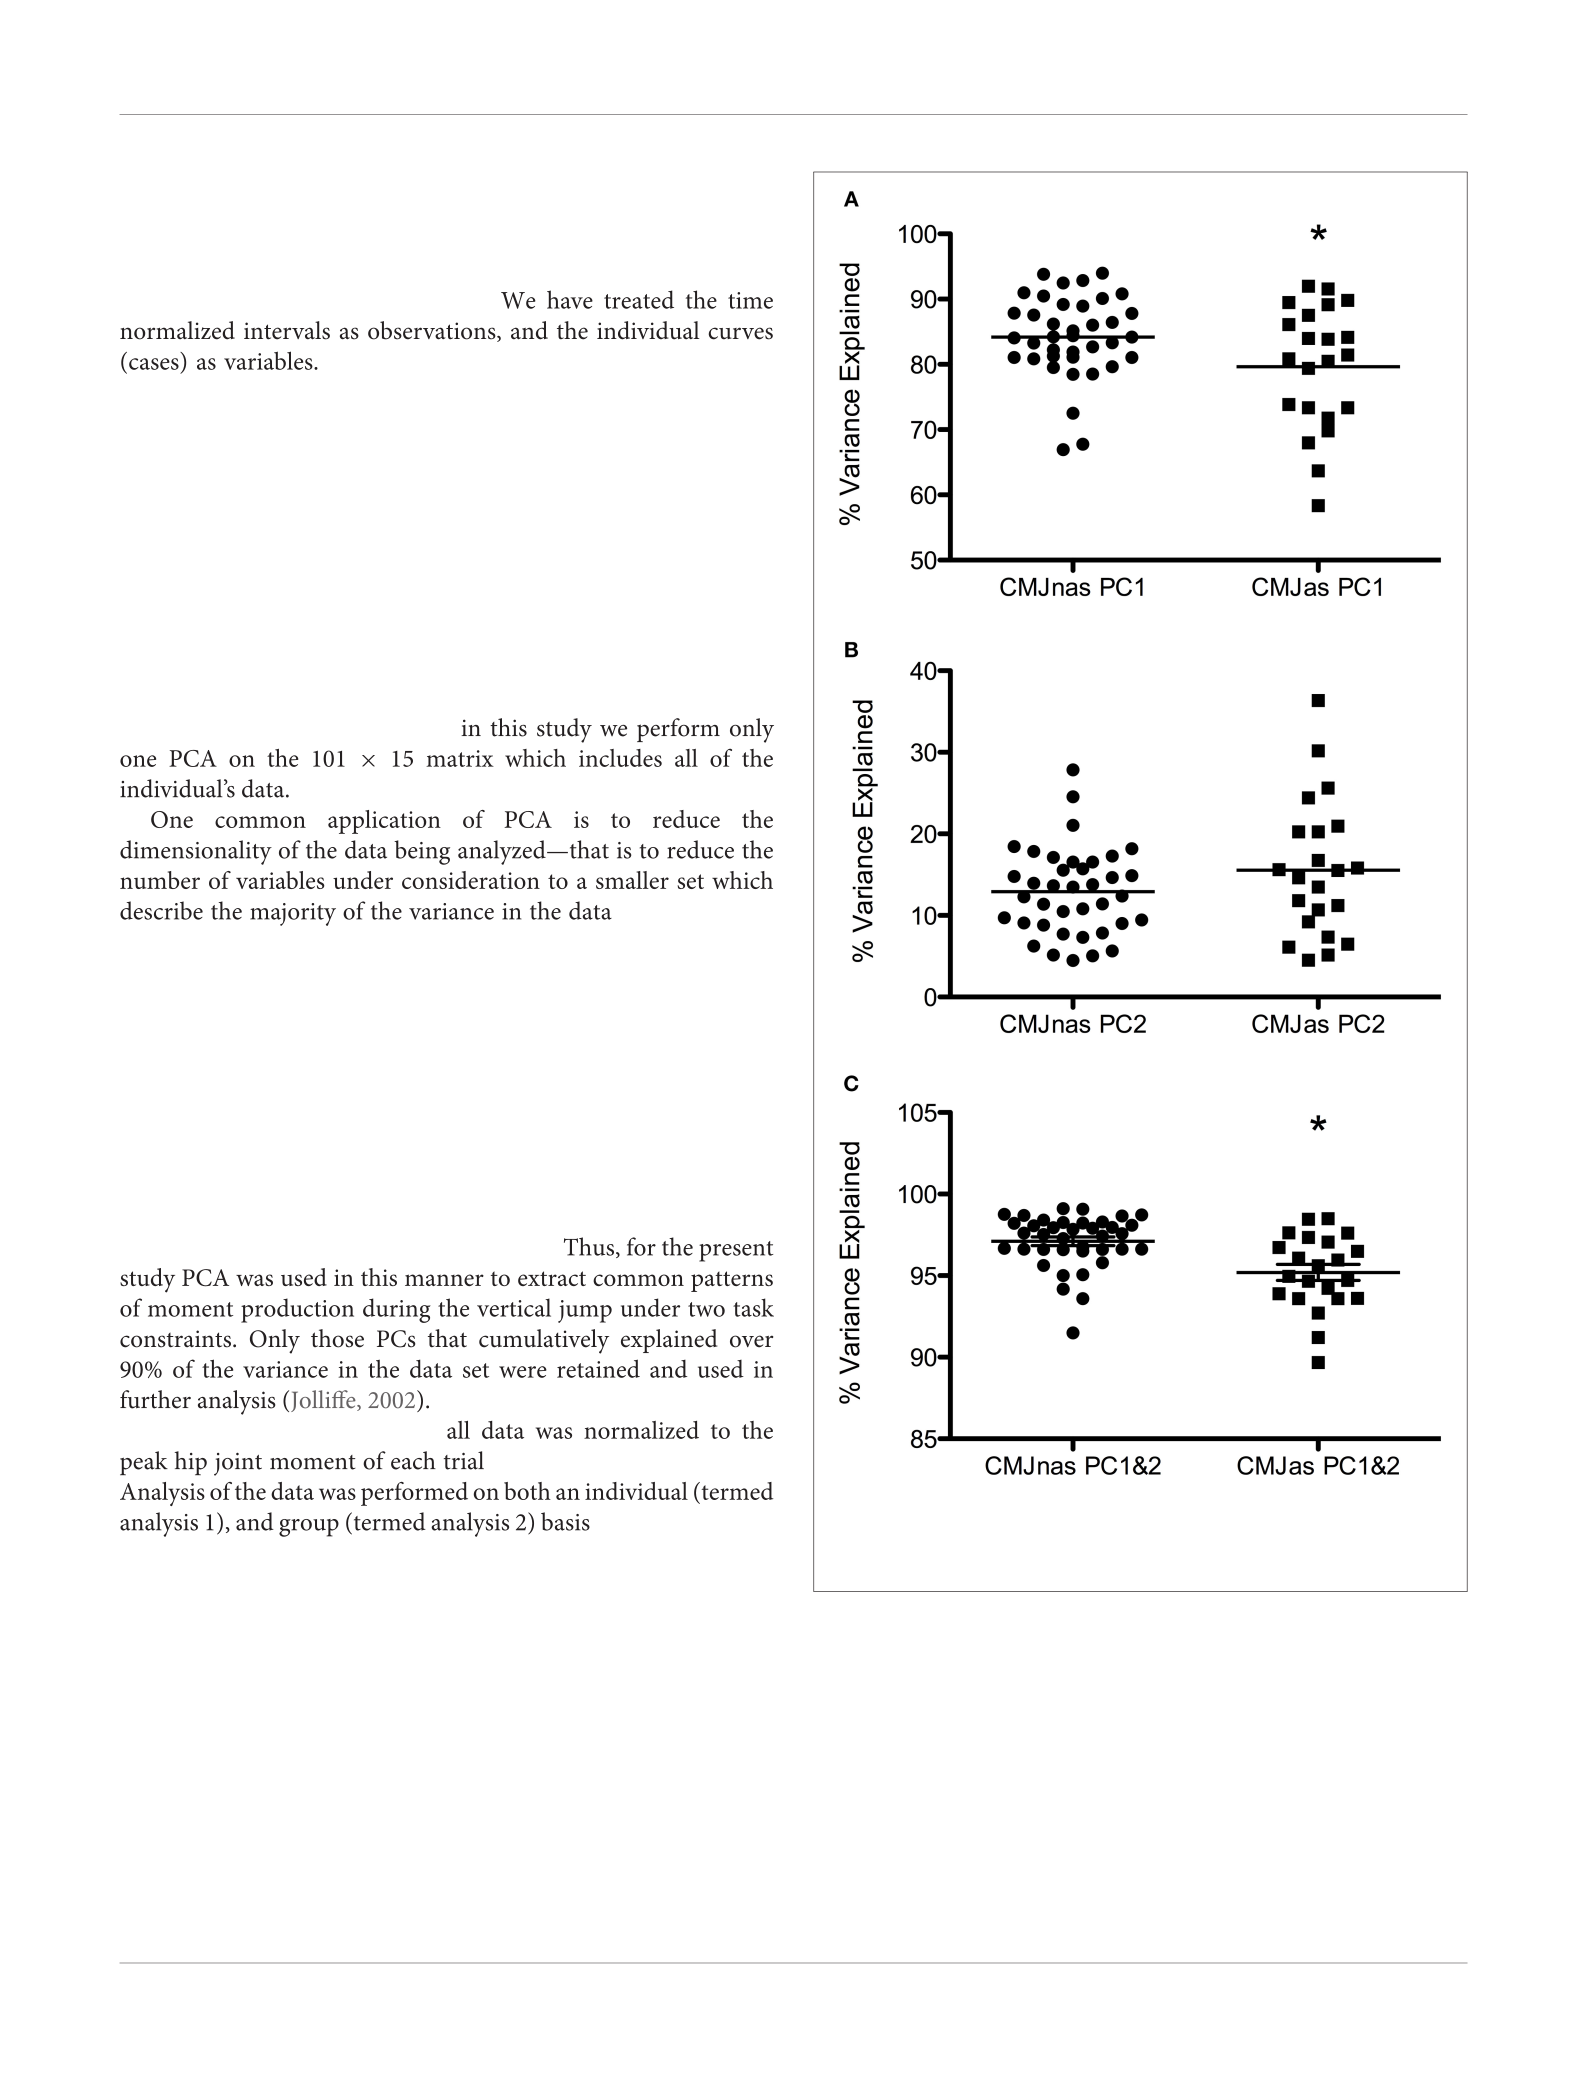
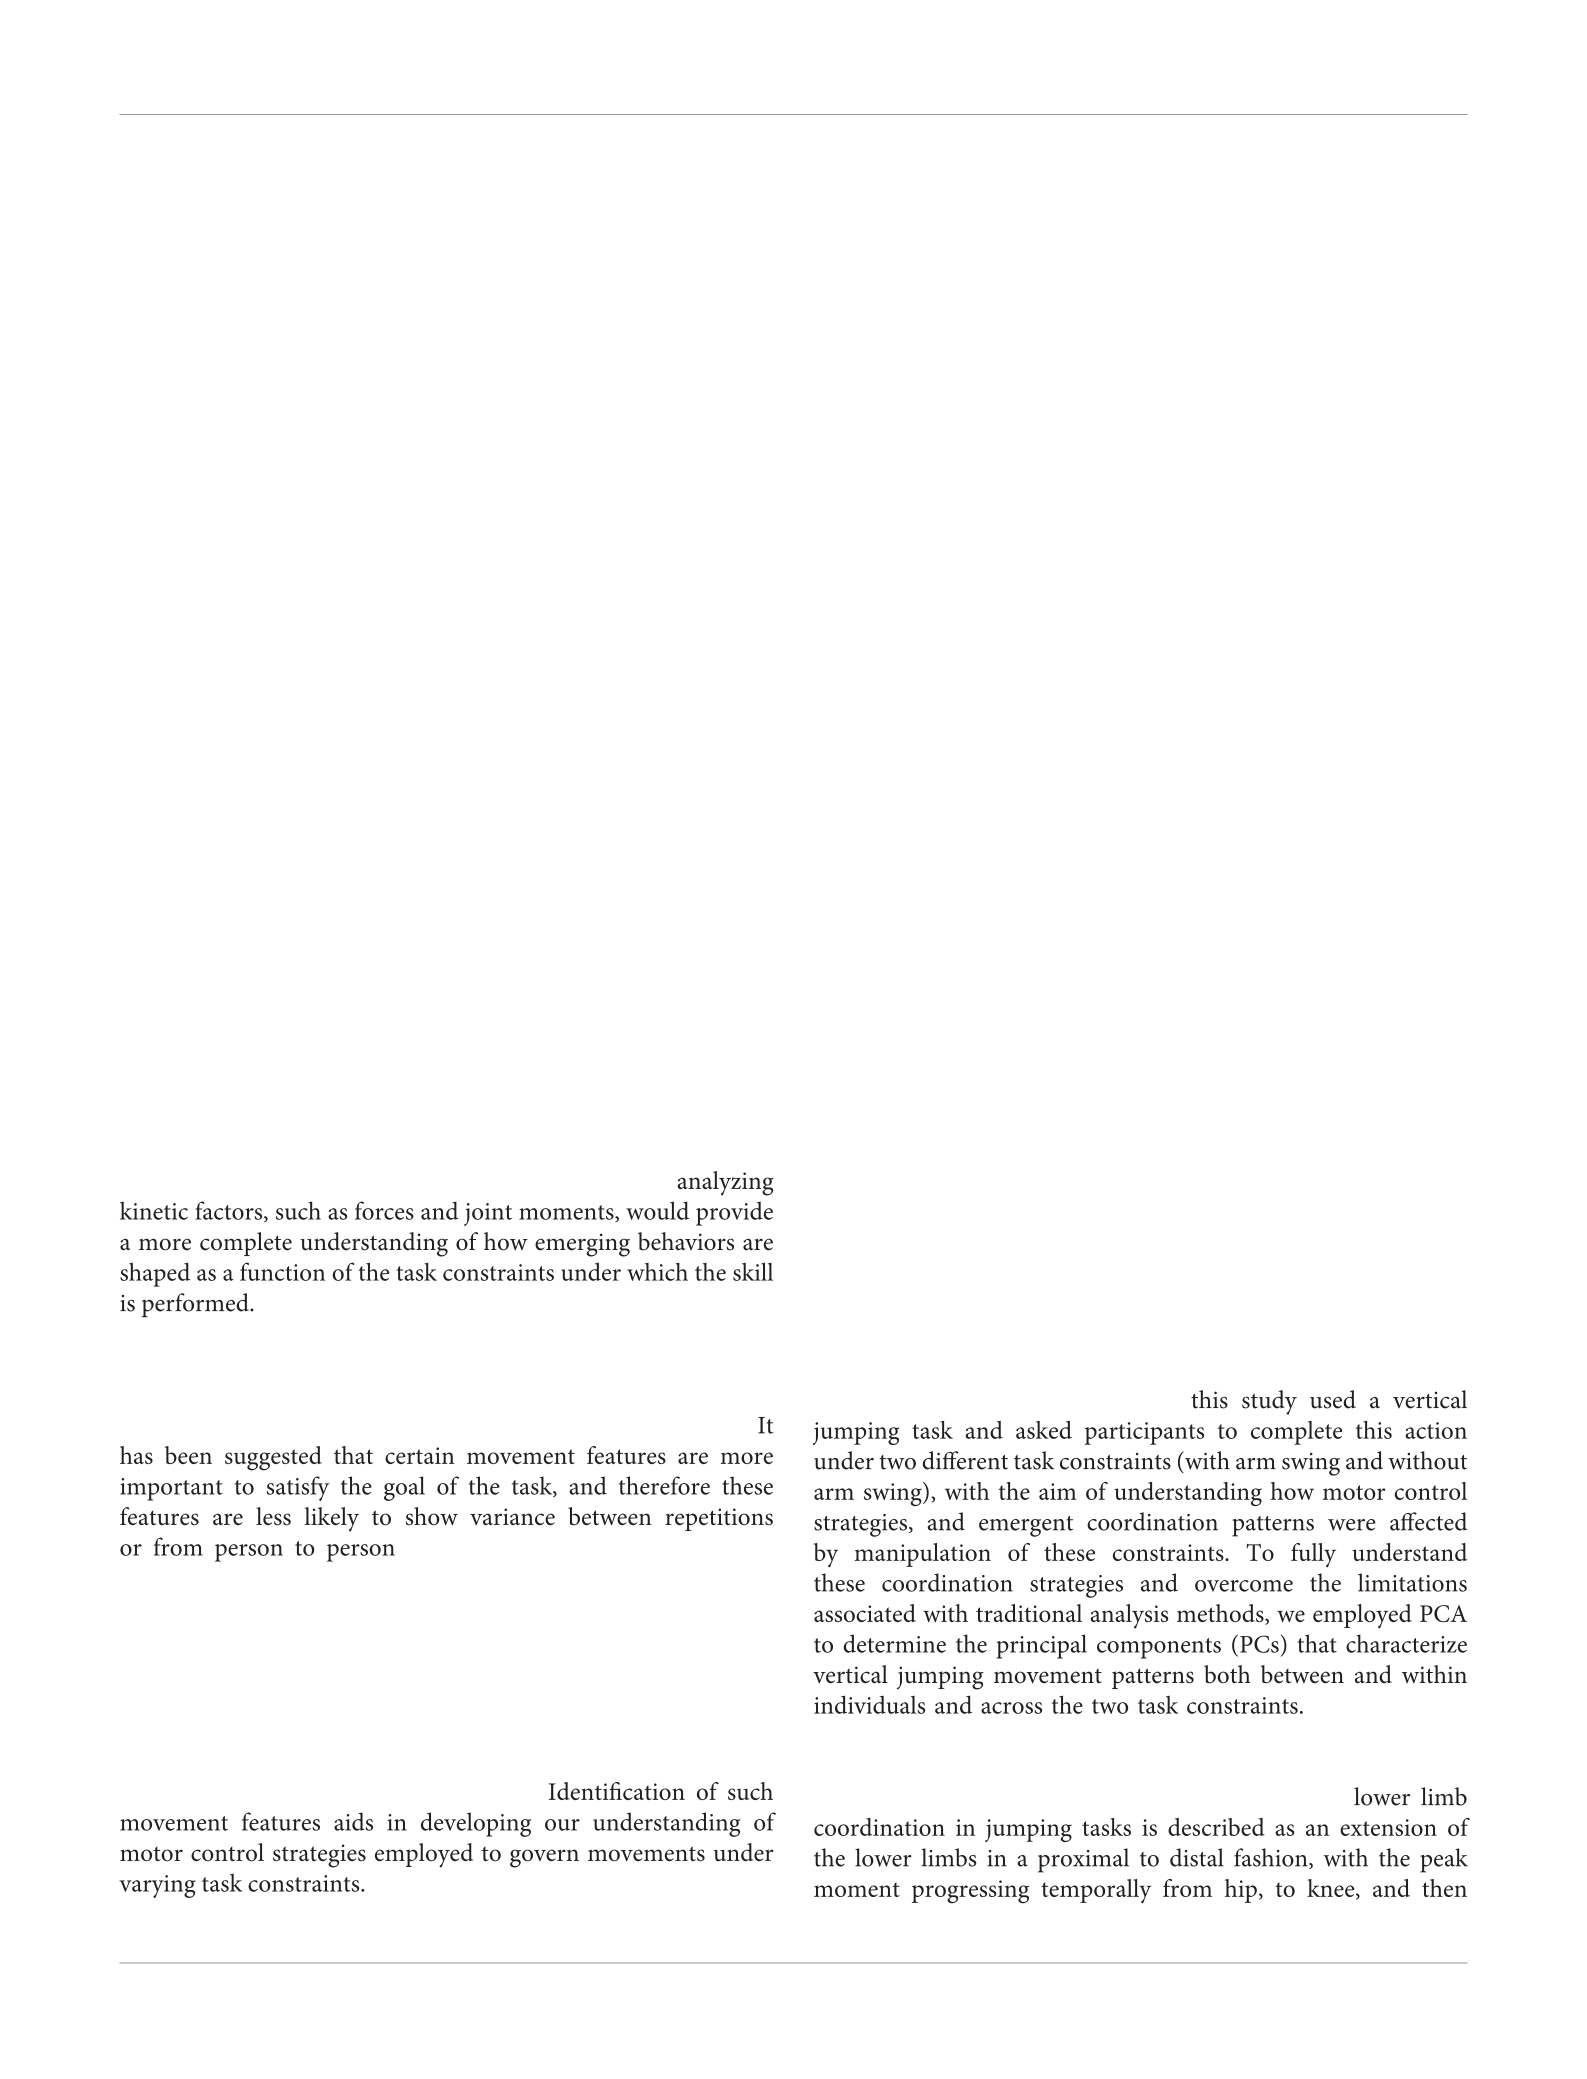
FIGURE 1 | Variance explained by (A) PC1i, (B) PC2i, and (C) the sum of
PC1i&2i for CMJnas, and CMJas. Horizontal line represents group mean.
i=individual PCA analysis. *Indicates significant difference from CMJnas.
PCA was performed to compare CMJnas and CMJas data with
only the participants who had performed both jumps (101 data
points ×672 joint moment time-series). This is referred to as
analysis 3. Finally, an additional group level PCA was conducted
using only the first 2 PCs obtained from the individual PCA
(CMJnas: 101 data points ×76 PCs, CMJas: 101 data points ×
44 PCs; hereafter called analysis 4).
The output of each PCA was a matrix (henceforth named
the coefficients matrix) where each column gives the coefficients
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 4August 2019 | Volume 7 | Article 193
Cushion et al. PCA of Vertical Jumping
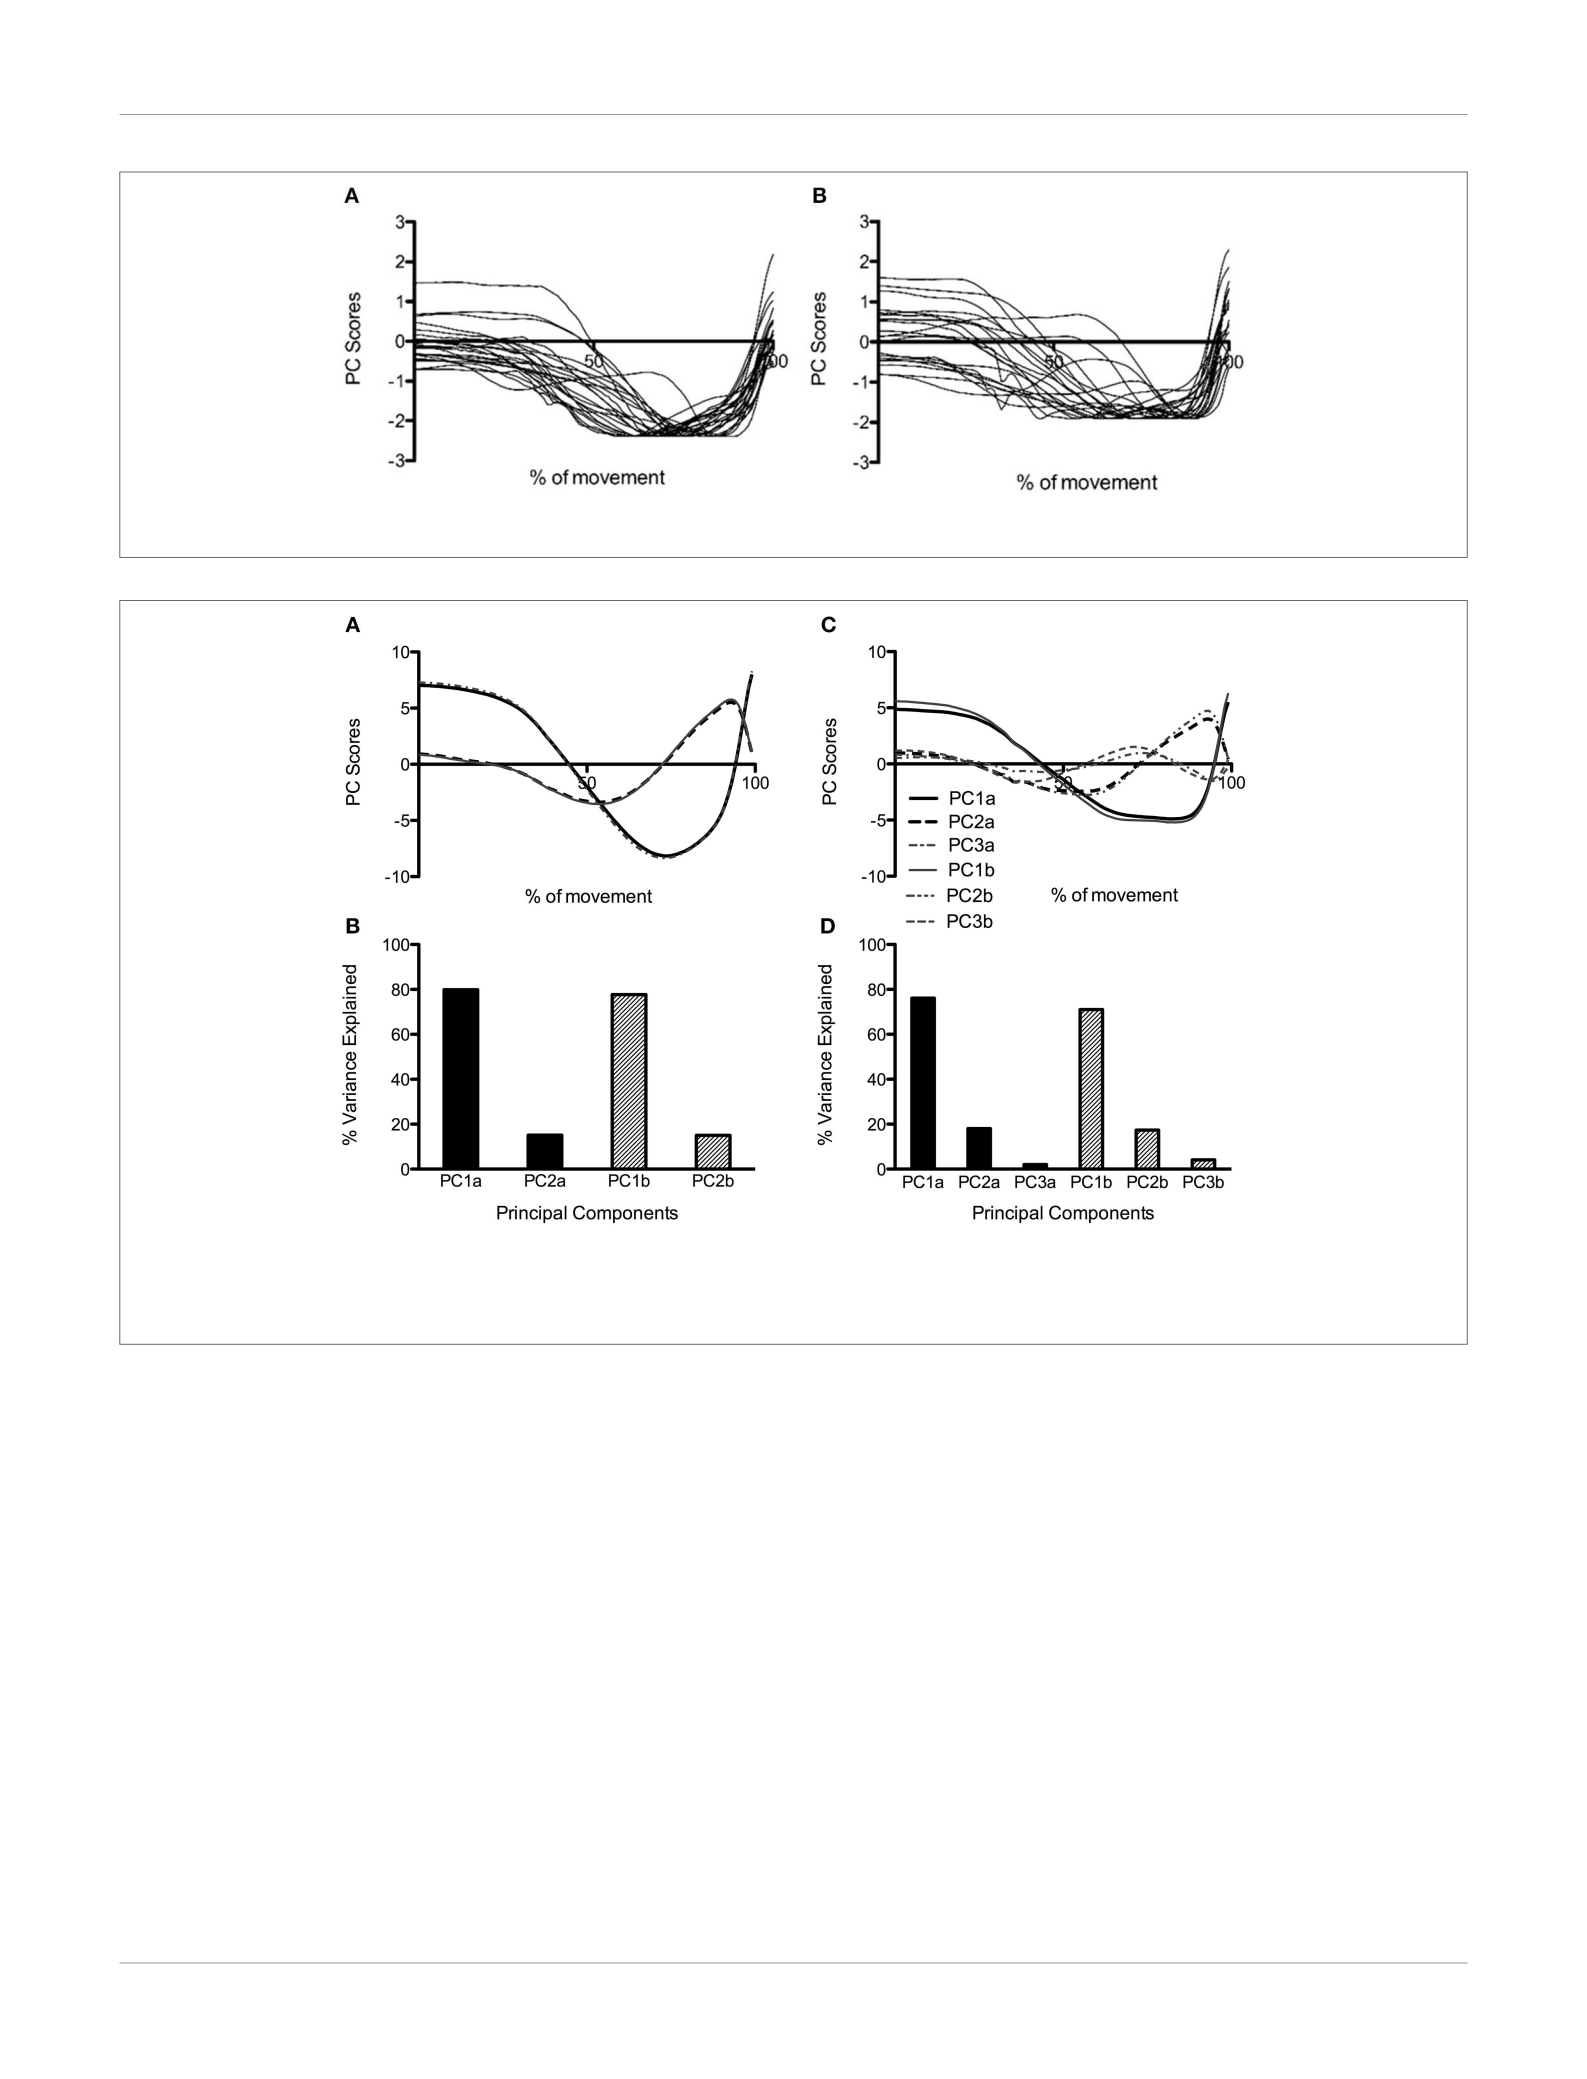
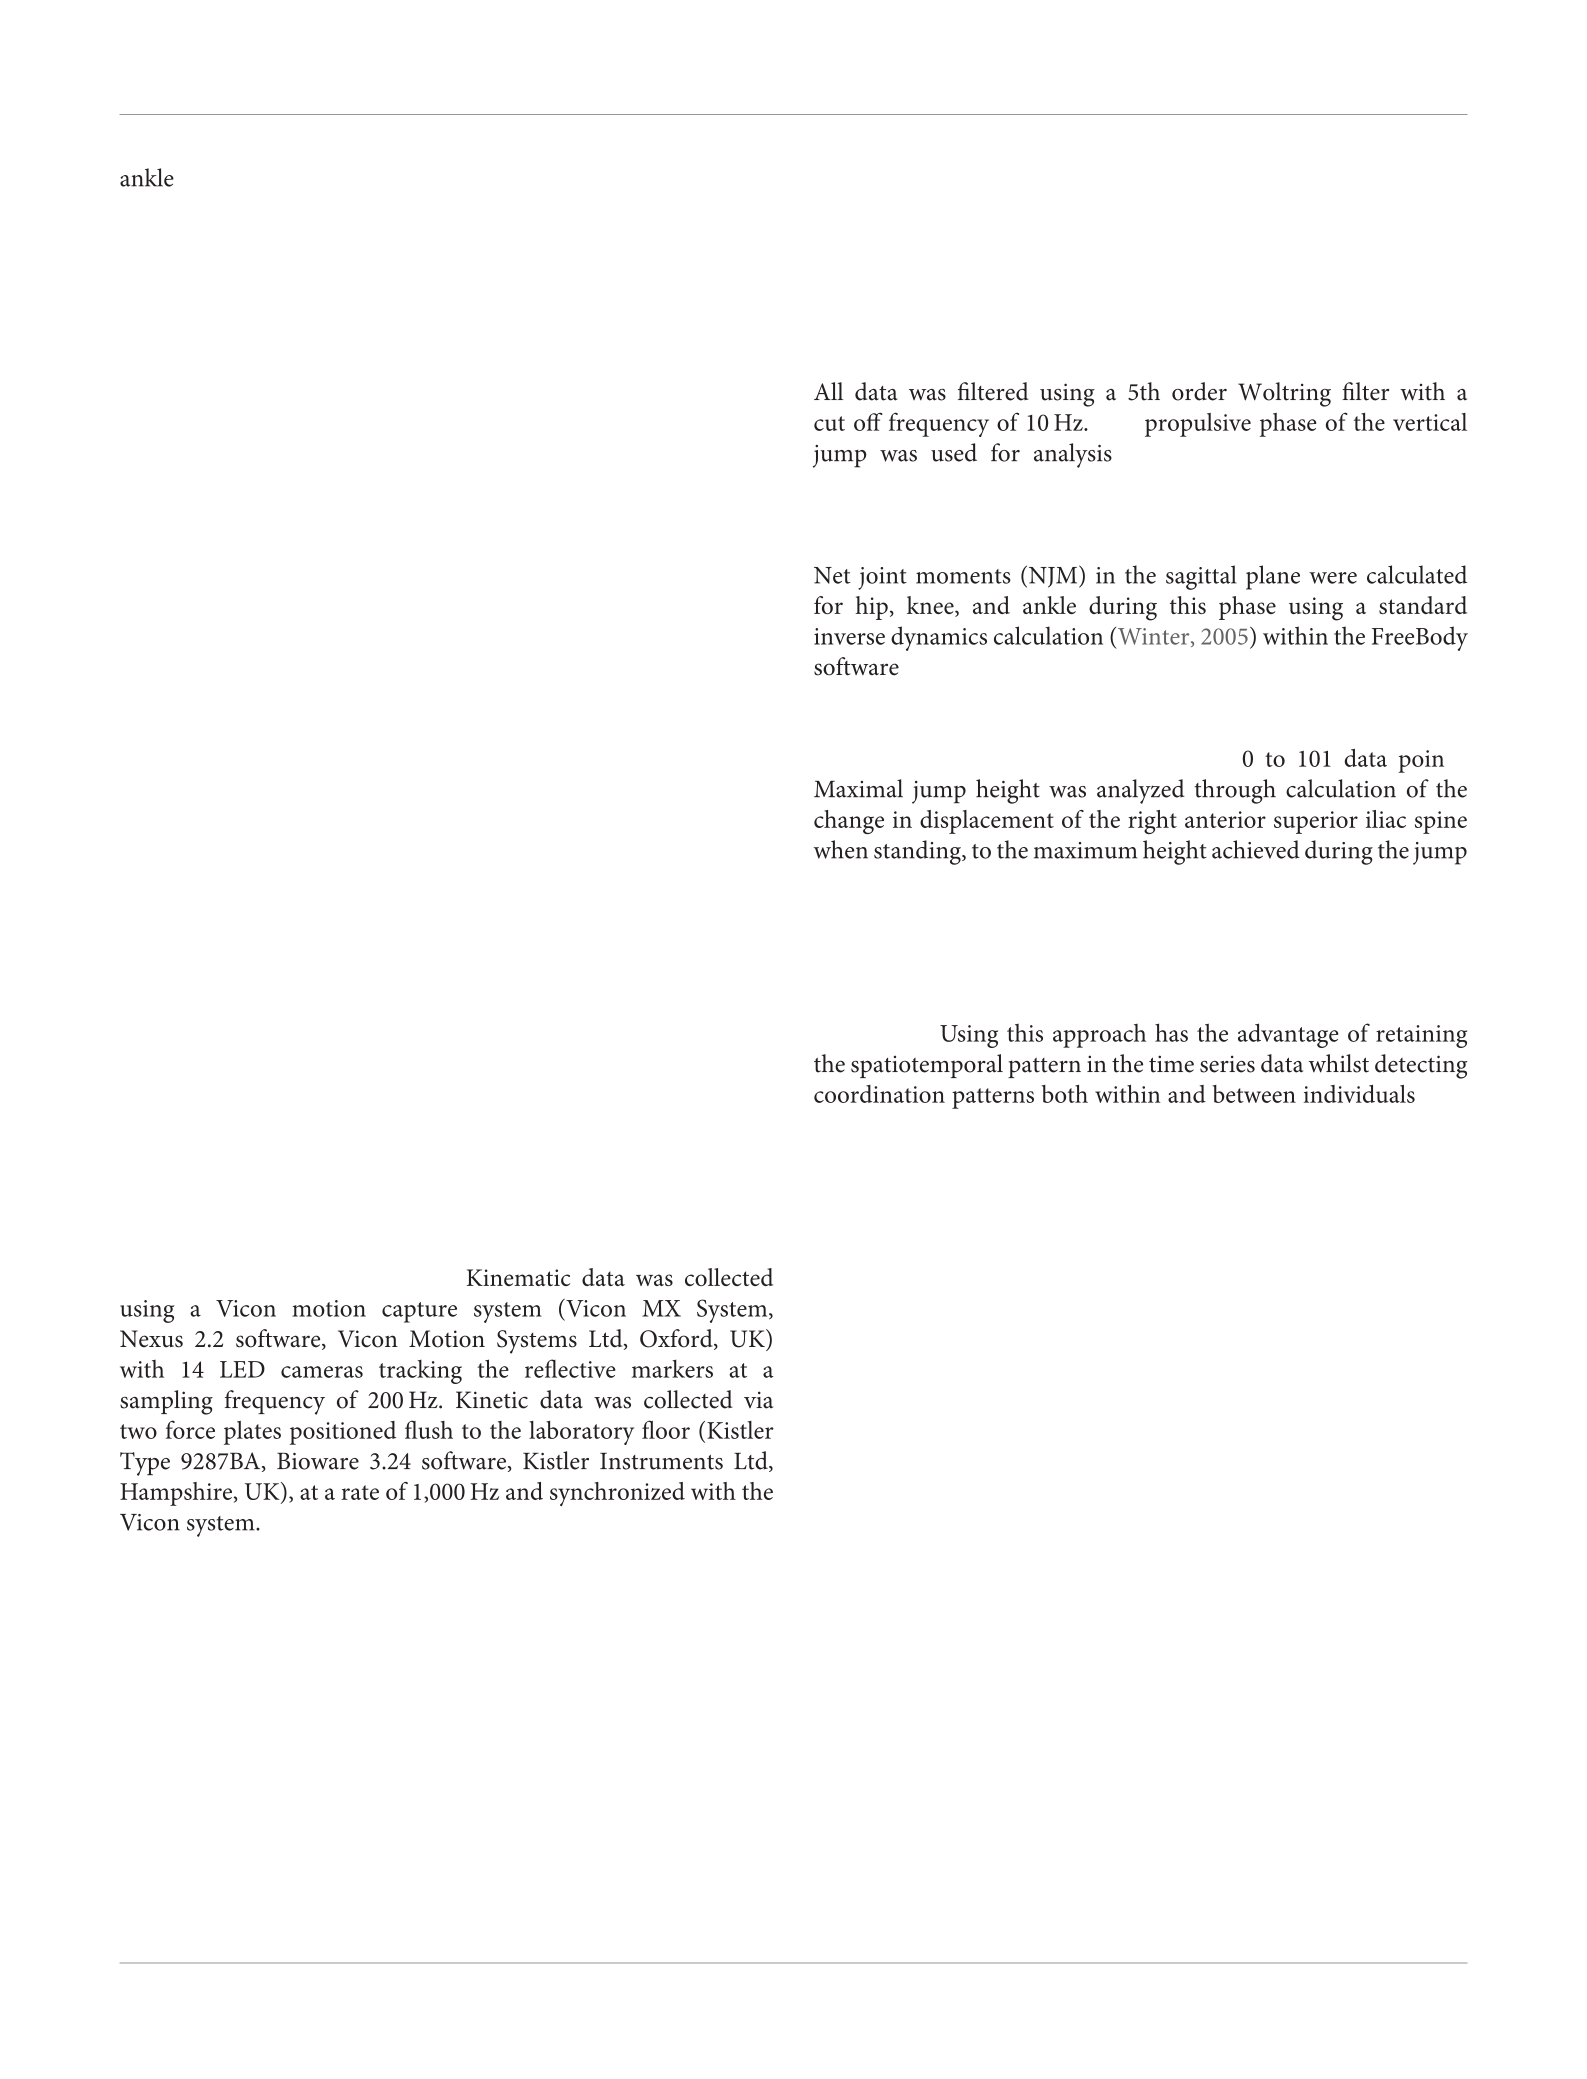
FIGURE 2 | PC1i scores for (A) CMJnas and (B) CMJas from 22 participants completing both conditions. Data is normalized to peak value. i =individual PCA analysis.
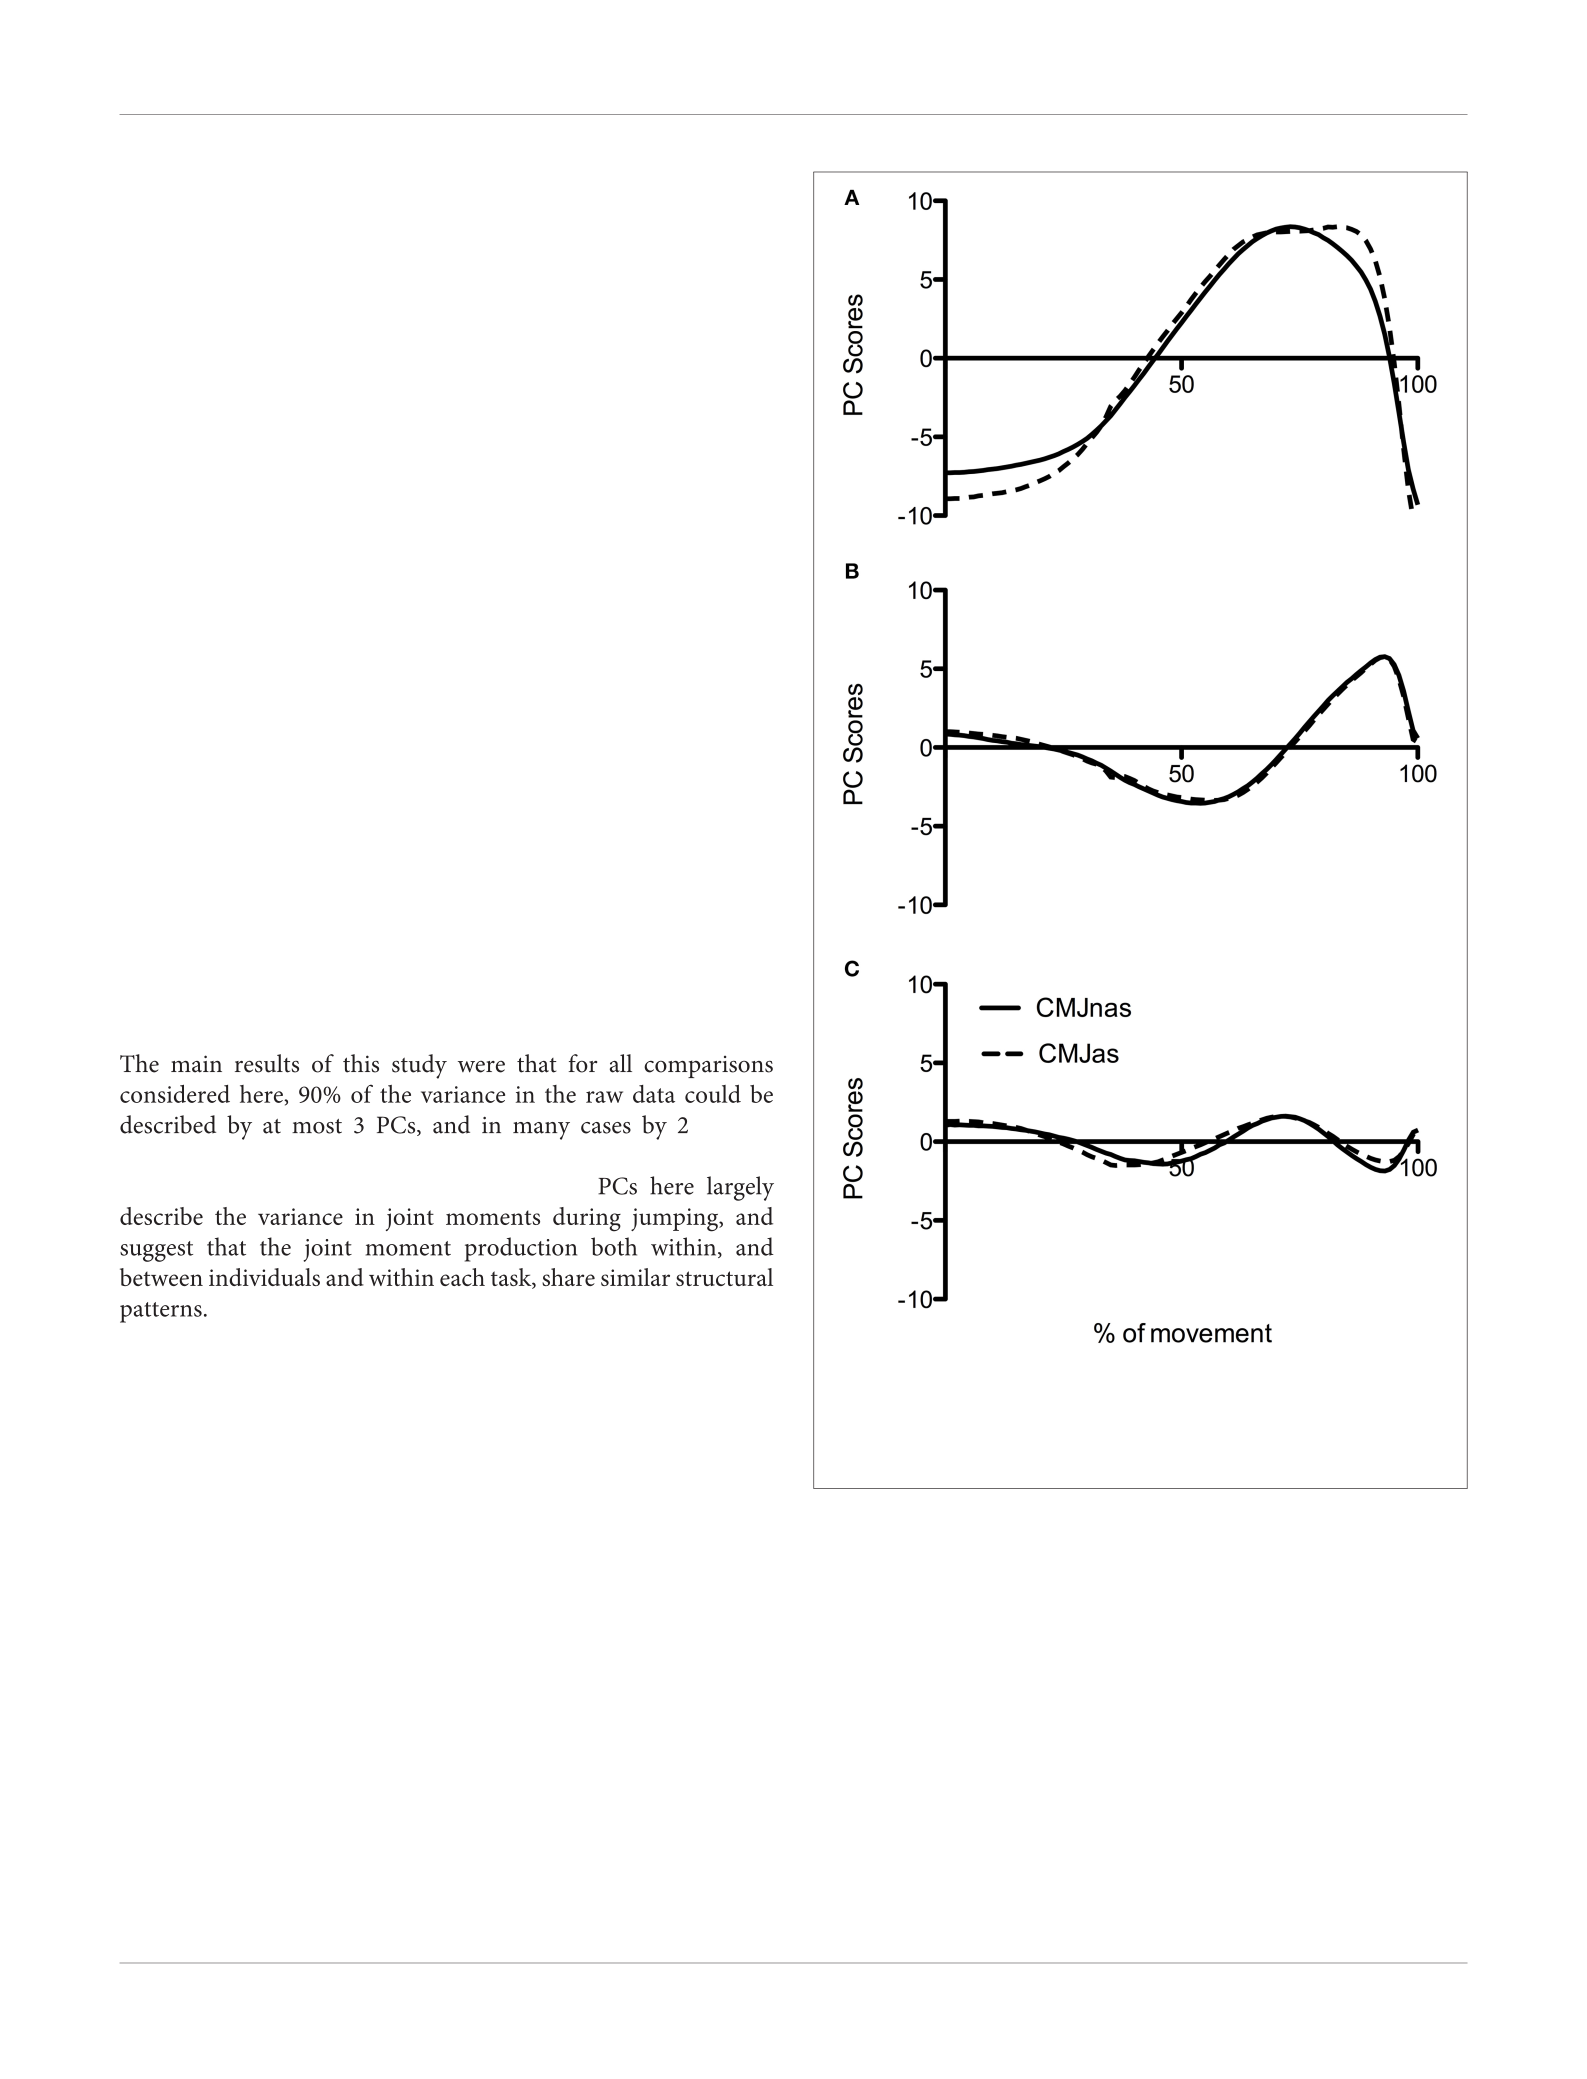
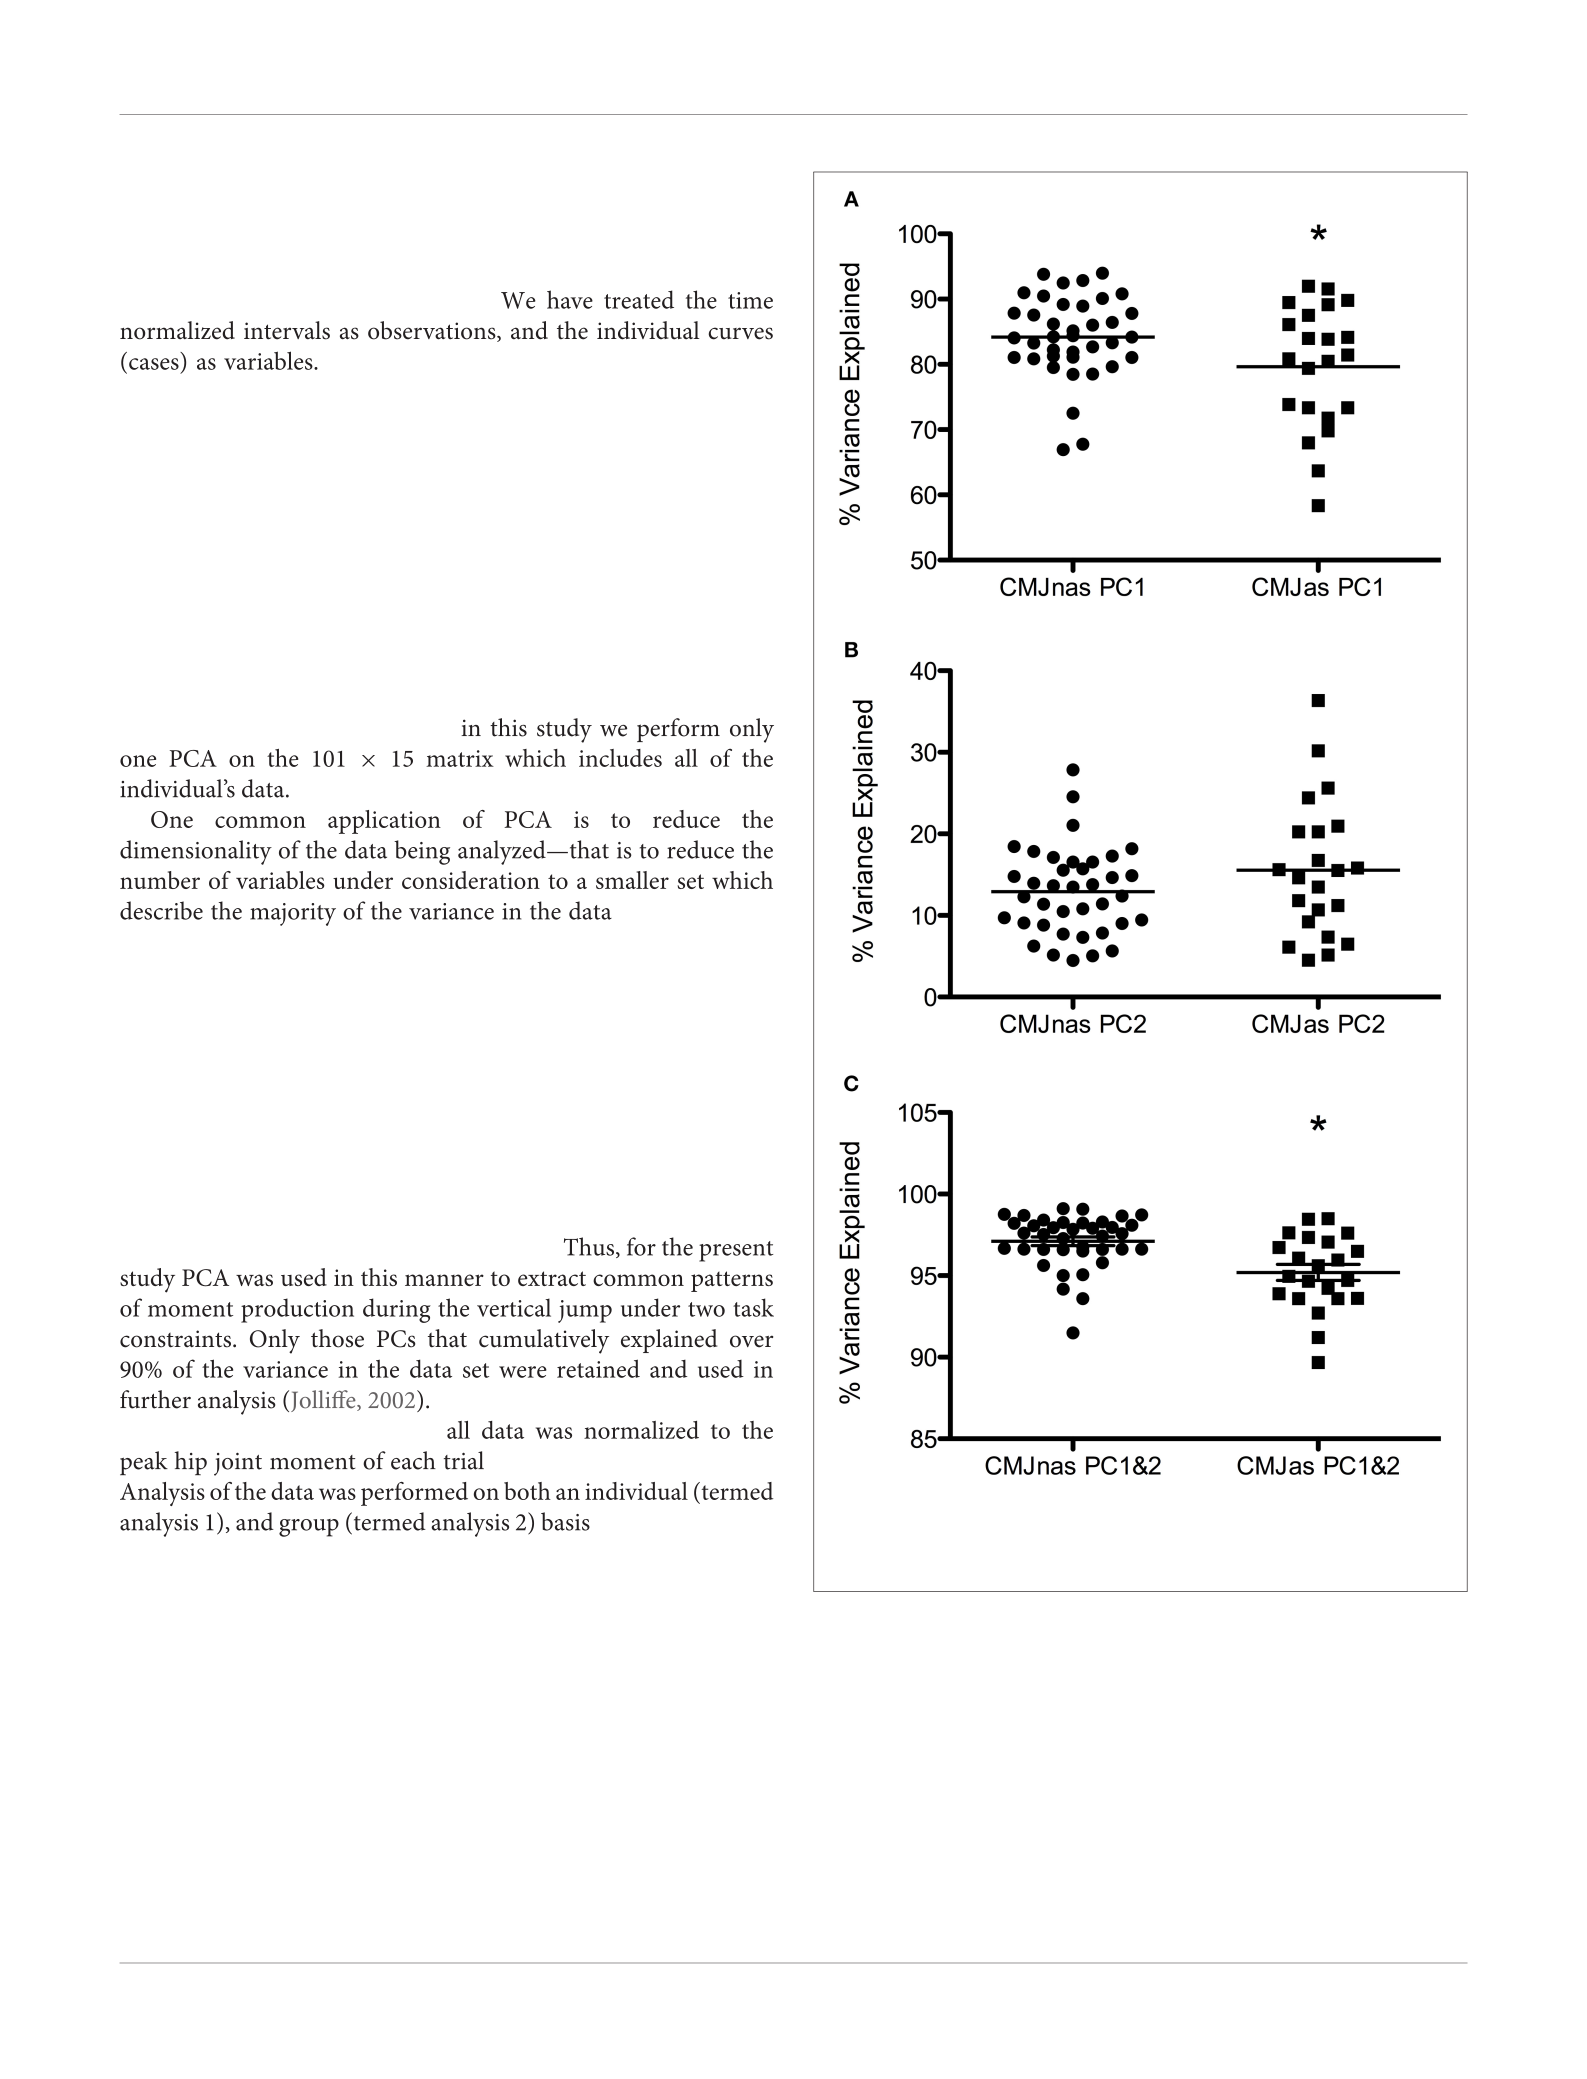
FIGURE 3 | PC waveforms along with percentage of explained variance for CMJnas (A,B) and CMJas (C,D) conditions. Data in (C) has been flipped to a negative
peak to more clearly show comparison between the shape of waveforms in (A,C). PC1, 2, and 3a represent data obtained from PCA using only the first two PCs from
each individual (analysis 4). PC1, 2, and 3b represent data obtained from group PCA for CMJnas, and CMJas (analysis 2).
of a PC, and the PCs are ordered in terms of the amount of
variance they explain. The coefficients matrix thus gives the
transformation of the raw data into the variable space defined
by the PCs. Thus, the matrix obtained by multiplying the raw
data matrix by the coefficients matrix is a matrix describing
the time-series of the values for each PC. These time series are
reported as the PC scores in this study. Similarly, the raw data
can be reconstructed based upon a limited number of PCs by
transforming the selected number of PCs back to the variable
space defined by the raw data. This was performed for CMJnas
data as an example. All PCA calculations were performed in
Matlab (The MathWorks, Inc., MA, version 2017a).
Statistical Analysis
Further statistical analysis was performed to compare the
variance explained by each PC attained from the individual
analysis of both CMJnas and CMJas. Group differences between
PC1, PC2, and the sum of PC1 and PC2 were assessed using an
independent sample t-test. The alpha level was set at p<0.05.
RESULTS
When considered individually, only one or two PCs were
required to describe at least 90% of the variance in the data.
Data from each individual PCA showed PC1i and the sum of
PC1i, and 2i explained a significantly greater amount of the
variance in CMJnas than CMJas (p=0.05, p=0.00, respectively;
Figure 1). The greater variation in PC1i scores for CMJas can be
seen in Figure 2.
When all joint moment data was combined in the same
PCA, three PCs were retained for the CMJas condition, and
two were retained for the CMJnas condition (Figure 3). Figure 3
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 5August 2019 | Volume 7 | Article 193
Cushion et al. PCA of Vertical Jumping
also illustrates waveforms from the group analysis PCA that just
retained the first two PCs for each individual (analysis 4).
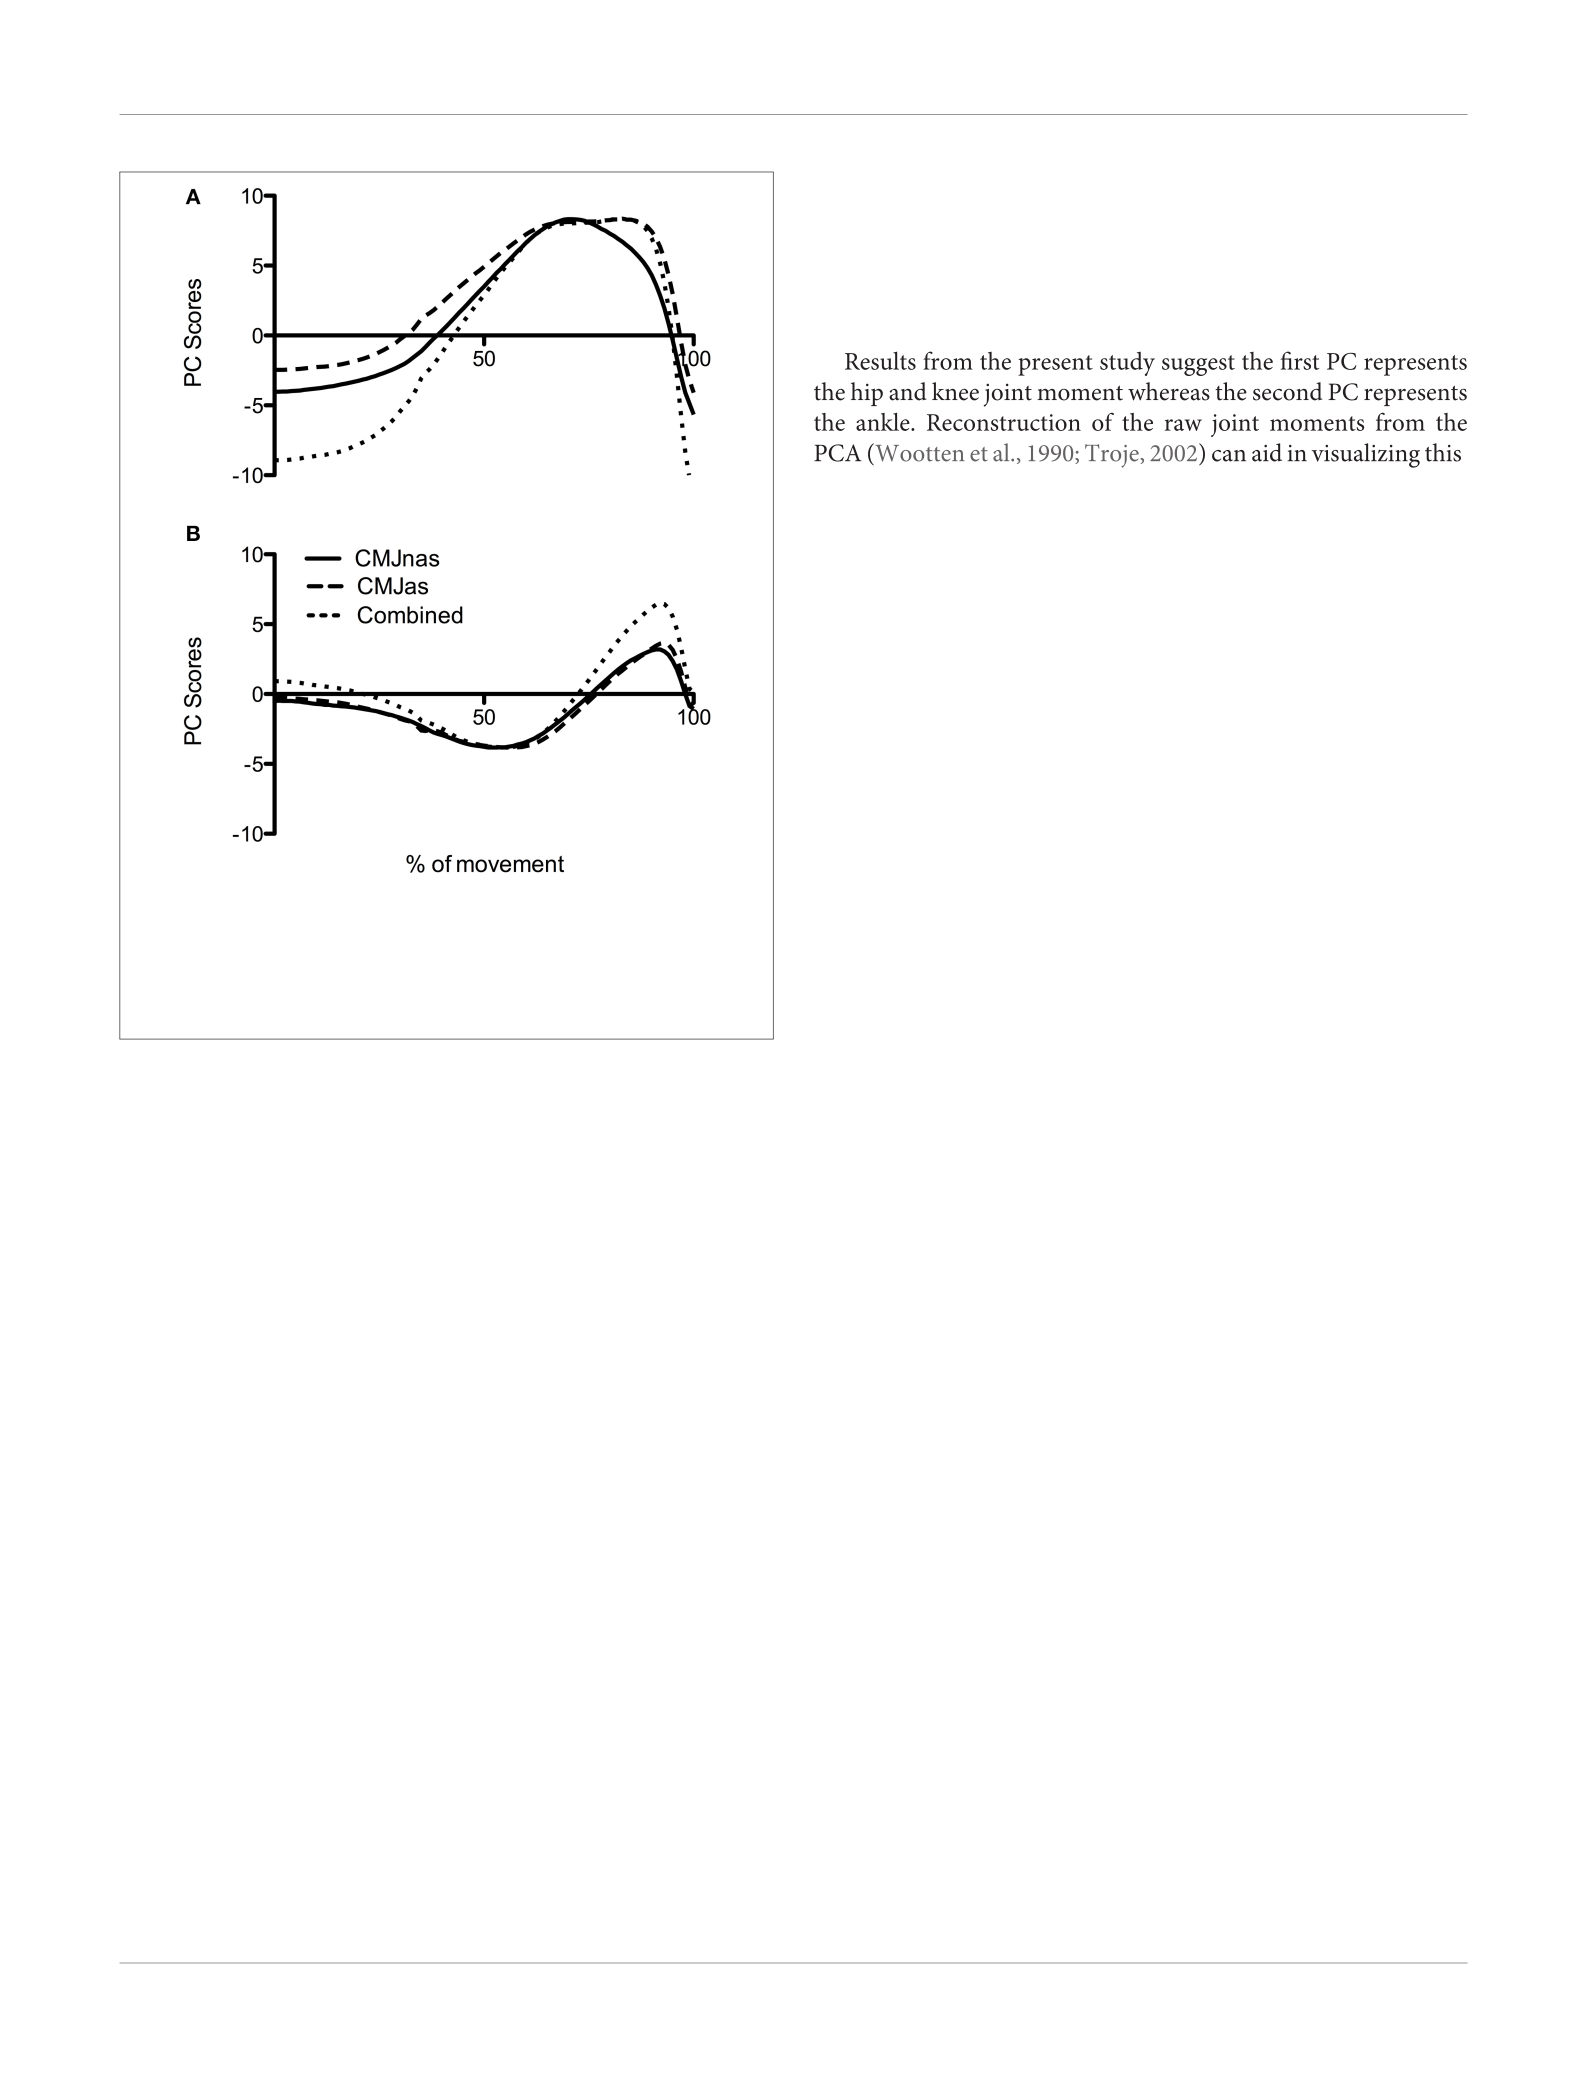
To make a robust comparison between jumps at the group
level, data was reanalyzed with only those participants who
completed both CMJnas and CMJas conditions (Figure 4,
analysis 3). This highlighted the same trend with CMJas requiring
three PCs and CMJnas requiring only two PCs to describe over
90% of the variance. Waveforms for each jump condition were
similar to those observed in Figure 3.
An analysis was also conducted with only those participants
who completed both CMJnas and CMJas conditions with all joint
moment data combined (Figure 5). Only two PCs were required
to explain over 90% of the variance.
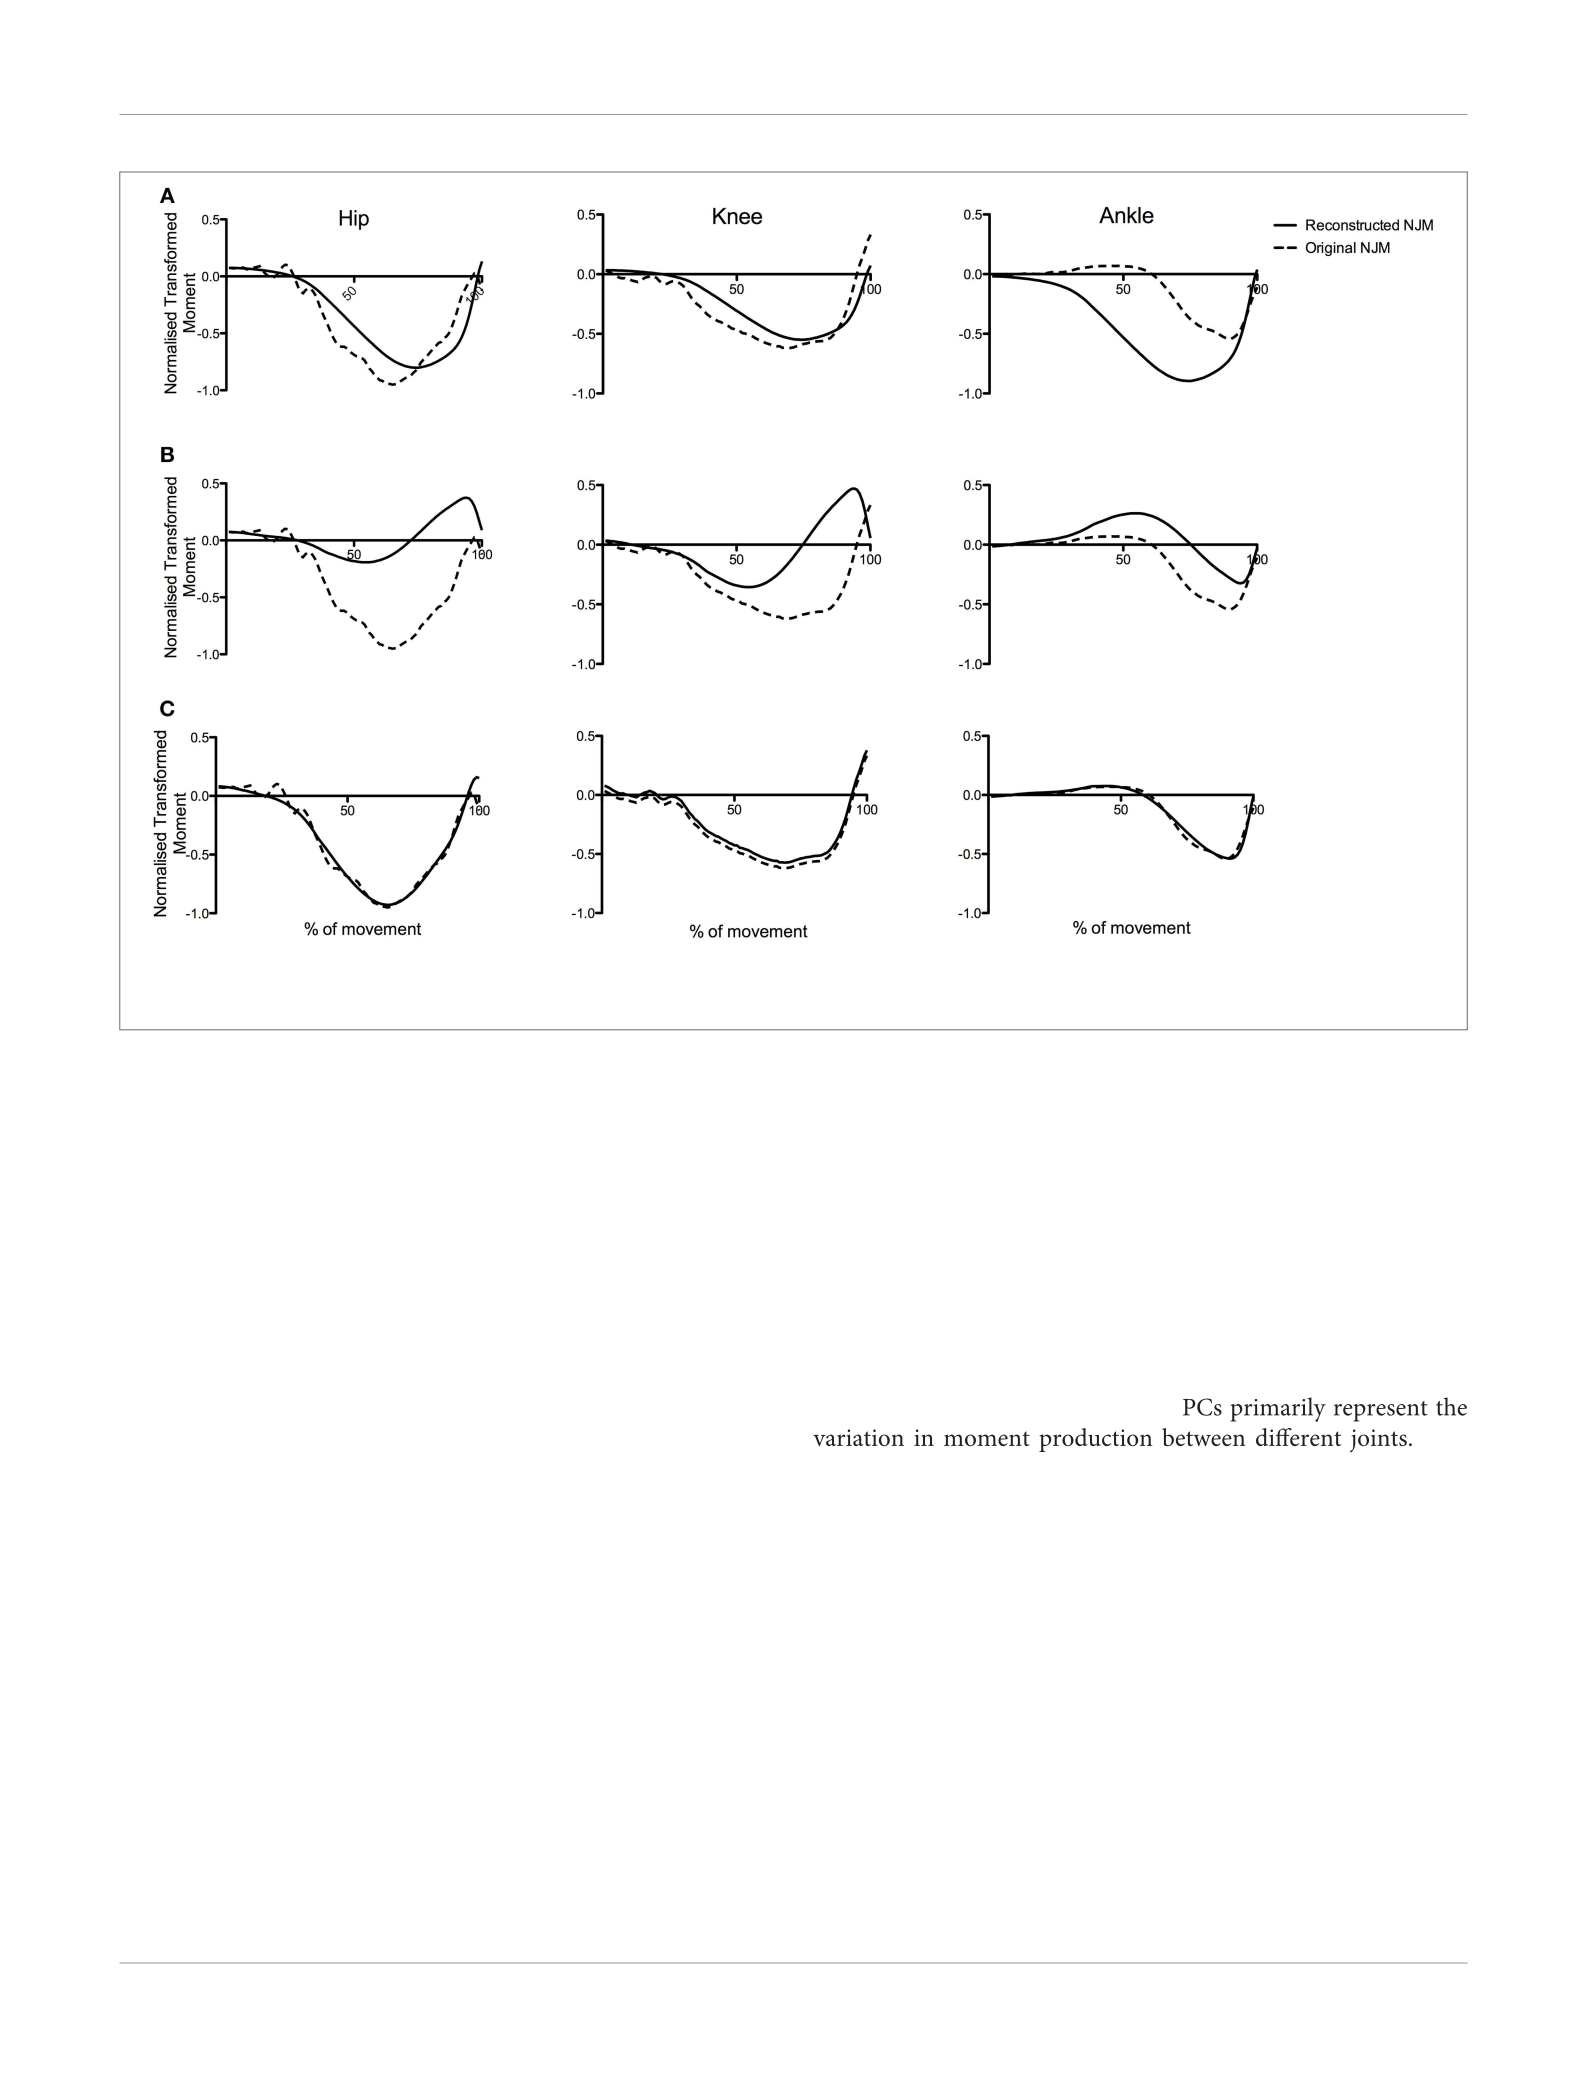
Figure 6 presents an illustrative example of the reconstruction
of a typical jump from PC1g and PC2g—and shows how the
sum of the time series for PC1g and PC2g describe such a high
proportion of the variance in the raw data.
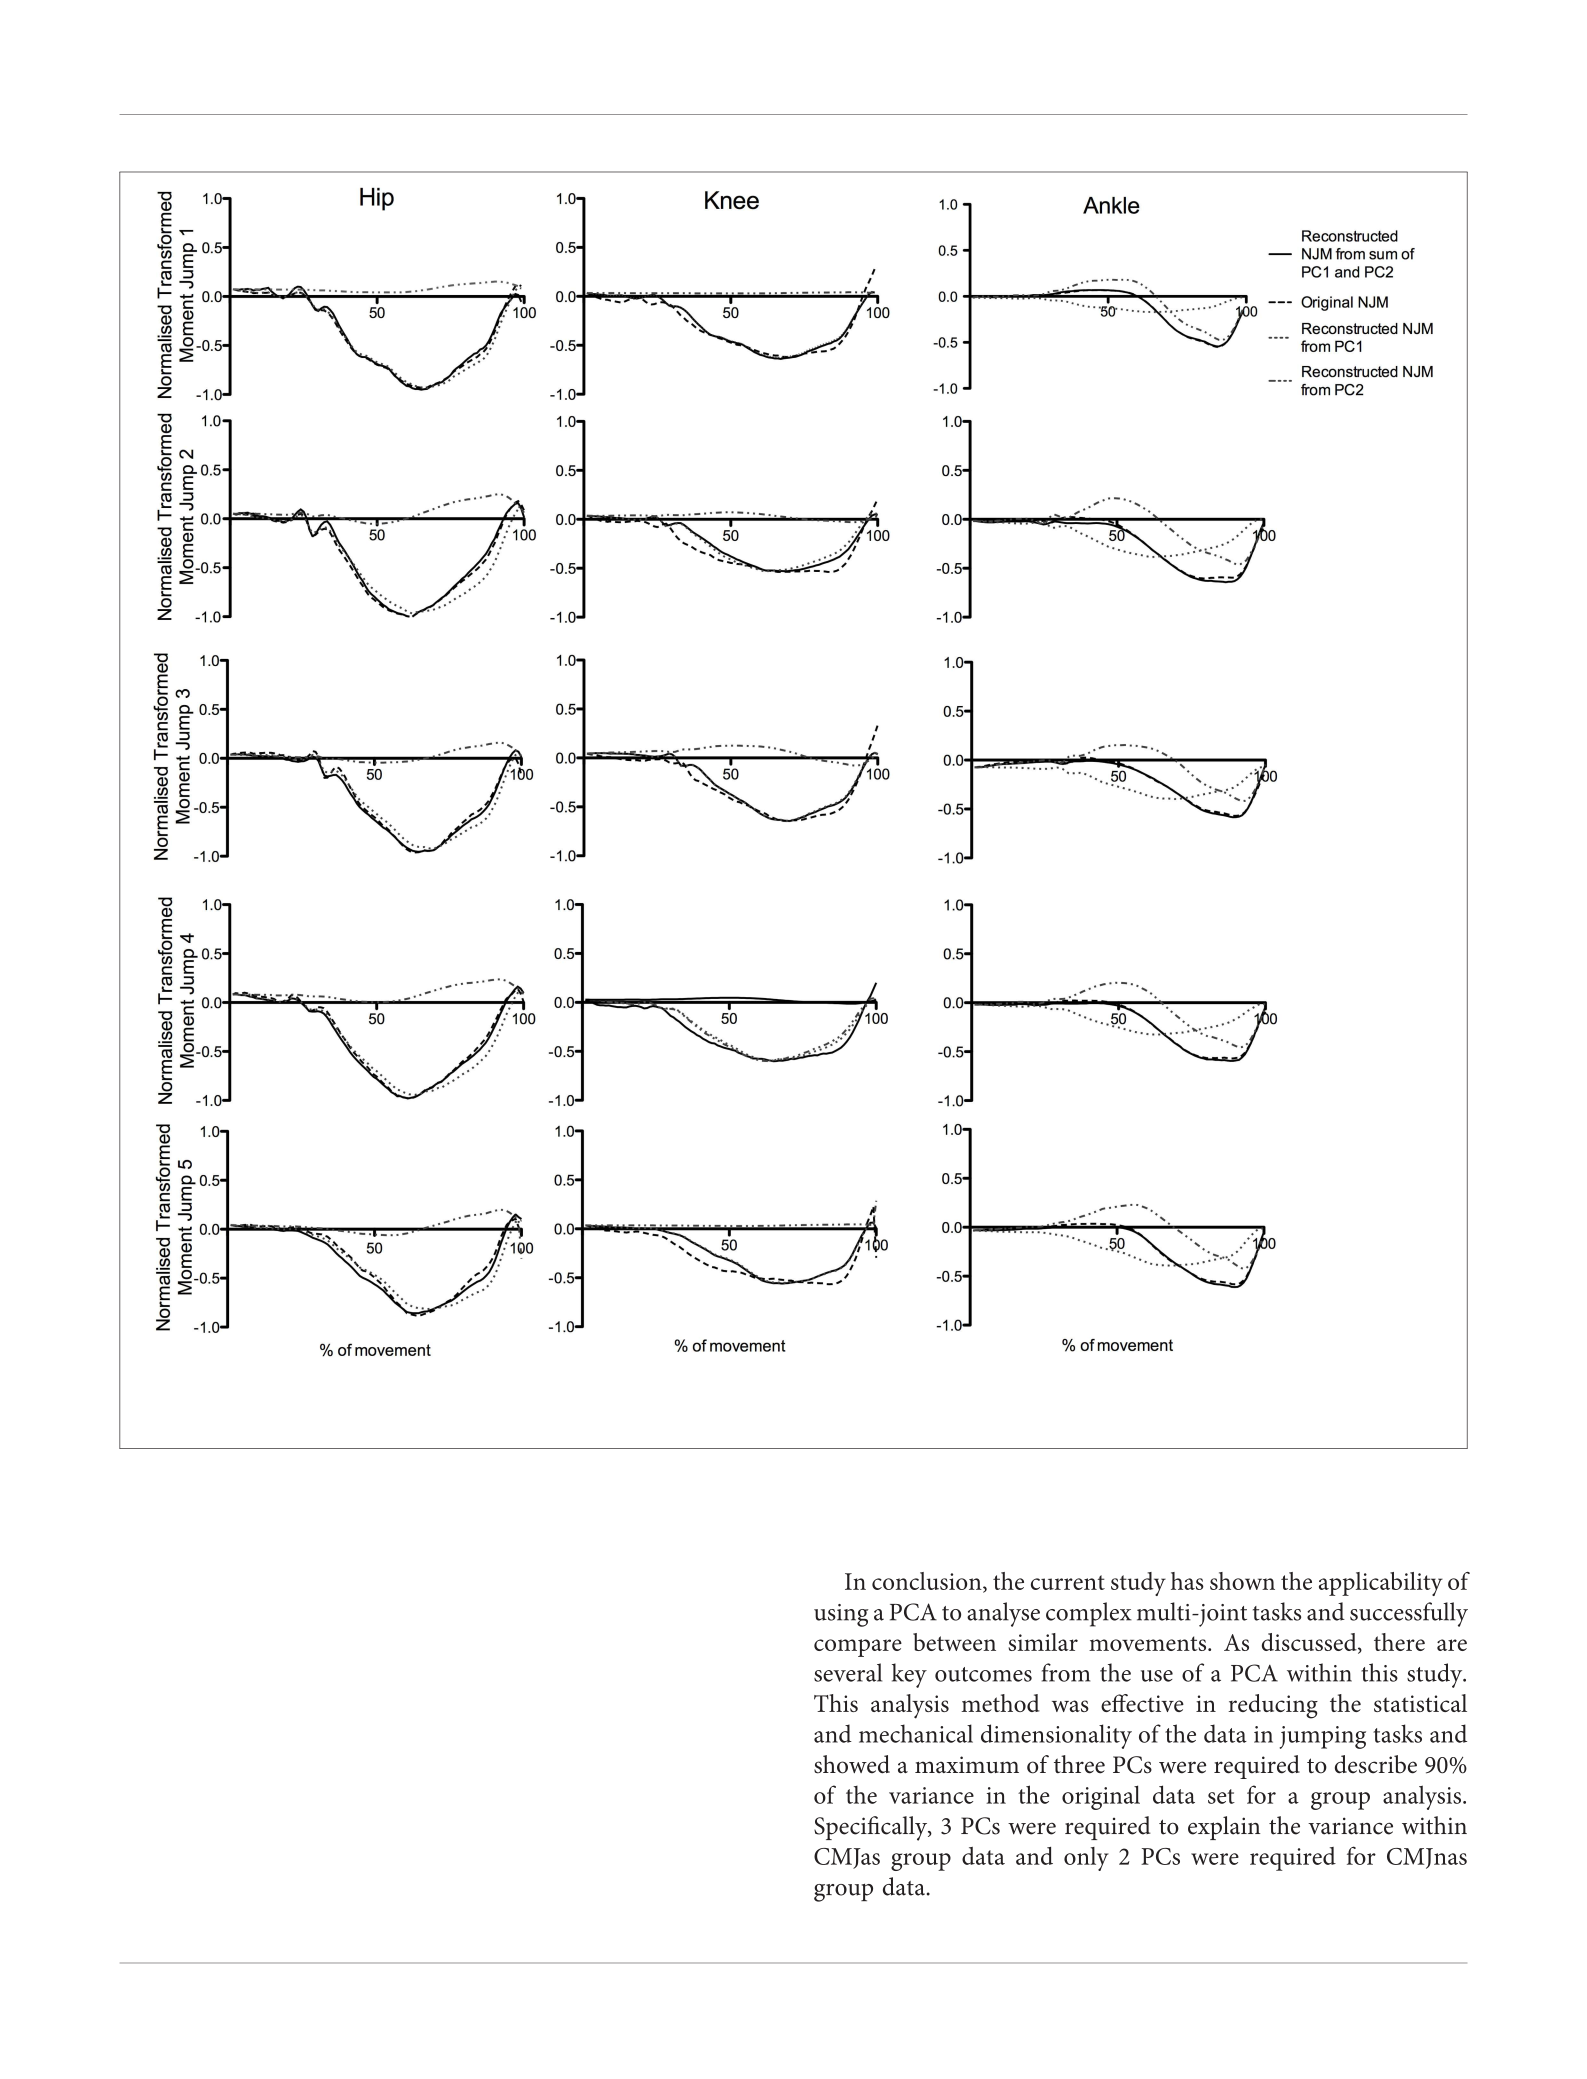
Figure 7 presents an illustrative example of the reconstruction
of a series of five jumps from a representative participant
performing CMJnas. The figure shows the sum of the time series
for PC1i and PC2i describe a high proportion of the variance in
the raw data.
DISCUSSION
The purpose of this study was to use PCA to characterize
movement strategies, through reducing a large data set of
hip, knee, and ankle NJMs measured during vertical jumping.
The main results of this study were that for all comparisons
considered here, 90% of the variance in the raw data could be
described by at most 3 PCs, and in many cases by 2. Whilst
there are multiple sources of variation within the dataset (e.g.,
joint, trial, individual), we suggest that the PCs here largely
describe the variance in joint moments during jumping, and
suggest that the joint moment production both within, and
between individuals and within each task, share similar structural
patterns. Further to this, the dimensionality of sagittal plane
lower limb extension in some forms of vertical jumping can be
reduced to only 2 functional DOF. This is an important result—
it indicates that simply providing the participants with the task
constraint “jump as high as you can” produced a markedly
similar pattern, and that between and within participant variation
amounted to <10%. This is a highly non-trivial result and
provides insight to the nature of motor control within this task—
although it has previously been suggested that during jumping,
people exhibit a characteristic proximal to distal pattern of joint
moment production (Bobbert and van Ingen Schenau, 1988), the
degree of similarity has not been emphasized.
When considering the group and individual analysis for
CMJnas only 2 PCs are required to explain over 90% of
the variance (Figure 3). This would suggest the relationships
between curves are not just unique to specific individuals but are
demonstrated by the whole group. If this was not the case further
PCs would be required to describe the movement. For CMJas an
additional PC was required at the group level in order to capture
90% of the variance in the data (see Figure 3), although it was
FIGURE 4 | Comparison of PC waveforms for CMJnas and CMJas for the 22
participants who completed both jumps: (A) PC1, (B) PC2, and (C) PC3.
CMJas waveforms have been flipped and peaks matched to show differences
in temporal pattern.
not required at the individual level. These results are consistent
with previous research findings which have also looked to
determine how the high dimensionality of human movement can
be reduced to low dimensional states (see Soechting and Flanders,
1997; Borzelli et al., 1999; Balasubramaniam and Turvey, 2004;
Witte et al., 2009; Nordin and Dufek, 2016a; Majed et al., 2017),
For example, (Santello et al., 1998) have shown that in a hand
grasping task only two PCs were required to describe over 80% of
the variance in the data, demonstrating few synergies govern the
production of hand motion in the specific grasping task. Equally,
in a sit to stand task only two PCs were required to describe
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 6August 2019 | Volume 7 | Article 193
Cushion et al. PCA of Vertical Jumping
FIGURE 5 | Comparison of PC waveforms for CMJnas and CMJas for the 22
participants who completed both jumps along with PC waveform of combined
CMJnas and CMJas analysis (analysis 3): (A) PC1, (B) PC2. CMJas
waveforms have been flipped and data peaks matched to show differences in
temporal pattern.
the task from six components of ground reaction force data (see
Borzelli et al., 1999).
It is interesting to note that at only the group level an
additional PC was required to describe over 90% of the variance
within the dataset for CMJas. The need for the third PC is
indicative of the greater variability in the CMJas data. This
greater variability is seen both within individuals (see Figure 1)
and between individuals (see Figure 2), where a significant
difference in explained variance for PC1 was observed between
CMJnas and CMJas. In contrast, in analysis 4 (which essentially
eliminates the effect of within individual variation on the group
scores) only 2 PCs are required to explain 90% of the variance.
This improvement in predictive value is gained in the variance
explained by PC1g. It is interesting to consider the shape of
the PC3g score and think about the linear sum of the PC1g
score with PC3g score. In particular, the effect of adding PC3g
to PC1g is to make the curve less flat and to make it more
peaked toward the end of the jump. This type of variation is also
seen between individuals (Figure 2). It is also worth noting that
the requirement for a third PC for the group analysis provides
further support for the fact that the reduction to 2 PCs seen
for CMJnas is not trivial. The increase in variability within
the CMJas data could be related to unfamiliarity with the task
or complexity of the task for the participants involved. It has
previously been demonstrated an increase in complexity of a
task results in an increase in dimensionality and a reduction in
explained variance within the first principal component (Zago
et al., 2017). Whilst participants within this study were familiar
with jumping, the requirement to use an arm swing may have
added complexity to the task such that they were required
to explore movement options to a greater extent than in the
constrained CMJnas condition.
Results from the present study suggest the first PC represents
the hip and knee joint moment whereas the second PC represents
the ankle. Reconstruction of the raw joint moments from the
PCA (Wootten et al., 1990; Troje, 2002) can aid in visualizing this.
The reconstruction of the moment curves for a representative
individual (see Figure 6), shows the score for PC2i featuring
heavily in the linear sum of the reconstructed curve for the
ankle moments. Similarly, the first PC curve shares a similar
pattern to either the hip or knee joint moment curve—this varied
depending on the individual (for the individual in Figure 6 it
was hip-like). The relationship between the two PCs can also
be seen in Figure 7. Consider, for instance, the ankle moments
and compare jump1 to jump4. Here jump4 shows a flatter peak
compared to jump1 and a much wider curve. Consideration of
the 2 PC scores shows how these 2 quite different ankle moment
curves can still be constructed. In particular, the scores for PC1i,
and PC2i are out of phase, however the difference in timing
between them is such that they can still be summed to produce
all the different ankle curve combinations. To put this another
way, given the differences in the shape of the ankle curves we
know that at least 2 PCs would be needed to reconstruct them.
However, the 2 PCs that we obtain not only allow all of the
ankle moment curves to be created, but also all the hip and knee
moment curves. This synergy implies a relationship between the
different joint moment curves that persists across jumps.
This concept of synergy is not unique to this study and
demonstrates an approach of the system to optimize control of
motor tasks (see Santello et al., 1998; Jaric and Latash, 1999;
St-Onge et al., 2004; Todorov and Ghahramani, 2004; Latash
et al., 2007; Latash, 2010; Kipp et al., 2012; Nordin and Dufek,
2017). This organization of movement to synergies may occur
due to mechanical constraints (defined as limits in the options of
motion that can be achieved due to the mechanical configuration
of the human body) on the system that determine the movement
pattern—so called mechanical intelligence (Blickhan et al., 2006).
Within this study it is suggested that the proximal to distal
pattern of moment production (in the sagittal plane) during
vertical jumping might be governed by only 2 functional
DOF and this may be related to mechanical constraints. For
instance, Cleather (2018) has recently shown how the geometry
of the patellofemoral joint alone can explain over 90% of the
variance in the relative timing of femoral and tibial segment
moments (Cleather, 2018). To put that observation in terms
of the findings reported here, the patella could provide a
mechanical constraint that reduces 2 functional DOF to 1—
the hip and knee moments are largely dependent on one
another. This would then represent a potential explanation for
the remarkably consistent timing of moment production here. It
seems more credible that such consistency would be produced
by a mechanical feature of human anatomy that is shared by
all (a shared organismic mechanical constraint), than it being
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 7August 2019 | Volume 7 | Article 193
Cushion et al. PCA of Vertical Jumping
FIGURE 6 | Original NJMs (raw data) for a typical CMJnas compared with reconstructed data using only the first two principal components. The reconstructed curve
in (C) is the linear sum of the curves in (A,B).
the result of everyone learning a pattern of motor coordination
during their development that is so markedly consistent. A
similar conclusion of mechanical constraints reducing the
dimensionality of movement patterns has been proposed in a
similar, albeit much slower task of sit to stand (Borzelli et al.,
1999) as well as in drop landings (Nordin and Dufek, 2017).
An additional comparison between CMJnas and CMJas was
made between only those individuals who had completed both
forms of the jump (Figures 4,5, analysis 3). This comparison
demonstrates that the PC2g scores are effectively the same. This
can be interpreted as suggesting that the ankle is being used in
the same way, and that the potential effect of the ankle on the
relative timing of hip and knee NJM is also the same. However,
there is a notable difference in the PC1g scores. Specifically,
Figure 4A shows PC1g curves between each jump. This shows
a PC1g curve for CMJas to exhibit a flatter peak along with a
greater area under the curve compared to the CMJnas condition.
This is likely to be reflective of the use of the arm swing to slow
joint extension and thus provide greater time for the musculature
to develop force (Feltner et al., 2004; Domire and Challis, 2010).
Previous literature (e.g., Lees et al., 2004; Hara et al., 2006)
has suggested that the use of the lower limb in CMJnas and
CMJas is distinct. The results reported here suggest that although
this is true, the motor control strategy only differs in terms of
the first PC, and that there is still a striking similarity between
the movements.
Whilst interesting and novel findings have been identified
within this study, limitations of this work should be highlighted.
Although statistically rigorous procedures have been employed,
the analysis of the results is in some parts interpretative. This is a
limitation of trying to describe the mechanics of movement from
statistical techniques—although it should be noted that we are
not alone in using this technique to tease out different sources
of variation (e.g., Daffertshofer et al., 2004). In particular, there
are multiple sources of variation—joints (hip, knee or ankle),
participant, trial, and type of jump (with or without arms). Our
contention in this paper is that the PCs primarily represent the
variation in moment production between different joints. This
can be inferred based upon the following reasoning. Firstly, the
PCA analysis was first performed considering each individual
separately—thus eliminating inter-individual variability—this
analysis produced similar PC1i and PC2i for each participant
suggesting that the PC1g and PC2g are not produced by inter-
individual variability. Secondly, the group PCA analysis was
performed on both the whole data set, and on a reduced data
set comprising the resulting PCs from the individual analysis.
Inter-trial variation for each individual would be to a large part
mitigated in the latter data set, yet there was little difference in
the results of these two analyses (Figure 3). This suggests that
inter-trial variability is not a major factor in the group PCs.
Thirdly, the variation based upon type of jump was quantified
by the comparison of CMJas and CMJnas in Figure 4, and the
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 8August 2019 | Volume 7 | Article 193
Cushion et al. PCA of Vertical Jumping
FIGURE 7 | Original NJMs (raw data) for a typical CMJnas compared with reconstructed data using only the first two principal components, for a representative
participant across five jump trials.
same PCs were found for both jump types. Having eliminated 3
of the 4 sources of variation, we suggest that the PCs from the
group analysis describe variation in joint moment production.
Of course, this contention has not been “proven” statistically,
but, we argue, is the only reasonable explanation. Furthermore,
Figures 6,7demonstrate the reconstruction of joint moments
from the PCA. This shows the similarity of the reconstructed
curves to the original raw joint moment curves. If variance was
predominantly from individual differences in jumping style, the
ability to so closely reconstruct the moment curves would likely
not occur. In addition, whilst the focus of this research was
on the analysis of the lower limb during jumping, based on
their large contribution to the movement, future research would
benefit from conducting a whole-body analysis to determine the
dimensionality of the system.
In conclusion, the current study has shown the applicability of
using a PCA to analyse complex multi-joint tasks and successfully
compare between similar movements. As discussed, there are
several key outcomes from the use of a PCA within this study.
This analysis method was effective in reducing the statistical
and mechanical dimensionality of the data in jumping tasks and
showed a maximum of three PCs were required to describe 90%
of the variance in the original data set for a group analysis.
Specifically, 3 PCs were required to explain the variance within
CMJas group data and only 2 PCs were required for CMJnas
group data. The first PC has a greater loading for hip and knee
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 9August 2019 | Volume 7 | Article 193
Cushion et al. PCA of Vertical Jumping
joint moments, whereas the second PC has a greater loading
for the ankle joint moment. The results suggest the proximal to
distal extension pattern in the sagittal plane typical of vertical
jumping tasks is governed by only 2 functional DOF rather than
the previously reported 3 mechanical DOF. This study adds to the
motor control literature suggesting that despite the redundancy
within the system coordinated movements are produced based
on task and mechanical constraints. Importantly, the results
suggest vertical jumping is controlled by 2 functional DOF at
both an individual and group level. We suggest the reduction
in dimensionality of the movement may be mechanically driven
by human anatomy.
ETHICS STATEMENT
All subjects gave written informed consent in accordance with the
Declaration of Helsinki. The protocol was approved by the ethics
sub-committee of St Mary’s University.
AUTHOR CONTRIBUTIONS
EC, JN, and DC were involved in the design of the
study. EC carried out all data collection. All authors
were involved in the interpretation and final write
up of the study.
REFERENCES
Balasubramaniam, R., and Turvey, M. T. (2004). Coordination modes in
the multisegmental dynamics of hula hooping. Biol. Cybern. 90, 176–190.
doi: 10.1007/s00422-003-0460-4
Bates, B. T. (1996). Single-subject methodology: an alternative approach. Med. Sci.
Sports. Exerc. 28, 631–638. doi: 10.1249/00005768-199605000-00016
Bernstein, N. A. (1967). The Co-ordination and Regulation of Movements. Oxford:
Pergamon Press.
Blickhan, R., Seyfarth, A., Geyer, H., Grimmer, S., Wagner, H., and Gunther,
M. (2006). Intelligence by mechanics. Phil. Trans. R. Sco. A. 365, 199–220.
doi: 10.1098/rsta.2006.1911
Bobbert, M. F., and van Ingen Schenau, G. J. (1988). Coordination in vertical
jumping. J. Biomech. 21, 249–262. doi: 10.1016/0021-9290(88)90175-3
Borzelli, G., Cappizzon, A., and Papa, E. (1999). Inter and intra
individual variability of ground reaction forces during sit to stand
with principal component analysis. Med. Eng. Phys. 21, 235–240.
doi: 10.1016/S1350-4533(99)00050-8
Button, C., MacLeod, M., Sanders, R., and Coleman, S. (2003). Examining
movement variability in the basketball free-throw action at different skill levels.
Res. Q. Exerc. Sport. 74, 257–269. doi: 10.1080/02701367.2003.10609090
Chiu, L. Z. F., and Salen, G. J. (2010). Pelvic kinematic method for determining
vertical jump height. J. App. Biomech. 26, 508–511. doi: 10.1123/jab.26.4.508
Chow, J. Y., Davids, K., Button, C., and Rein, R. (2008). Dynamics of movement
patterning in learning a discrete multiarticular action. Motor Control 12,
219–240. doi: 10.1123/mcj.12.3.219
Cleather, D. J. (2018). The patella: a mechanical determinant of
coordination during vertical jumping. J. Theor. Biol. 446, 205–211.
doi: 10.1016/j.jtbi.2018.03.013
Cleather, D. J., and Bull, A. M. J. (2015). The development of a segment based
musculoskeletal model of the lower limb: introducing freebody. R. Soc. Open
Sci. 2, 140–449. doi: 10.1098/rsos.140449
Cleather, D. J., Goodwin, J. E., and Bull, A. M. J. (2013). Inter-segmental moment
analysis characterises the partial correspondence of jumping and jerking. J.
Strength. Cond. Res. 27, 89–100. doi: 10.1519/JSC.0b013e31825037ee
Daffertshofer, A., Lamoth, C. J., Meijer, O. G., and Beek, P. J. (2004). PCA in
studying coordination and variability: a tutorial. Clin. Biomech. 19, 415–428.
doi: 10.1016/j.clinbiomech.2004.01.005
Deluzio, K. J., and Astephen, J. L. (2007). Biomechanical features of gait waveform
data associated with knee osteoarthritis an application of principal component
analysis. Gait Posture. 25, 86–93. doi: 10.1016/j.gaitpost.2006.01.007
Deluzio, K. J., Wyss, U. P., Zee, B., Costigan, P. A., and Serbie, C.
(1997). Principal component models of knee kinematics and kinetics:
normal vs. pathological gait patterns. Hum. Movement. Sci. 16, 201–217.
doi: 10.1016/S0167-9457(96)00051-6
Domire, Z. J., and Challis, J. H. (2010). An induced energy analysis to determine
the mechanism for performance enhancement as a result of arm swing during
jumping. Sports. Biomech. 9, 38–46. doi: 10.1080/14763141003692639
Dona, G., Preatoni, E., Cobelli, C., Rodano, R., and Harrison, A. J.
(2009). Application of functional principal component analysis in
race walking: an emerging methodology. Sports. Biomech. 8, 284–301.
doi: 10.1080/14763140903414425
Dufek, J. S., Bates, B. T., Stergiou, N., and James, C. R. (1995). Interactive effects
between group and single-subject response patterns. Hum. Movement Sci, 14,
301–323. doi: 10.1016/0167-9457(95)00013-I
Federolf, P. A., Boyer, K. A., and Andriacchi, T. P. (2013). Application of principal
component analysis in clinical gait research: identification of systematic
differences between healthy and medial knee-osteoarthritic gait. J. Biomech. 46,
2173–2178. doi: 10.1016/j.jbiomech.2013.06.032
Feltner, M. E., Bishop, E. J., and Perez, C. M. (2004). Segmental and kinetic
contributions in vertical jumps performed with and without an arm swing. Res.
Q. Exerc. Sport. 75, 216–230. doi: 10.1080/02701367.2004.10609155
Forner-Cordero, A., Levin, O., Li, Y., and Swinnen, S. P. (2005). Principcal
component analysis of complex multi-joint coordinative movements. Biol.
Cybern. 93, 63–78. doi: 10.1007/s00422-005-0582-y
Hara, M., Shibayama, A., Takeshita, D., and Fukashiro, S. (2006). The effects of
arm swing on lower extremities in vertical jumping. J. Biomech. 39, 2503–2511.
doi: 10.1016/j.jbiomech.2005.07.030
Hristovski, R., Davids, K., Araujo, D., and Button, C. (2006). How boxers decide to
punch a target: emergent behaviour in nonlinear dynamical movement systems.
J. Sports. Sci. Med. 5, 60–73.
James, C. R., Atkins, L. T., Dufek, J. S., and Bates, B. T. (2014). An exploration of
load accommodation strategies during walking with extremity carried weights.
Hum. Movement Sci. 35, 17–29. doi: 10.1016/j.humov.2014.03.012
James, C. R., and Bates, B. T. (1997). Experimental and statistical design
issues in human movement research. Meas. Phys. Educ. Exerc. Sci. 1, 55–69.
doi: 10.1207/s15327841mpee0101_4
James, C. R., Bates, B. T., and Dufek, J. S. (2003). Classification and comparison of
biomechanical response strategies for accommodating landing impact. J. App.
Biomech. 19, 106–118. doi: 10.1123/jab.19.2.106
Jaric, S., and Latash, M. L. (1999). Learning a pointing task with a
kinematically redundant limb: emerging synergies and patterns of final position
variability. Hum. Movement Sci. 18, 819–838. doi: 10.1016/S0167-9457(99)0
0042-1
Jolliffe, I. T. (2002). “Graphical representation of data using principal components,”
in Principal Component Analysis. Springer Series in Statistics, 2nd Edn (New
York, NY: Springer), 78–110.
Jolliffe, I. T., and Cadima, J. (2016). Principal component analysis: a
review and recent development. Phil. Trans. R. Soc. 374:20150202.
doi: 10.1098/rsta.2015.0202
Ketcham, C. J., Seidler, R. D., van Gemmert, A. W. A., and Stelmach, G. E. (2002).
Age related kinematic differences as influenced by task difficulty, target size and
movement amplitude. J. Gerontol. 57, 54–64. doi: 10.1093/geronb/57.1.P54
Kipp, K., Redden, J., Sabick, M., and Harris, C. (2012). Kinematic and kinetic
synergies of the lower extremities during the pull in olympic weightlifting. J.
App. Biomech. 28, 271–278. doi: 10.1123/jab.28.3.271
Kollias, I., Hatzitaki, V., Papaiakovou, G., and Giatsis, G. (2001). Using
principal components analysis to identify individual differences
in vertical jump performance. Res. Q. Exerc. Sport. 72, 63–67.
doi: 10.1080/02701367.2001.10608933
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 10 August 2019 | Volume 7 | Article 193
Cushion et al. PCA of Vertical Jumping
Laffaye, G., Bardy, B. G., and Durey, A. (2007). Principal component structure and
sport specific differences in the running on leg vertical jump. Int. J. Sports. Med.
28, 420–425. doi: 10.1055/s-2006-924507
Lamoth, C. J. C., Daffertshofer, A., Meijer, O. G., and Beek, P. J. (2006). How do
persons with chronic low back pain speed up and slow down? trunk-pelvis
coordination and lumbar erector spinae activity during gait. Gait Posture. 23,
230–239. doi: 10.1016/j.gaitpost.2005.02.006
Latash, M. (2000). There is no motor redundancy in human movements. There is
motor abundance. Motor Control. 4, 259–261. doi: 10.1123/mcj.4.3.259
Latash, M. (2010). Motor synergies and the equilibrium point hypothesis. Motor
Control. 14, 294–322. doi: 10.1123/mcj.14.3.294
Latash, M., Scholz, J. P., and Schoner, G. (2007). Toward a new theory of motor
synergies. Motor Control. 11, 276–308. doi: 10.1123/mcj.11.3.276
Lee, M., Roan, M., and Smith, B. (2009). An application of principal component
analysis for lower body kinematics between loaded and unloaded walking. J.
Biomech. 42, 2226–2230. doi: 10.1016/j.jbiomech.2009.06.052
Lees, A., Vanrenterghem, J., and De Clercq, D. (2004). Understanding how an arm
swing enhances performance in the vertical jump. J. Biomech. 37, 1929–1940.
doi: 10.1016/j.jbiomech.2004.02.021
Majed, L., Heugas, A. M., and Siegler, I. A. (2017). Changes in movement
organization and control strategies when learning a biomechanically
constrained gait pattern, racewalking: a PCA study. Exp. Brain. Res. 235,
931–940. doi: 10.1007/s00221-016-4853-8
Newell, K. M. (1986). “Constraints on the development of coordination,” in Motor
Development in Children: Aspect of Coordination and Control, eds M. G. Wade
and H. T. A. Whiting (Dordrecht: Nijhoff), 341–360.
Nordin, A. D., and Dufek, J. S. (2016a). Neuromechanical synergies in single leg
landing reveal changes in movement control. Hum. Movement Sci. 49, 66–78.
doi: 10.1016/j.humov.2016.06.007
Nordin, A. D., and Dufek, J. S. (2016b). Single leg landing neuromechanical
data following load and land height manipulations. Data Brief 8, 1024–1030.
doi: 10.1016/j.dib.2016.07.011
Nordin, A. D., and Dufek, J. S. (2017). Load accommodation strategies and
movement variability in single leg landing. J. App. Biomech. 33, 241–247.
doi: 10.1123/jab.2016-0097
Nordin, A. D., and Dufek, J. S. (2019). Reviewing the variability-overuse injury
hypothesis: does movement variability relate to landing injuries? Res. Q. Exerc.
Sport. 90, 190–205. doi: 10.1080/02701367.2019.1576837
Nordin, A. D., Dufek, J. S., James, C. R., and Bates, B. T. (2017). Classifying
performer strategies in drop landing activities. J. Sports. Sci. 35, 1858–1863.
doi: 10.1080/02640414.2016.1240876
Orth, D., Davids, K., and Seifert, L. (2018). Constraints representing a meta-
stable regime facilitate exploration during practice and transfer of learning
in a complex multi-articular task. Hum. Movement Sci. 57, 291–302.
doi: 10.1016/j.humov.2017.09.007
Raffalt, P. C., Alkjaer, T., and Simonsen, E. B. (2016). Intra and inter
subject variation in lower limb coordination during countermovement
jumps in children and adults. Hum. Movement Sci. 46, 63–77.
doi: 10.1016/j.humov.2015.12.004
Richter, C., O’Connor, N. E., Marshall, B., and Moran, K. (2014). Comparison
of discrete point vs dimensionality reduction techniques for describing
performance related aspects of maximal vertical jumping. J. Biomech. 47,
3012–3017. doi: 10.1016/j.jbiomech.2014.07.001
Santello, M., Flanders, M., and Soechting, J. F. (1998). Postural
hand synergies for tool use. J. Neurosci. 18, 10105–10115.
doi: 10.1523/JNEUROSCI.18-23-10105.1998
Scholz, J., Schoner, G., and Latash, M. (2000). Identifying the control structure of
multijoint coordination during pistol shooting. Exp. Brain. Res. 135, 382–404.
doi: 10.1007/s002210000540
Scholz, J. P., Reisman, D., and Schoner, G. (2001). Effects of varying task
constraints on solutions to joint coordination in a sit to stand task. Exp. Brain.
Res. 141, 485–500. doi: 10.1007/s002210100878
Scholz, J. P., and Schoner, G. (1999). The uncontrolled manifold concept:
identifying control variables for a functional task. Exp. Brain. Res. 126, 289–306.
doi: 10.1007/s002210050738
Seifert, L., Chollet, D., and Rouard, A. (2007). Swimming constraints
and arm coordination. Hum. Movement Sci. 26, 68–86.
doi: 10.1016/j.humov.2006.09.003
Seifert, L., Leblanc, H., Herault, R., Komar, J., Button, C., and Chollet, D.
(2011). Inter-individual variability in the upper lower limb breaststroke
coordination. Hum. Movement Sci. 30, 550–565. doi: 10.1016/j.humov.201
0.12.003
Soechting, J. F., and Flanders, M. (1997). Flexibility and repeatability of finger
movements during typing: analysis of multiple degrees of freedom. J. Comput.
Neurosci. 4, 29–46. doi: 10.1023/A:1008812426305
St-Onge, N., Duval, N., Yahia, L.’H., and Feldman, A. G. (2004). Interjoint
coordination in lower limbs in patients with a rupture of the anterior cruciate
ligament of the knee joint. Knee. Surg. Sports. Traumatol. Arthrosc. 12, 203–216.
doi: 10.1007/s00167-003-0420-5
Todorov, E., and Ghahramani, Z. (2004). “Analysis of the synergies underlying
complex hand manipulation,” in The 26th Annual International Conference of
the IEEE Engineering in Medicine and Biology Society, Vol. 2 (San Francisco,
CA: IEEE), 4637–4640. doi: 10.1109/IEMBS.2004.1404285
Troje, N. F. (2002). Decomposing biological motion: a framework for analysis and
synthesis of human gait patterns. J. Vis. 2:2. doi: 10.1167/2.5.2
Verrel, J., Pologe, S., Manselle, W., Lindenberger, U., and Woollacott,
M. (2013). Coordination of degrees of freedom and stabilization of
task variables in a complex motor skill: expertise-related differences in
cello bowing. Exp. Brain. Res. 224, 323–334. doi: 10.1007/s00221-012-
3314-2
Winter, D. A. (2005). Biomechanics and Motor Control of Human Movement. 3rd
ed. Hoboken, NJ; John Wiley & Sons, Inc.
Witte, K., Ganter, N., Baumgard, C., and Peham, C. (2010). Applying a principal
component analysis to movement coordination in sport. MCMDS 16, 477–488.
doi: 10.1080/13873954.2010.507079
Witte, K., Schobesberger, H., and Peham, C. (2009). Motion pattern analysis of
gait in horseback riding by means of principal component analysis. Hum.
Movement Sci. 28, 394–405. doi: 10.1016/j.humov.2009.04.002
Wootten, M. E., Kadaba, M. P., and Cochran, G. V. B. (1990). Dynamic
electromyography. I. Numerical representation using principal
component analysis. J. Orthop. Res. 8, 247–258. doi: 10.1002/jor.11000
80214
Zago, M., Pacifici, I., Lovecchio, N., Galli, M., Federolf, P. A., and Sforza,
C. (2017). Multi-segmental movement patterns reflect juggling complexity
and skill level. Hum. Movement Sci. 54, 144–153. doi: 10.1016/j.humov.201
7.04.013
Conflict of Interest Statement: The authors declare that the research was
conducted in the absence of any commercial or financial relationships that could
be construed as a potential conflict of interest.
Copyright © 2019 Cushion, Warmenhoven, North and Cleather. This is an open-
access article distributed under the terms of the Creative Commons Attribution
License (CC BY). The use, distribution or reproduction in other forums is permitted,
provided the original author(s) and the copyright owner(s) are credited and that the
original publication in this journal is cited, in accordance with accepted academic
practice. No use, distribution or reproduction is permitted which does not comply
with these terms.
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 11 August 2019 | Volume 7 | Article 193
ORIGINAL RESEARCH
published: 08 August 2019
doi: 10.3389/fbioe.2019.00193
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 1August 2019 | Volume 7 | Article 193
Edited by:
Veronica Cimolin,
Politecnico di Milano, Italy
Reviewed by:
Francesco Travascio,
University of Miami, United States
Andrew D. Nordin,
University of Florida, United States
*Correspondence:
Emily J. Cushion
emily[email protected]
Daniel J. Cleather
Specialty section:
This article was submitted to
Biomechanics,
a section of the journal
Frontiers in Bioengineering and
Biotechnology
Received: 20 December 2018
Accepted: 24 July 2019
Published: 08 August 2019
Citation:
Cushion EJ, Warmenhoven J,
North JS and Cleather DJ (2019)
Principal Component Analysis Reveals
the Proximal to Distal Pattern in
Vertical Jumping Is Governed by Two
Functional Degrees of Freedom.
Front. Bioeng. Biotechnol. 7:193.
doi: 10.3389/fbioe.2019.00193
Principal Component Analysis
Reveals the Proximal to Distal
Pattern in Vertical Jumping Is
Governed by Two Functional Degrees
of Freedom
Emily J. Cushion 1
*, John Warmenhoven 2, Jamie S. North 1and Daniel J. Cleather 1
*
1Faculty of Sport, Health and Applied Science, St Mary’s University, Twickenham, United Kingdom, 2Exercise and Sports
Science, Faculty of Health Sciences, The University of Sydney, Lidcombe, NSW, Australia
The successful completion of motor tasks requires effective control of multiple degrees
of freedom (DOF), with adaptations occurring as a function of varying performance
constraints. In this study we sought to compare the emergent coordination strategies
employed in vertical jumping under different task constraints [countermovement jump
(CMJ) with arm swing-CMJas and no arm swing-CMJnas]. In order to achieve this,
principal component analysis (PCA) was conducted on joint moment waveform data
from the hip, knee and ankle. This statistical approach has the advantage of analyzing
the whole movement within a time series and reduces multidimensional datasets to
lower dimensions for analysis. Both individual and group analyses were conducted.
For individual analysis, PCA was conducted on combined hip, knee, and ankle joint
moment data for each individual across both CMJnas (thirty-eight participants), and
CMJas (twenty-two participants) conditions. PCA was also performed comparing all
data from each individual across CMJnas and CMJas conditions. The results revealed a
maximum of three principal components (PC) explained over 90% of the variance in the
data sets for both conditions and within individual and group analyses. For individual
analysis, no more than 2PCs were required for both conditions. For group analysis,
CMJas required 3PCs to explain over 90% of the variance within the dataset and CMJnas
only required 2PCs. Reconstruction of the original NJM waveforms from the PCA output
demonstrates a greater loading of hip and knee joint moments to PC1, with PC2 showing
a greater loading to ankle joint moment. The reduction in dimensions of the original data
shows the proximal to distal extension pattern in the sagittal plane, typical of vertical
jumping tasks, is governed by only 2 functional DOF, at both a group, and individual
level, rather than the typically reported 3 mechanical DOF in some forms of jumping.
Keywords: principal component analysis, vertical jumping, degrees of freedom, constraints, proximal to distal
pattern
Cushion et al. PCA of Vertical Jumping
INTRODUCTION
In both day-to-day and sporting contexts, human
beings consistently perform complex motor actions. Whether
this is walking up and down flights of stairs at home or
performing jumping actions in sport, people are able to perform
such skills with relative ease. Yet underpinning these observable
actions is a need to coordinate and control multiple degrees
of freedom (DOF), referred to as “the degrees of freedom
problem” by Bernstein (1967). With so many DOF within
the motor system, there are an almost limitless number of
coordination patterns available to the performer. However,
according to theoretical principles from ecological psychology,
and dynamical systems theory, it is proposed that the performer
seeks to satisfy the goal of the task whilst operating under
continually interacting task, environmental, and organismic
constraints, through which coordinated patterns of behavior
emerge (Newell, 1986; Hristovski et al., 2006; Orth et al., 2018).
Critical, therefore, in successfully completing such tasks is the
need to control the “redundant” DOF (Bernstein, 1967; Latash,
2000). These “redundant” DOF, however, provide important
functionality as they enable adaptation of emerging actions
to the varying performance constraints under which they are
operating. For example, Chow et al. (2008) demonstrated that
participants adapted their use of limb segments to continue
successfully performing a soccer chipping task whilst the task
constraints (which we define here as goals or rules which are
imposed that influence the movement) were manipulated.
Such a finding evidences how the redundant DOF allow for
functional variability and for performers to adapt to ever
changing performance constraints. Whilst there has been much
work within this area it is common for only kinematic changes
under varying constraints to be considered (e.g., Ketcham et al.,
2002; Seifert et al., 2007; Majed et al., 2017). However, analyzing
kinetic factors, such as forces and joint moments, would provide
a more complete understanding of how emerging behaviors are
shaped as a function of the task constraints under which the skill
is performed.
Explaining the control strategies adopted by performers has
been a topic within the motor control literature for many
years (see Dufek et al., 1995; Bates, 1996; James and Bates,
1997; James et al., 2003, 2014; Nordin and Dufek, 2019). It
has been suggested that certain movement features are more
important to satisfy the goal of the task, and therefore these
features are less likely to show variance between repetitions
or from person to person (Scholz and Schoner, 1999; Scholz
et al., 2000). This has been demonstrated using several tasks
(see Button et al., 2003; Seifert et al., 2011; Nordin et al.,
2017). For instance, elbow angle at ball release in a basketball
shooting task showed lesser variability between individuals of
varying skill levels, compared to other features such as wrist
angle at ball release (Button et al., 2003), which indicates that
elbow angle at ball release is an important movement feature
for successful performance in this task. Identification of such
movement features aids in developing our understanding of
motor control strategies employed to govern movements under
varying task constraints.
Traditional approaches to the study of human movement
have typically relied on selecting discrete data points for
analysis. However, these methods may not provide a complete
representation of the complexities of motor actions due to
data being discarded outside of those discrete points. Instead,
methods which analyse data across the full temporal cycle of the
movement, such as principal component analysis (PCA), may
prove more informative (Richter et al., 2014). The attraction
of PCA is that large amounts of data across movement cycles
can be analyzed whilst reducing the dimensionality of data to
features of importance (Daffertshofer et al., 2004). This statistical
approach has been used to determine key characteristics of
movement tasks (see for example Soechting and Flanders, 1997;
Kollias et al., 2001; Lamoth et al., 2006; Dona et al., 2009;
Witte et al., 2010; Federolf et al., 2013; Nordin and Dufek,
2016a) as well as determining similarities and differences between
groups through data filtering (see for example Deluzio et al.,
1997; Deluzio and Astephen, 2007; Laffaye et al., 2007; Lee
et al., 2009; Federolf et al., 2013; Verrel et al., 2013). Despite
the growth of PCA in sports sciences recently, its application
is still in its relative infancy. In particular, fewer researchers
have used this approach to determine coordination patterns
within movements or to compare movements under differing
task constraints (see Forner-Cordero et al., 2005; Lee et al.,
2009; Nordin and Dufek, 2016b; Majed et al., 2017 for some
exceptions). Therefore, applying a statistical approach such as
PCA can be useful in reducing large datasets to key movement
features and may be more effective in showing how movement
emerges under changing constraints.
Vertical jumping is an interesting motor task to study as
it requires the effective coordination of the upper and lower
limbs to raise the center of mass vertically, with a clear goal
of jumping for height (Raffalt et al., 2016). Vertical jumping
also represents a task which can be easily manipulated to
provide insight into how emergent behaviors adapt to differing
conditions. Analysis of movements under constrained conditions
can lead to a better understanding of the key mechanisms for
efficient movement, such as the requirement to keep balance in
a sit to stand task (Scholz et al., 2001) or the accommodation
strategies with increased task demands (Nordin and Dufek,
2016b, 2017). With this in mind, this study used a vertical
jumping task and asked participants to complete this action
under two different task constraints (with arm swing and without
arm swing), with the aim of understanding how motor control
strategies, and emergent coordination patterns were affected
by manipulation of these constraints. To fully understand
these coordination strategies and overcome the limitations
associated with traditional analysis methods, we employed PCA
to determine the principal components (PCs) that characterize
vertical jumping movement patterns both between and within
individuals and across the two task constraints. Specifically, we
aimed to answer the question of the number of PCs expected
to describe either a single jump, repetitions of a jump from an
individual, and across the whole group. Typically, lower limb
coordination in jumping tasks is described as an extension of
the lower limbs in a proximal to distal fashion, with the peak
moment progressing temporally from hip, to knee, and then
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 2August 2019 | Volume 7 | Article 193
Cushion et al. PCA of Vertical Jumping
ankle (Bobbert and van Ingen Schenau, 1988). A moment curve
is typically bell-shaped and unimodal (examples can be seen in
Figures 6,7). If the timing of peak moments and the shape of
the moment curves are independent of one another it would be
expected that 3 PCs would be required to represent the 3 moment
curves of a particular jump (that is 3 functional DOF). If the peaks
of the 3 moment curves occur at different time points along the
curve, then there needs to be more than one PC score.
MATERIALS AND METHODS
Participants
Thirty-eight healthy individuals (males =24, females =14)
volunteered to take part in this study (mean ±SD; age =
27 ±5 years, height =174.4 ±9.0 cm, body mass 78.1 ±
14.1 kg). Participants were free from musculoskeletal injuries and
were provided with details of the study before written informed
consent was obtained. The experimental procedure was approved
by the ethics sub-committee at the institution where the research
took place.
Procedure
Participants were required to attend one data collection session.
This involved the collection of anthropometric measures (height
and weight), before each participant was provided with a
standardized shoe according to their shoe size. Eighteen
reflective markers were placed on the pelvis and on the right
lower limb. Data from the right limb was used for further
analysis in accordance with previous work from Cleather et al.
(2013). Markers were placed on the right and left anterior
superior iliac spine and posterior superior iliac spine, lateral
and medial femoral epicondyle, apex of lateral and medial
malleolus, posterior aspect of calcaneus, tuberosity of fifth
metatarsal, and head of second metatarsal. Three additional
markers placed on rigid plates were attached to the mid-
thigh and anterior tibial shaft, with an additional marker
attached to the top of the foot. Kinematic data was collected
using a Vicon motion capture system (Vicon MX System,
Nexus 2.2 software, Vicon Motion Systems Ltd, Oxford, UK)
with 14 LED cameras tracking the reflective markers at a
sampling frequency of 200 Hz. Kinetic data was collected via
two force plates positioned flush to the laboratory floor (Kistler
Type 9287BA, Bioware 3.24 software, Kistler Instruments Ltd,
Hampshire, UK), at a rate of 1,000 Hz and synchronized with the
Vicon system.
Participants completed a standardized warm-up (bodyweight
squats, lunges, inchworms, hip rotations, and vertical jumps)
prior to completing any vertical jumps. Thirty-eight participants
performed a vertical jump task (countermovement jump with no
arm swing—CMJnas). For this task, participants were instructed
to keep hands in contact with the hip throughout the jump,
and to land with one foot on each force plate. Participants were
required to complete five maximal effort trials with a self-selected
recovery period between each jump to reduce any effects of
fatigue. Twenty-two of the participants carried out an additional
jumping task. For this task, participants performed a vertical
jump with the use of an arm swing (CMJas). Participants were
instructed to use an arm swing to aid in jumping performance
and were required to land with one foot on each force plate. For
these participants the order of completion of the two tasks was
counterbalanced to prevent order effects. Participants were given
a 2 min recovery period between the two tasks.
Data Analysis
All data was filtered using a 5th order Woltring filter with a
cut off frequency of 10 Hz. The propulsive phase of the vertical
jump was used for analysis and was defined as being from
the point where the right anterior superior iliac spine marker
moved below stationary height until take-off (which was defined
as the point where the ground reaction force fell to zero).
Net joint moments (NJM) in the sagittal plane were calculated
for hip, knee, and ankle during this phase using a standard
inverse dynamics calculation (Winter, 2005) within the FreeBody
software (Cleather and Bull, 2015). Each jump trial therefore had
the 3 mechanical DOF described by the NJM.
As trial length varied across each participant, data was spline
interpolated and time normalized from 0 to 101 data points.
Maximal jump height was analyzed through calculation of the
change in displacement of the right anterior superior iliac spine
when standing, to the maximum height achieved during the jump
(Chiu and Salen, 2010).
PCA Calculation
PCA was used in this study to extract common patterns of
moment production during the vertical jump under two task
constraints. Using this approach has the advantage of retaining
the spatiotemporal pattern in the time series data whilst detecting
coordination patterns both within and between individuals. The
fundamental purpose of a PCA is to find a linear transformation
that maps the raw data described in its original coordinate
frame to a new coordinate frame with orthonormal bases. In
the context of data analysis, the coordinate frame for the raw
data is defined by the measured variables, but these variables
may have some degree of correlation with one another. The
new coordinate frame that is given by the PCA will be defined
by a set of new uncorrelated variables called the principle
components (PC). For instance, for a dataset consisting of p
variables observed at ndifferent time-points the raw data can
be described by the n×pmatrix Xwhere the columns of
Xare the individual variables, and the rows represent each
observation (time-point). The transformation Uthen maps the
raw data to the new coordinate frame defined by the PCs,
such that the raw data in the new coordinate frame Z, is given
by Z=XU.
In biomechanics, PCA has sometimes been used to compare
time-normalized waveforms. For instance, a waveform can be
described by the value of a variable sampled at 1% intervals over
the course of a movement. Typically, we have multiple waveforms
(cases) for one particular biomechanical variable which we want
to compare—for instance, if we want to compare the curves
of different individuals. In this instance, as outlined extensively
in Deluzio and Astephen (2007), the individual time-points
have often been considered as variables and cases (observations)
considered to be the individual curves being analyzed. Thus if
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 3August 2019 | Volume 7 | Article 193
Cushion et al. PCA of Vertical Jumping
we had pdifferent curves for a given variable, that each consists
of 101 time-points, we would perform the PCA on the p×101
raw data matrix XT. In the present study we have adopted a
more intuitive approach to study waveforms that is closer to
the traditional description of PCA. We have treated the time
normalized intervals as observations, and the individual curves
(cases) as variables. Thus, for our pdifferent curves for a given
biomechanical variable sampled at 101 time-points we perform
the PCA on the 101 ×praw data matrix X. This approach has
been used previously (see Borzelli et al., 1999).
It should be noted that in the method of Deluzio and Astephen
(2007), a separate PCA is performed for each of the measured
variables. In contrast, in this study we have included all of
the measured variables within the same PCA. For instance, in
this study, for an individual subject we have time-series for 3
biomechanical variables (hip, knee, and ankle NJM) measured in
5 different jumps. Using the method of Deluzio and Astephen
(2007) we would perform 3 PCAs on the 3 5 ×101 matrices
representing each joint. Instead, in this study we perform only
one PCA on the 101 ×15 matrix which includes all of the
individual’s data.
One common application of PCA is to reduce the
dimensionality of the data being analyzed—that is to reduce the
number of variables under consideration to a smaller set which
describe the majority of the variance in the data. The advantage
of the method we have adopted here is that the coordinate frame
in which the data is described is defined by all of the cases for all
of the measured joints (NJM). This means that the PCA produces
a reduced new coordinate frame that can be used to describe
all cases and joints. This therefore means that the reduced
coordinate system represents the number of functional degrees
of freedom that are present in the movement being analyzed.
Conventional approaches to using PCA would require each
variable (e.g., hip NJM, knee NJM, ankle NJM) to be analyzed
separately. This would limit the ability to effectively interpret the
functional DOF describing the movements. Thus, for the present
study PCA was used in this manner to extract common patterns
of moment production during the vertical jump under two task
constraints. Only those PCs that cumulatively explained over
90% of the variance in the data set were retained and used in
further analysis (Jolliffe, 2002).
Prior to running the PCA, all data was normalized to the
peak hip joint moment of each trial (Jolliffe and Cadima, 2016).
Analysis of the data was performed on both an individual (termed
analysis 1), and group (termed analysis 2) basis (as has previously
been conducted within the literature, e.g., Nordin and Dufek,
2016a,b, 2017) and the PCs from the individual (PCi), and group
(PCg) analyses are indicated by subscripts as shown. For the
individual analysis a PCA was carried out for each individual
separately, which contained hip, knee and ankle NJM data
combined (101 ×15 matrix for each individual containing 15
columns representing 5 hip, 5 knee, and 5 ankle joint moment
time series with 101 data points). This was performed for both
CMJnas and CMJas conditions. For the group analysis, all NJM
data from each participant were combined and subjected to a
PCA (CMJnas: 101 data points ×567 joint moment time series,
CMJas: 101 data points ×330 joint moment trials). A further
FIGURE 1 | Variance explained by (A) PC1i, (B) PC2i, and (C) the sum of
PC1i&2i for CMJnas, and CMJas. Horizontal line represents group mean.
i=individual PCA analysis. *Indicates significant difference from CMJnas.
PCA was performed to compare CMJnas and CMJas data with
only the participants who had performed both jumps (101 data
points ×672 joint moment time-series). This is referred to as
analysis 3. Finally, an additional group level PCA was conducted
using only the first 2 PCs obtained from the individual PCA
(CMJnas: 101 data points ×76 PCs, CMJas: 101 data points ×
44 PCs; hereafter called analysis 4).
The output of each PCA was a matrix (henceforth named
the coefficients matrix) where each column gives the coefficients
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 4August 2019 | Volume 7 | Article 193
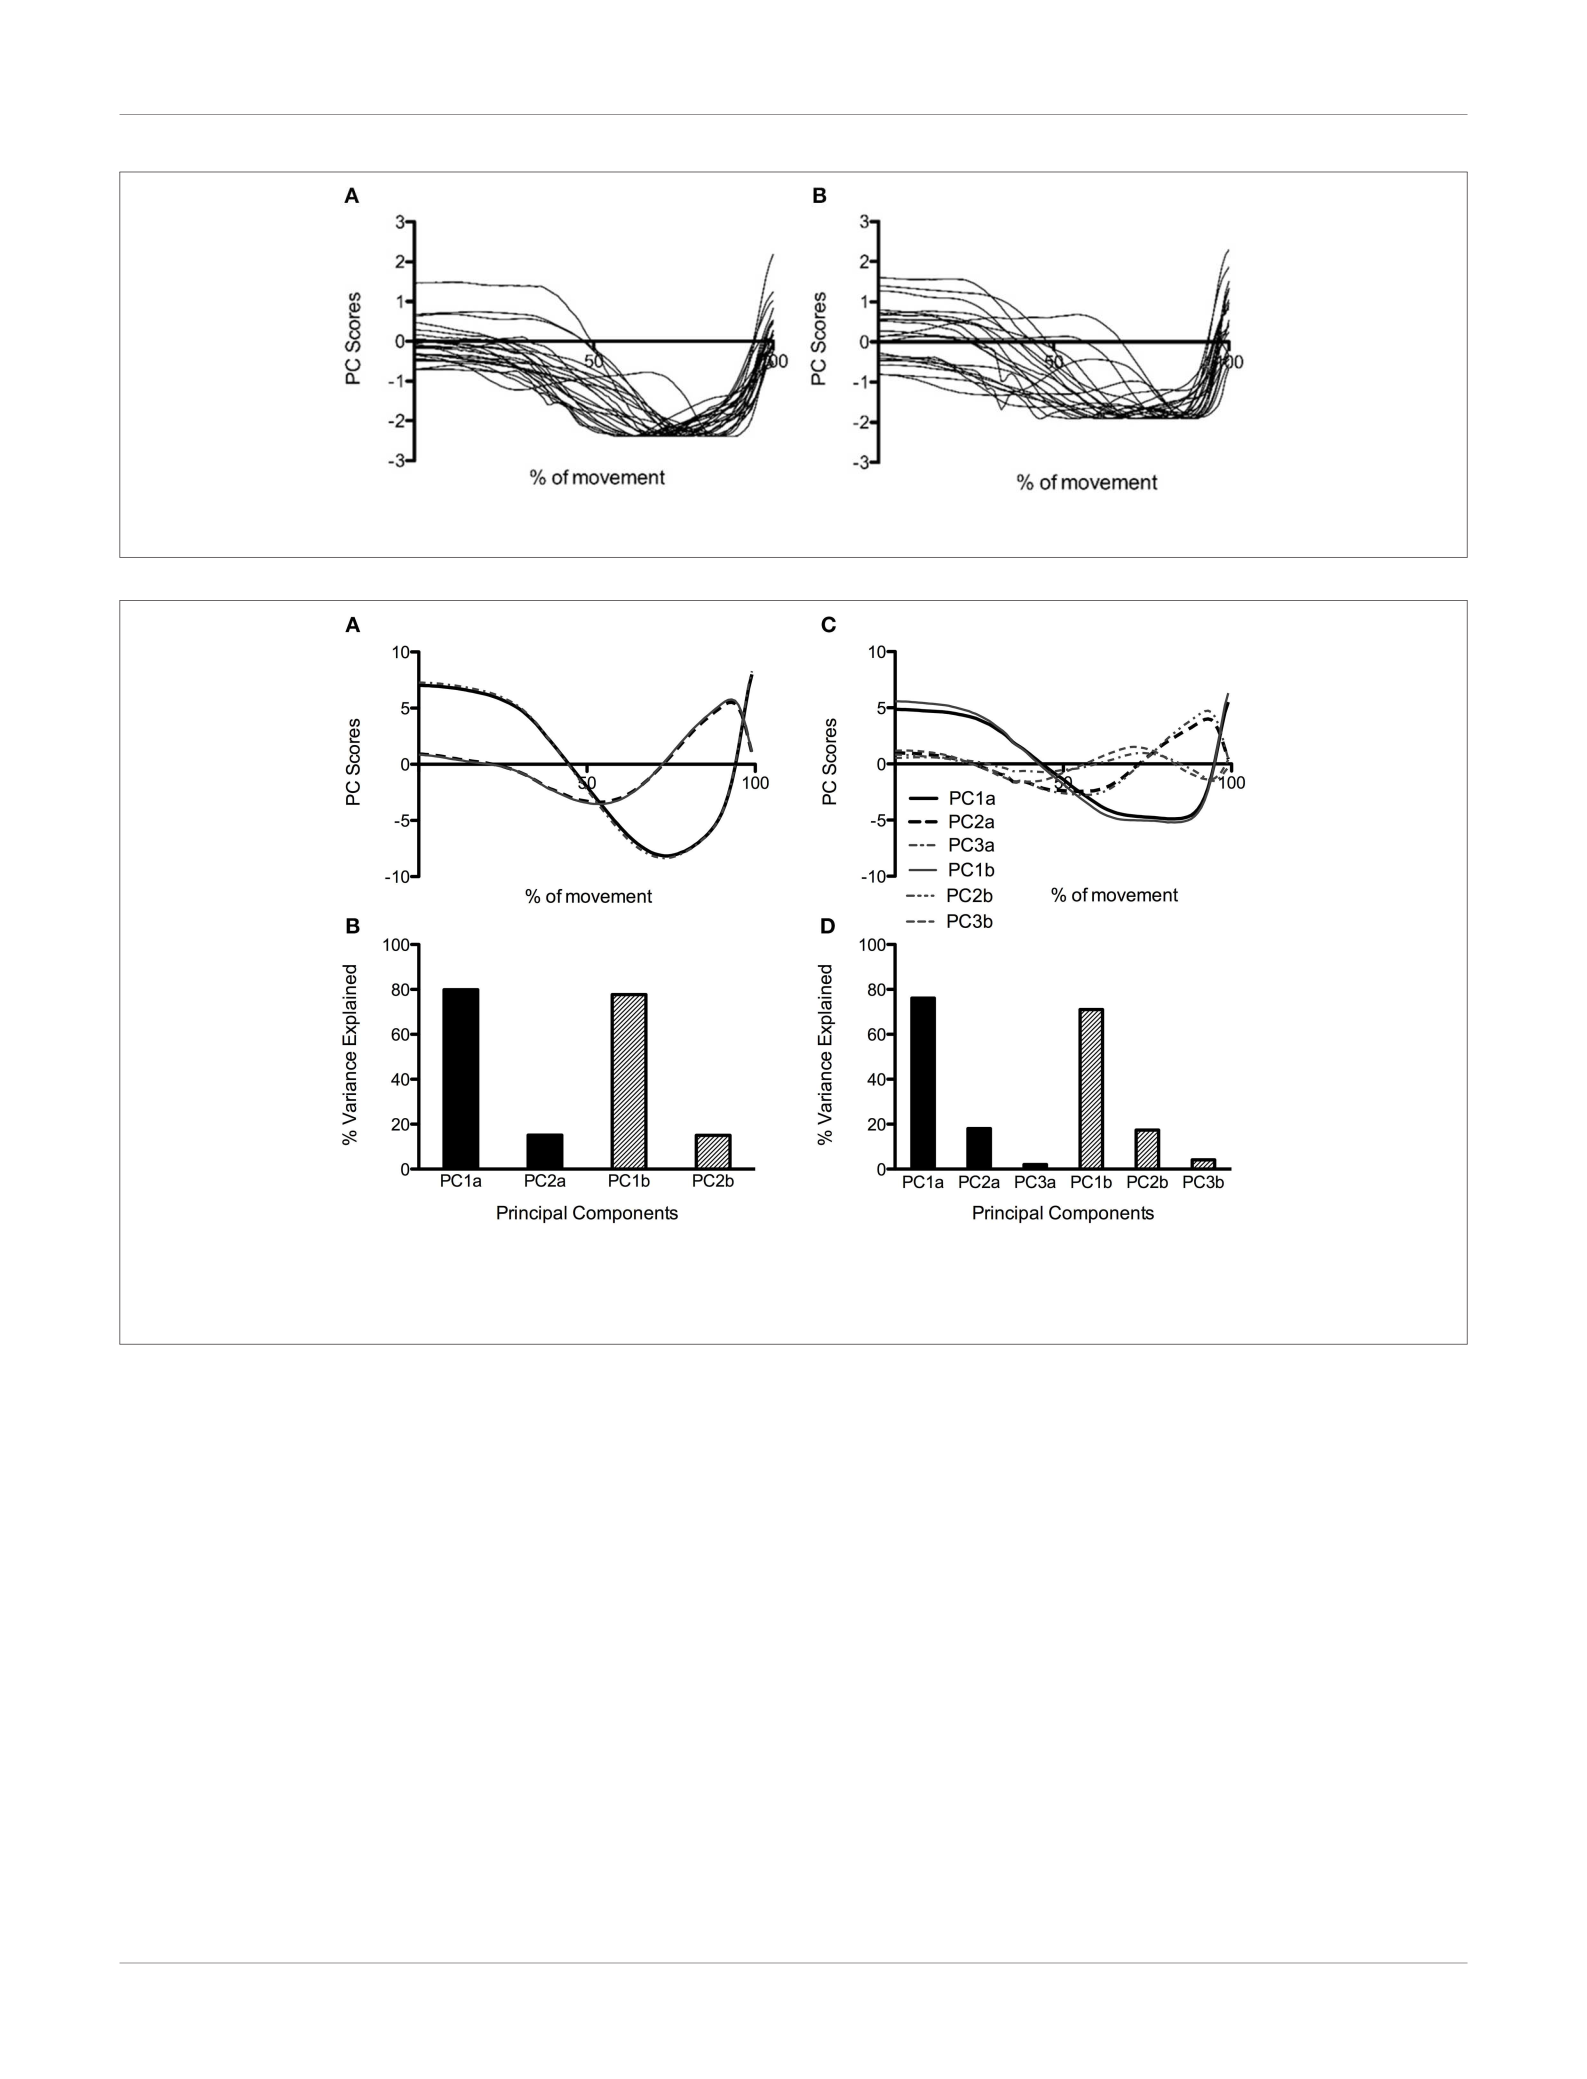
Cushion et al. PCA of Vertical Jumping
FIGURE 2 | PC1i scores for (A) CMJnas and (B) CMJas from 22 participants completing both conditions. Data is normalized to peak value. i =individual PCA analysis.
FIGURE 3 | PC waveforms along with percentage of explained variance for CMJnas (A,B) and CMJas (C,D) conditions. Data in (C) has been flipped to a negative
peak to more clearly show comparison between the shape of waveforms in (A,C). PC1, 2, and 3a represent data obtained from PCA using only the first two PCs from
each individual (analysis 4). PC1, 2, and 3b represent data obtained from group PCA for CMJnas, and CMJas (analysis 2).
of a PC, and the PCs are ordered in terms of the amount of
variance they explain. The coefficients matrix thus gives the
transformation of the raw data into the variable space defined
by the PCs. Thus, the matrix obtained by multiplying the raw
data matrix by the coefficients matrix is a matrix describing
the time-series of the values for each PC. These time series are
reported as the PC scores in this study. Similarly, the raw data
can be reconstructed based upon a limited number of PCs by
transforming the selected number of PCs back to the variable
space defined by the raw data. This was performed for CMJnas
data as an example. All PCA calculations were performed in
Matlab (The MathWorks, Inc., MA, version 2017a).
Statistical Analysis
Further statistical analysis was performed to compare the
variance explained by each PC attained from the individual
analysis of both CMJnas and CMJas. Group differences between
PC1, PC2, and the sum of PC1 and PC2 were assessed using an
independent sample t-test. The alpha level was set at p<0.05.
RESULTS
When considered individually, only one or two PCs were
required to describe at least 90% of the variance in the data.
Data from each individual PCA showed PC1i and the sum of
PC1i, and 2i explained a significantly greater amount of the
variance in CMJnas than CMJas (p=0.05, p=0.00, respectively;
Figure 1). The greater variation in PC1i scores for CMJas can be
seen in Figure 2.
When all joint moment data was combined in the same
PCA, three PCs were retained for the CMJas condition, and
two were retained for the CMJnas condition (Figure 3). Figure 3
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 5August 2019 | Volume 7 | Article 193
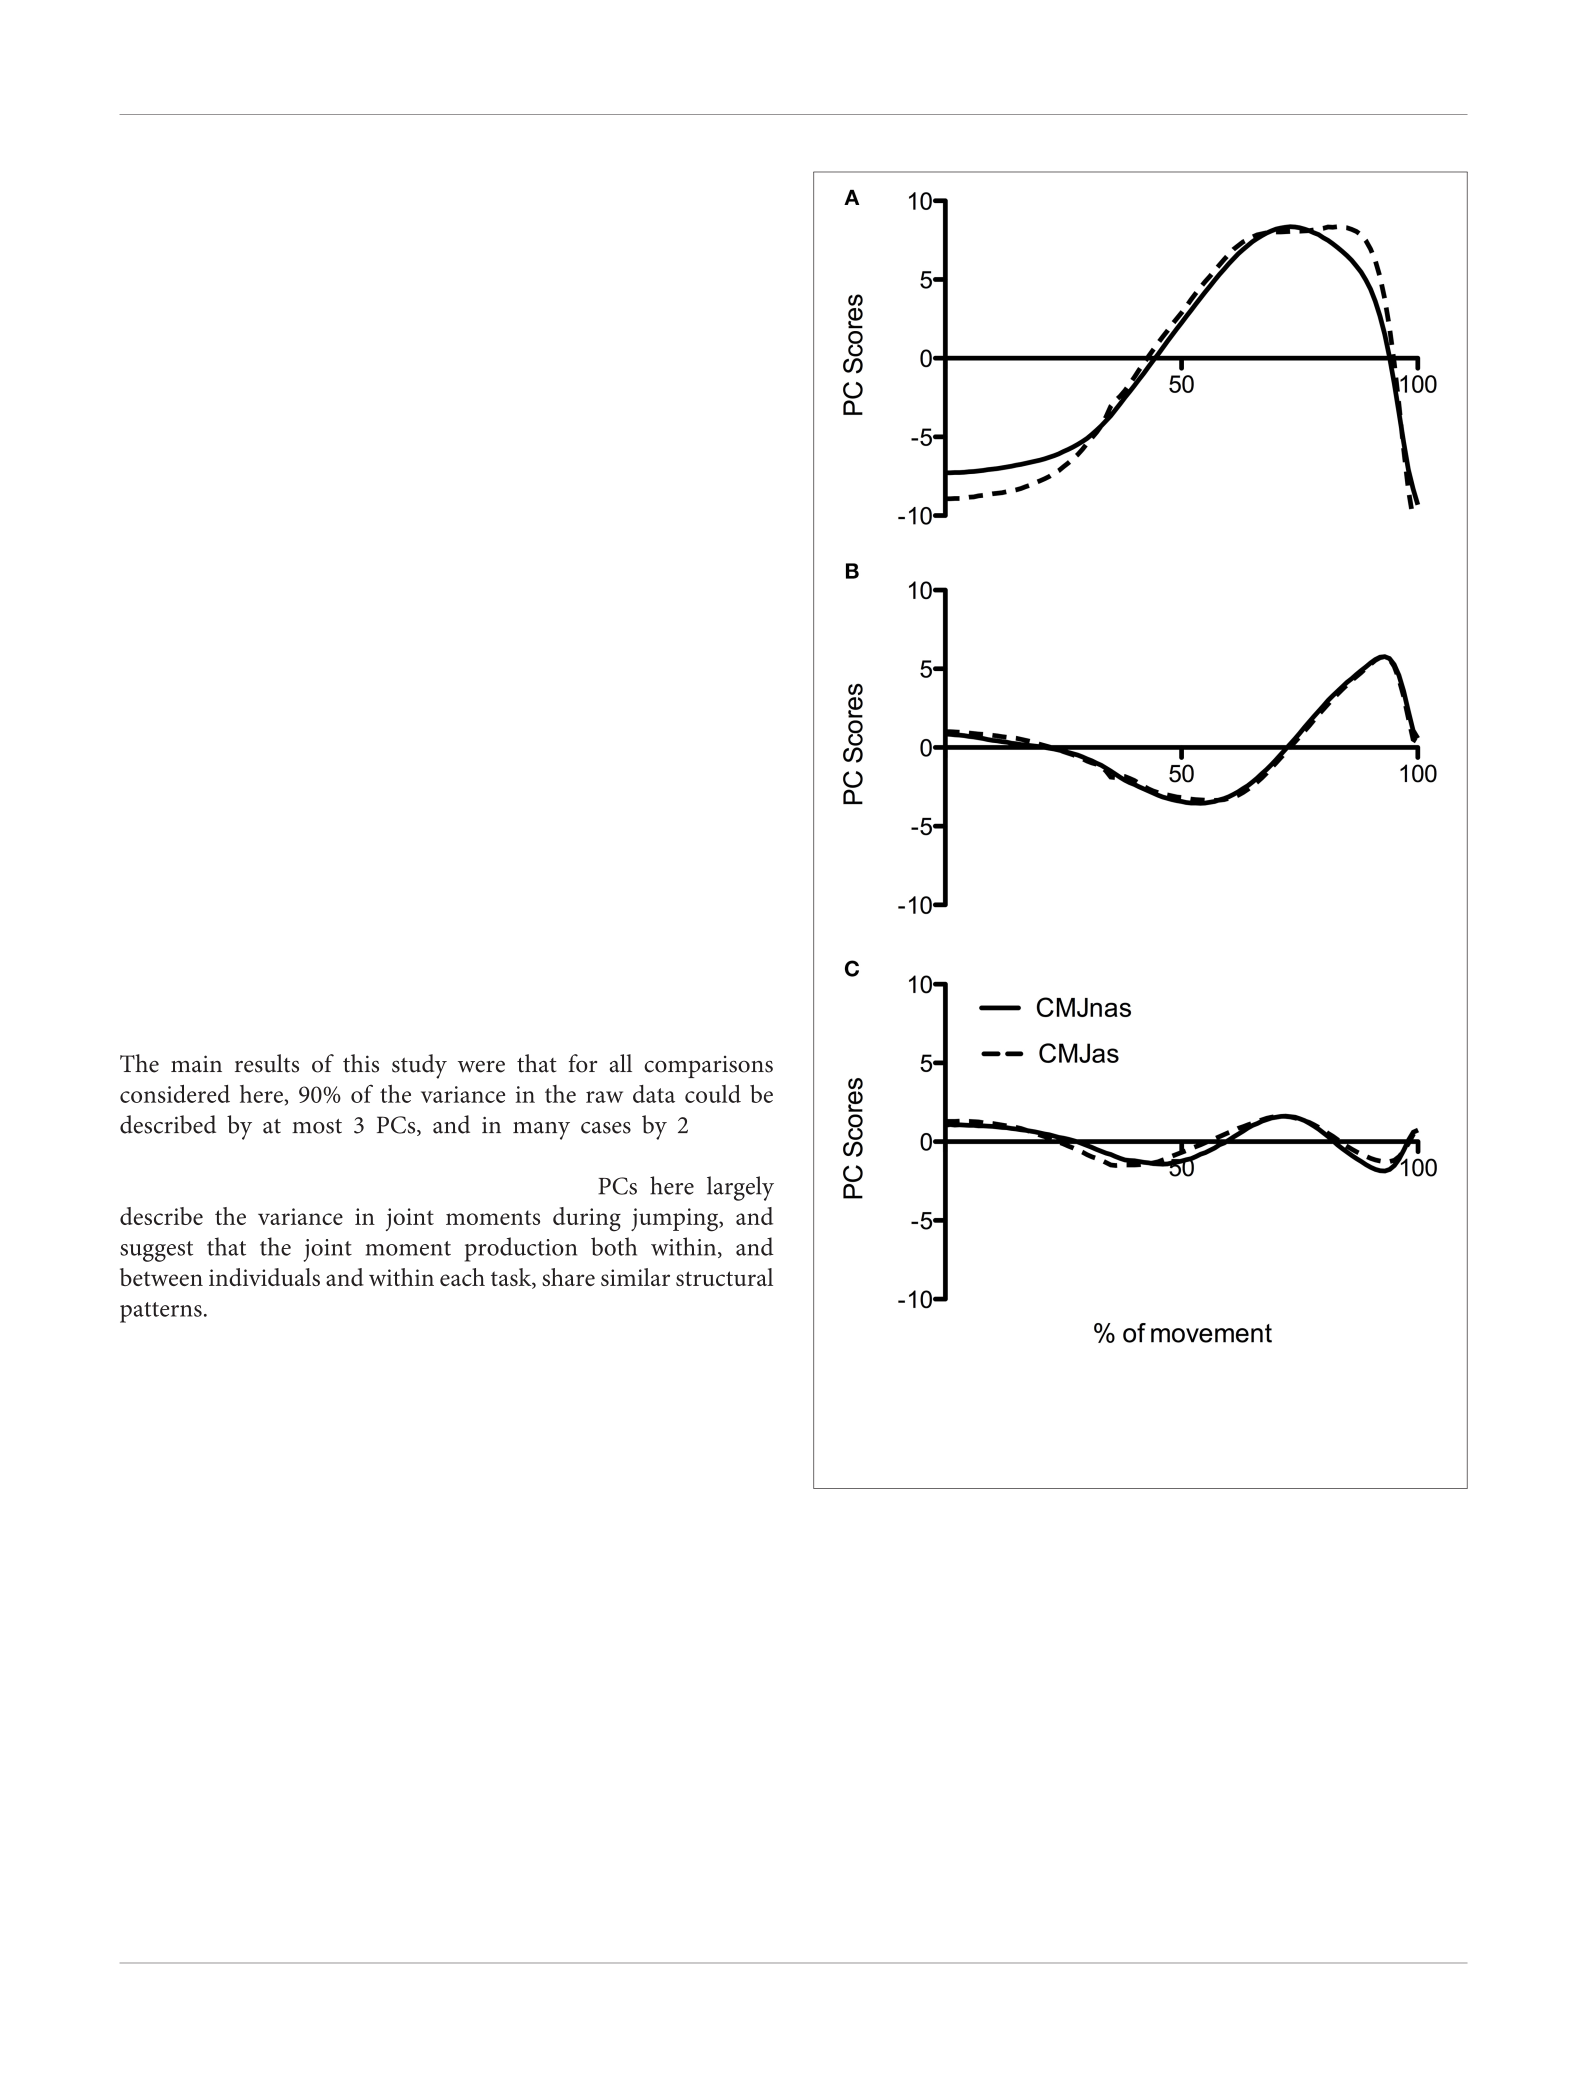
Cushion et al. PCA of Vertical Jumping
also illustrates waveforms from the group analysis PCA that just
retained the first two PCs for each individual (analysis 4).
To make a robust comparison between jumps at the group
level, data was reanalyzed with only those participants who
completed both CMJnas and CMJas conditions (Figure 4,
analysis 3). This highlighted the same trend with CMJas requiring
three PCs and CMJnas requiring only two PCs to describe over
90% of the variance. Waveforms for each jump condition were
similar to those observed in Figure 3.
An analysis was also conducted with only those participants
who completed both CMJnas and CMJas conditions with all joint
moment data combined (Figure 5). Only two PCs were required
to explain over 90% of the variance.
Figure 6 presents an illustrative example of the reconstruction
of a typical jump from PC1g and PC2g—and shows how the
sum of the time series for PC1g and PC2g describe such a high
proportion of the variance in the raw data.
Figure 7 presents an illustrative example of the reconstruction
of a series of five jumps from a representative participant
performing CMJnas. The figure shows the sum of the time series
for PC1i and PC2i describe a high proportion of the variance in
the raw data.
DISCUSSION
The purpose of this study was to use PCA to characterize
movement strategies, through reducing a large data set of
hip, knee, and ankle NJMs measured during vertical jumping.
The main results of this study were that for all comparisons
considered here, 90% of the variance in the raw data could be
described by at most 3 PCs, and in many cases by 2. Whilst
there are multiple sources of variation within the dataset (e.g.,
joint, trial, individual), we suggest that the PCs here largely
describe the variance in joint moments during jumping, and
suggest that the joint moment production both within, and
between individuals and within each task, share similar structural
patterns. Further to this, the dimensionality of sagittal plane
lower limb extension in some forms of vertical jumping can be
reduced to only 2 functional DOF. This is an important result—
it indicates that simply providing the participants with the task
constraint “jump as high as you can” produced a markedly
similar pattern, and that between and within participant variation
amounted to <10%. This is a highly non-trivial result and
provides insight to the nature of motor control within this task—
although it has previously been suggested that during jumping,
people exhibit a characteristic proximal to distal pattern of joint
moment production (Bobbert and van Ingen Schenau, 1988), the
degree of similarity has not been emphasized.
When considering the group and individual analysis for
CMJnas only 2 PCs are required to explain over 90% of
the variance (Figure 3). This would suggest the relationships
between curves are not just unique to specific individuals but are
demonstrated by the whole group. If this was not the case further
PCs would be required to describe the movement. For CMJas an
additional PC was required at the group level in order to capture
90% of the variance in the data (see Figure 3), although it was
FIGURE 4 | Comparison of PC waveforms for CMJnas and CMJas for the 22
participants who completed both jumps: (A) PC1, (B) PC2, and (C) PC3.
CMJas waveforms have been flipped and peaks matched to show differences
in temporal pattern.
not required at the individual level. These results are consistent
with previous research findings which have also looked to
determine how the high dimensionality of human movement can
be reduced to low dimensional states (see Soechting and Flanders,
1997; Borzelli et al., 1999; Balasubramaniam and Turvey, 2004;
Witte et al., 2009; Nordin and Dufek, 2016a; Majed et al., 2017),
For example, (Santello et al., 1998) have shown that in a hand
grasping task only two PCs were required to describe over 80% of
the variance in the data, demonstrating few synergies govern the
production of hand motion in the specific grasping task. Equally,
in a sit to stand task only two PCs were required to describe
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 6August 2019 | Volume 7 | Article 193
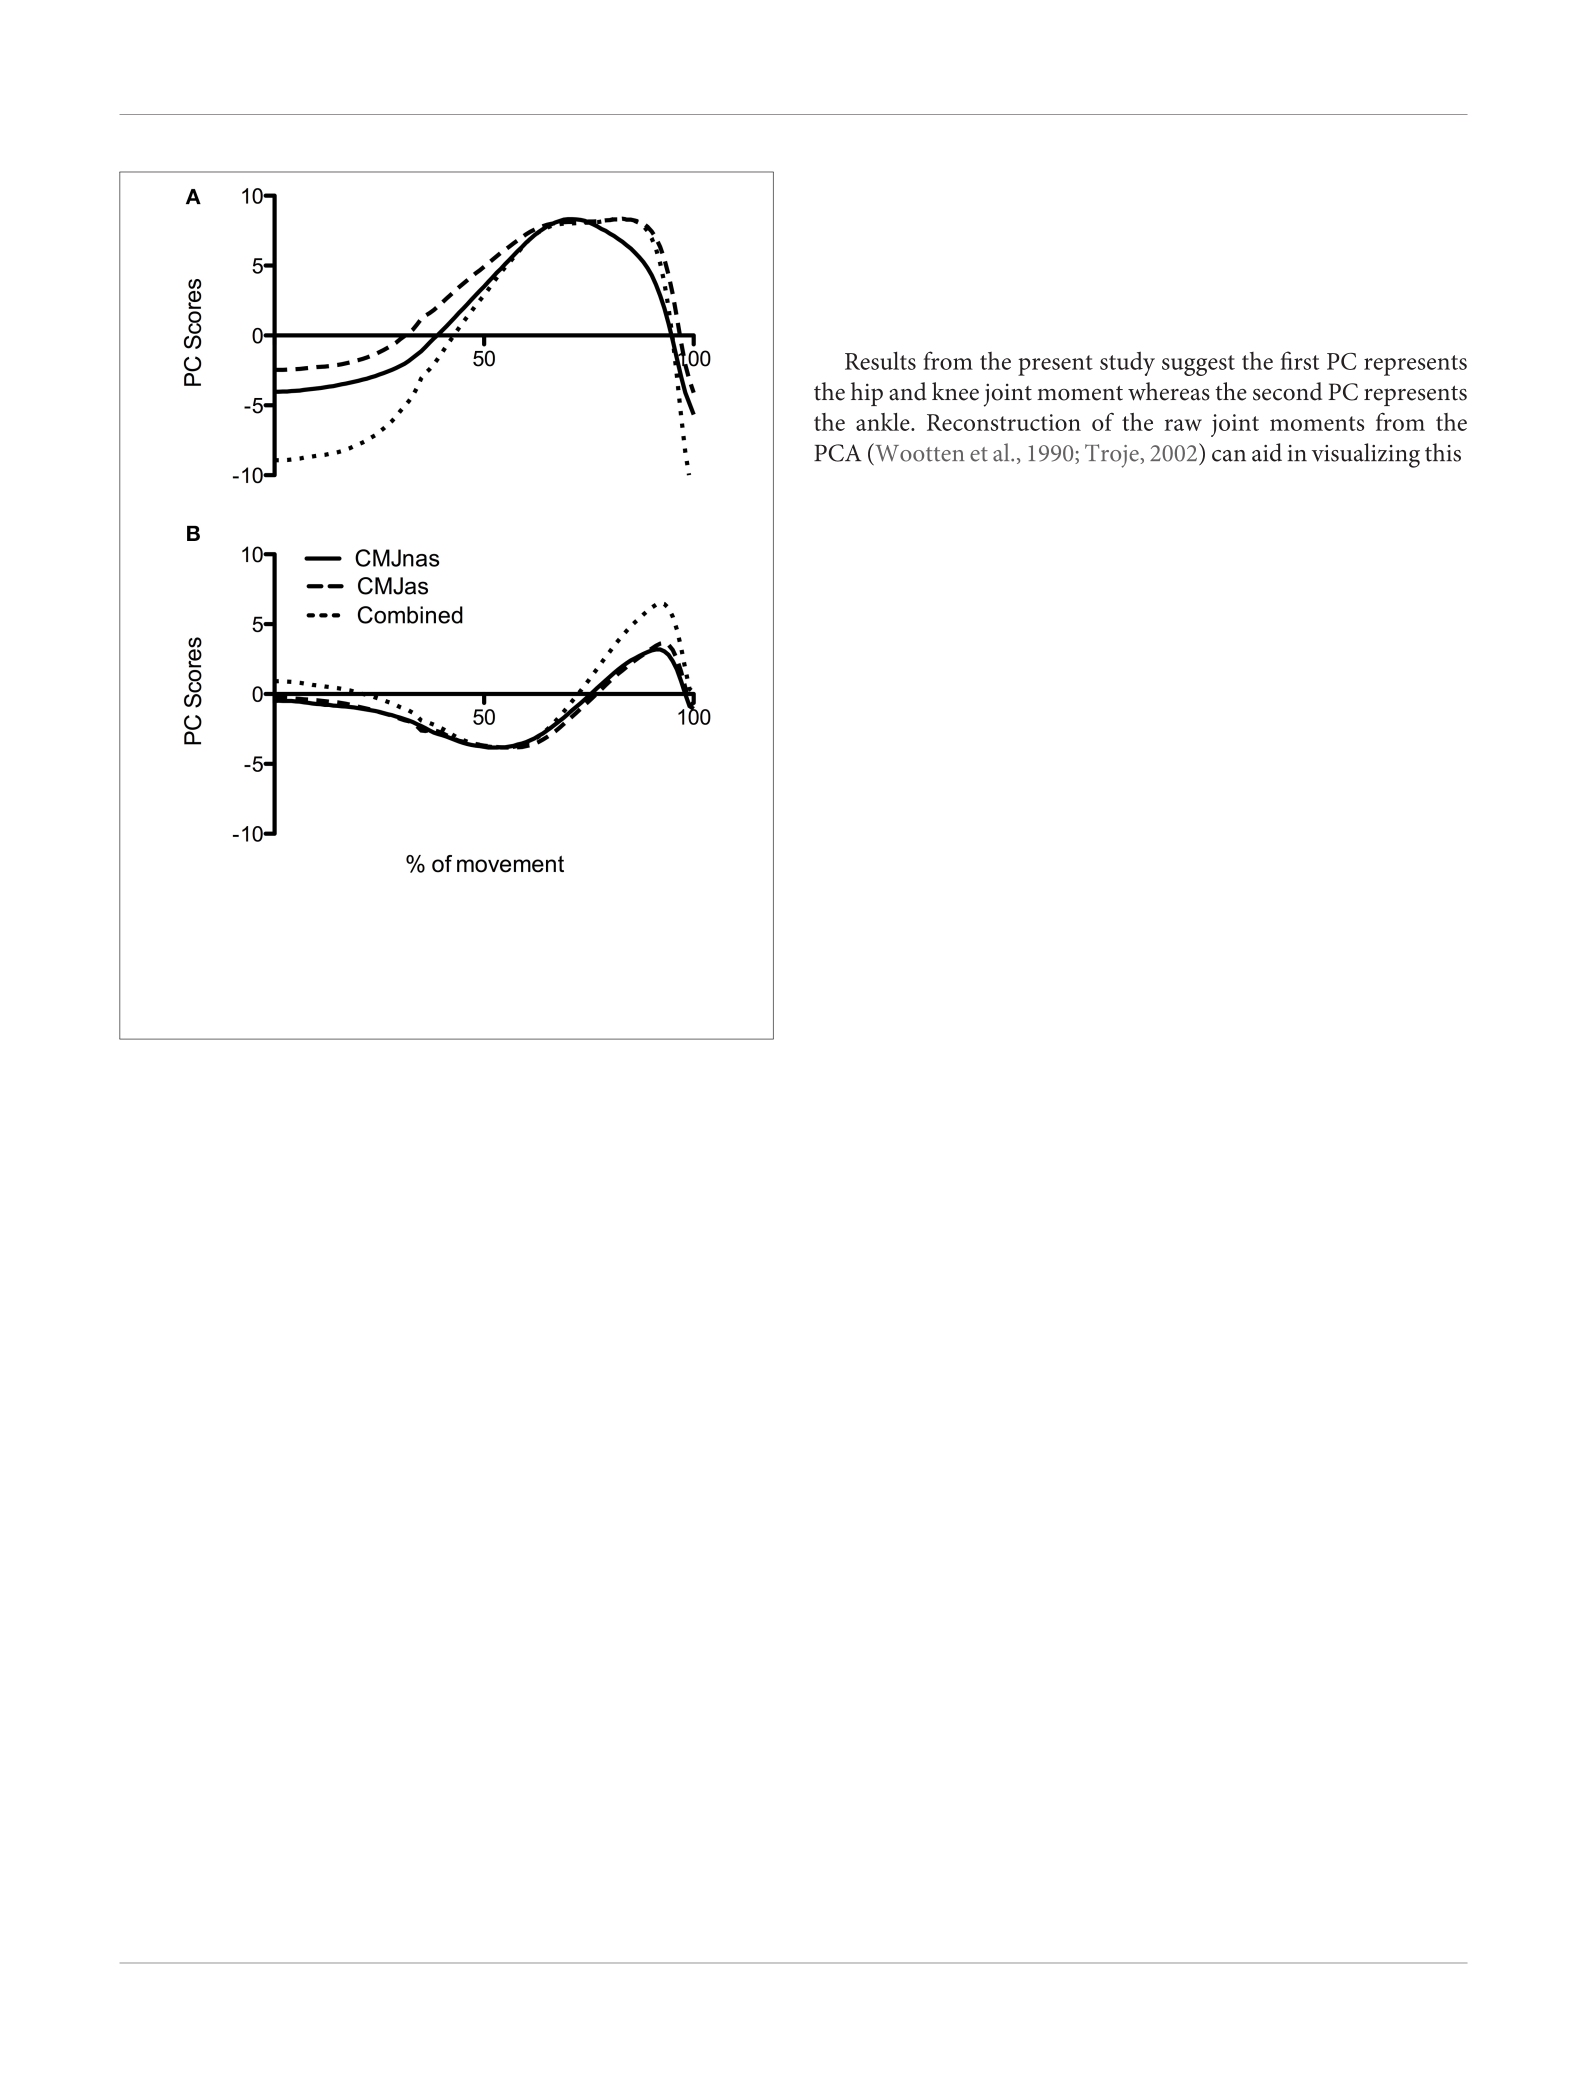
Cushion et al. PCA of Vertical Jumping
FIGURE 5 | Comparison of PC waveforms for CMJnas and CMJas for the 22
participants who completed both jumps along with PC waveform of combined
CMJnas and CMJas analysis (analysis 3): (A) PC1, (B) PC2. CMJas
waveforms have been flipped and data peaks matched to show differences in
temporal pattern.
the task from six components of ground reaction force data (see
Borzelli et al., 1999).
It is interesting to note that at only the group level an
additional PC was required to describe over 90% of the variance
within the dataset for CMJas. The need for the third PC is
indicative of the greater variability in the CMJas data. This
greater variability is seen both within individuals (see Figure 1)
and between individuals (see Figure 2), where a significant
difference in explained variance for PC1 was observed between
CMJnas and CMJas. In contrast, in analysis 4 (which essentially
eliminates the effect of within individual variation on the group
scores) only 2 PCs are required to explain 90% of the variance.
This improvement in predictive value is gained in the variance
explained by PC1g. It is interesting to consider the shape of
the PC3g score and think about the linear sum of the PC1g
score with PC3g score. In particular, the effect of adding PC3g
to PC1g is to make the curve less flat and to make it more
peaked toward the end of the jump. This type of variation is also
seen between individuals (Figure 2). It is also worth noting that
the requirement for a third PC for the group analysis provides
further support for the fact that the reduction to 2 PCs seen
for CMJnas is not trivial. The increase in variability within
the CMJas data could be related to unfamiliarity with the task
or complexity of the task for the participants involved. It has
previously been demonstrated an increase in complexity of a
task results in an increase in dimensionality and a reduction in
explained variance within the first principal component (Zago
et al., 2017). Whilst participants within this study were familiar
with jumping, the requirement to use an arm swing may have
added complexity to the task such that they were required
to explore movement options to a greater extent than in the
constrained CMJnas condition.
Results from the present study suggest the first PC represents
the hip and knee joint moment whereas the second PC represents
the ankle. Reconstruction of the raw joint moments from the
PCA (Wootten et al., 1990; Troje, 2002) can aid in visualizing this.
The reconstruction of the moment curves for a representative
individual (see Figure 6), shows the score for PC2i featuring
heavily in the linear sum of the reconstructed curve for the
ankle moments. Similarly, the first PC curve shares a similar
pattern to either the hip or knee joint moment curve—this varied
depending on the individual (for the individual in Figure 6 it
was hip-like). The relationship between the two PCs can also
be seen in Figure 7. Consider, for instance, the ankle moments
and compare jump1 to jump4. Here jump4 shows a flatter peak
compared to jump1 and a much wider curve. Consideration of
the 2 PC scores shows how these 2 quite different ankle moment
curves can still be constructed. In particular, the scores for PC1i,
and PC2i are out of phase, however the difference in timing
between them is such that they can still be summed to produce
all the different ankle curve combinations. To put this another
way, given the differences in the shape of the ankle curves we
know that at least 2 PCs would be needed to reconstruct them.
However, the 2 PCs that we obtain not only allow all of the
ankle moment curves to be created, but also all the hip and knee
moment curves. This synergy implies a relationship between the
different joint moment curves that persists across jumps.
This concept of synergy is not unique to this study and
demonstrates an approach of the system to optimize control of
motor tasks (see Santello et al., 1998; Jaric and Latash, 1999;
St-Onge et al., 2004; Todorov and Ghahramani, 2004; Latash
et al., 2007; Latash, 2010; Kipp et al., 2012; Nordin and Dufek,
2017). This organization of movement to synergies may occur
due to mechanical constraints (defined as limits in the options of
motion that can be achieved due to the mechanical configuration
of the human body) on the system that determine the movement
pattern—so called mechanical intelligence (Blickhan et al., 2006).
Within this study it is suggested that the proximal to distal
pattern of moment production (in the sagittal plane) during
vertical jumping might be governed by only 2 functional
DOF and this may be related to mechanical constraints. For
instance, Cleather (2018) has recently shown how the geometry
of the patellofemoral joint alone can explain over 90% of the
variance in the relative timing of femoral and tibial segment
moments (Cleather, 2018). To put that observation in terms
of the findings reported here, the patella could provide a
mechanical constraint that reduces 2 functional DOF to 1—
the hip and knee moments are largely dependent on one
another. This would then represent a potential explanation for
the remarkably consistent timing of moment production here. It
seems more credible that such consistency would be produced
by a mechanical feature of human anatomy that is shared by
all (a shared organismic mechanical constraint), than it being
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 7August 2019 | Volume 7 | Article 193
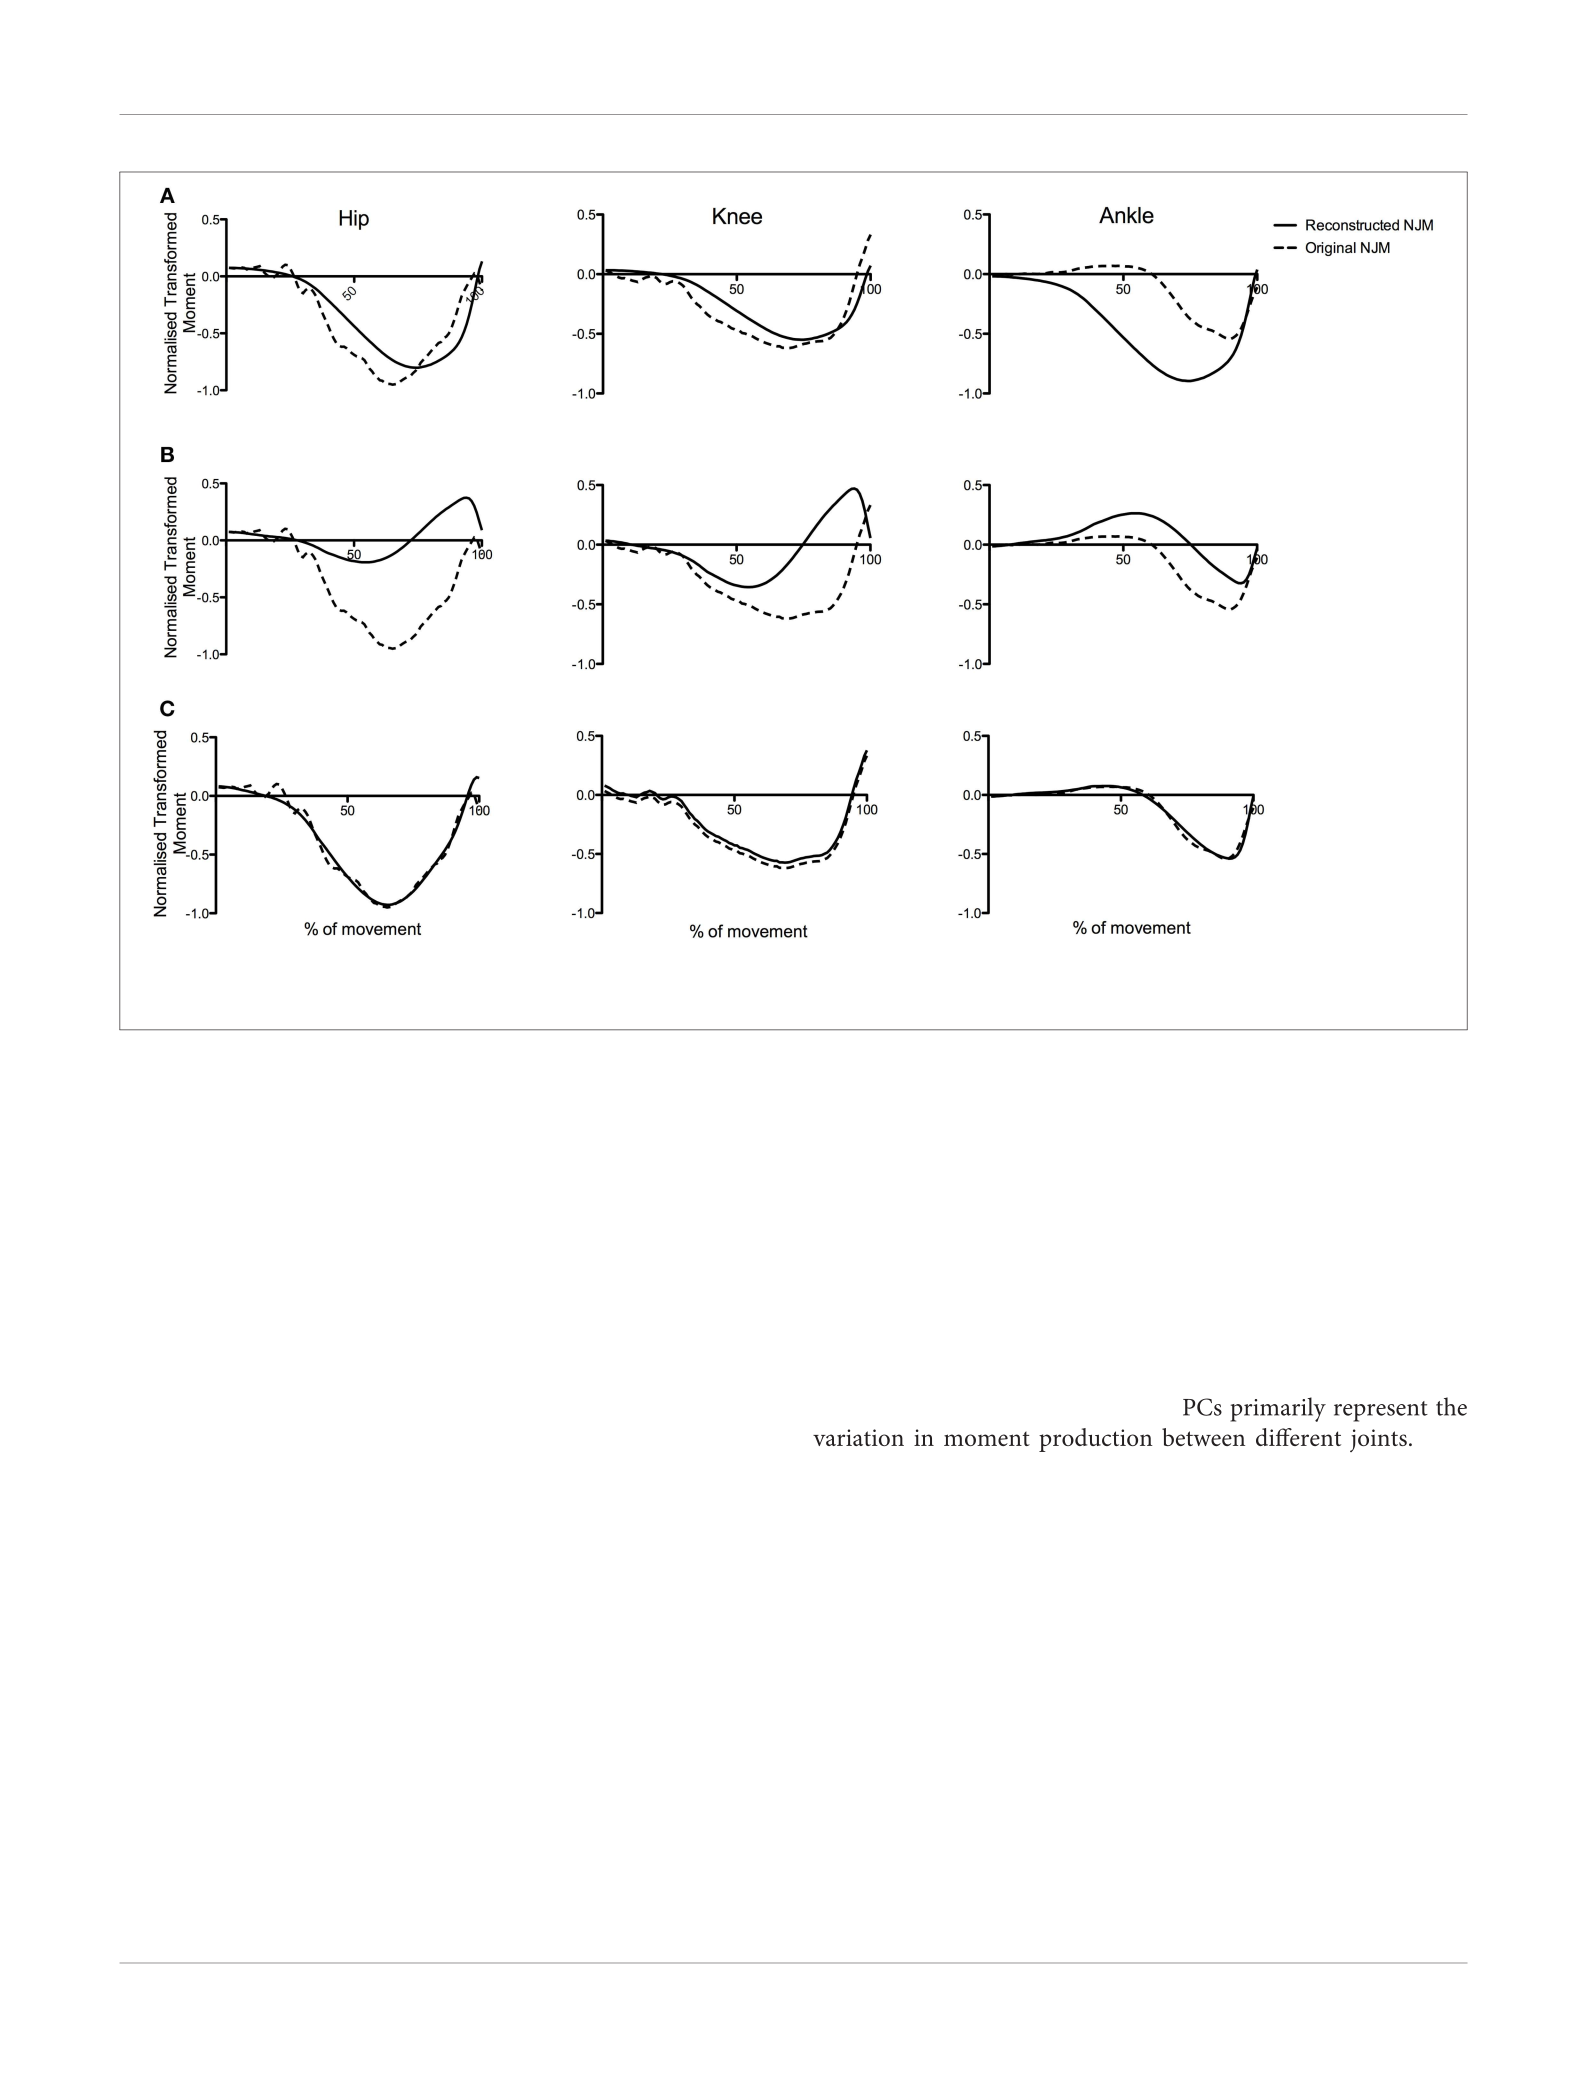
Cushion et al. PCA of Vertical Jumping
FIGURE 6 | Original NJMs (raw data) for a typical CMJnas compared with reconstructed data using only the first two principal components. The reconstructed curve
in (C) is the linear sum of the curves in (A,B).
the result of everyone learning a pattern of motor coordination
during their development that is so markedly consistent. A
similar conclusion of mechanical constraints reducing the
dimensionality of movement patterns has been proposed in a
similar, albeit much slower task of sit to stand (Borzelli et al.,
1999) as well as in drop landings (Nordin and Dufek, 2017).
An additional comparison between CMJnas and CMJas was
made between only those individuals who had completed both
forms of the jump (Figures 4,5, analysis 3). This comparison
demonstrates that the PC2g scores are effectively the same. This
can be interpreted as suggesting that the ankle is being used in
the same way, and that the potential effect of the ankle on the
relative timing of hip and knee NJM is also the same. However,
there is a notable difference in the PC1g scores. Specifically,
Figure 4A shows PC1g curves between each jump. This shows
a PC1g curve for CMJas to exhibit a flatter peak along with a
greater area under the curve compared to the CMJnas condition.
This is likely to be reflective of the use of the arm swing to slow
joint extension and thus provide greater time for the musculature
to develop force (Feltner et al., 2004; Domire and Challis, 2010).
Previous literature (e.g., Lees et al., 2004; Hara et al., 2006)
has suggested that the use of the lower limb in CMJnas and
CMJas is distinct. The results reported here suggest that although
this is true, the motor control strategy only differs in terms of
the first PC, and that there is still a striking similarity between
the movements.
Whilst interesting and novel findings have been identified
within this study, limitations of this work should be highlighted.
Although statistically rigorous procedures have been employed,
the analysis of the results is in some parts interpretative. This is a
limitation of trying to describe the mechanics of movement from
statistical techniques—although it should be noted that we are
not alone in using this technique to tease out different sources
of variation (e.g., Daffertshofer et al., 2004). In particular, there
are multiple sources of variation—joints (hip, knee or ankle),
participant, trial, and type of jump (with or without arms). Our
contention in this paper is that the PCs primarily represent the
variation in moment production between different joints. This
can be inferred based upon the following reasoning. Firstly, the
PCA analysis was first performed considering each individual
separately—thus eliminating inter-individual variability—this
analysis produced similar PC1i and PC2i for each participant
suggesting that the PC1g and PC2g are not produced by inter-
individual variability. Secondly, the group PCA analysis was
performed on both the whole data set, and on a reduced data
set comprising the resulting PCs from the individual analysis.
Inter-trial variation for each individual would be to a large part
mitigated in the latter data set, yet there was little difference in
the results of these two analyses (Figure 3). This suggests that
inter-trial variability is not a major factor in the group PCs.
Thirdly, the variation based upon type of jump was quantified
by the comparison of CMJas and CMJnas in Figure 4, and the
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 8August 2019 | Volume 7 | Article 193
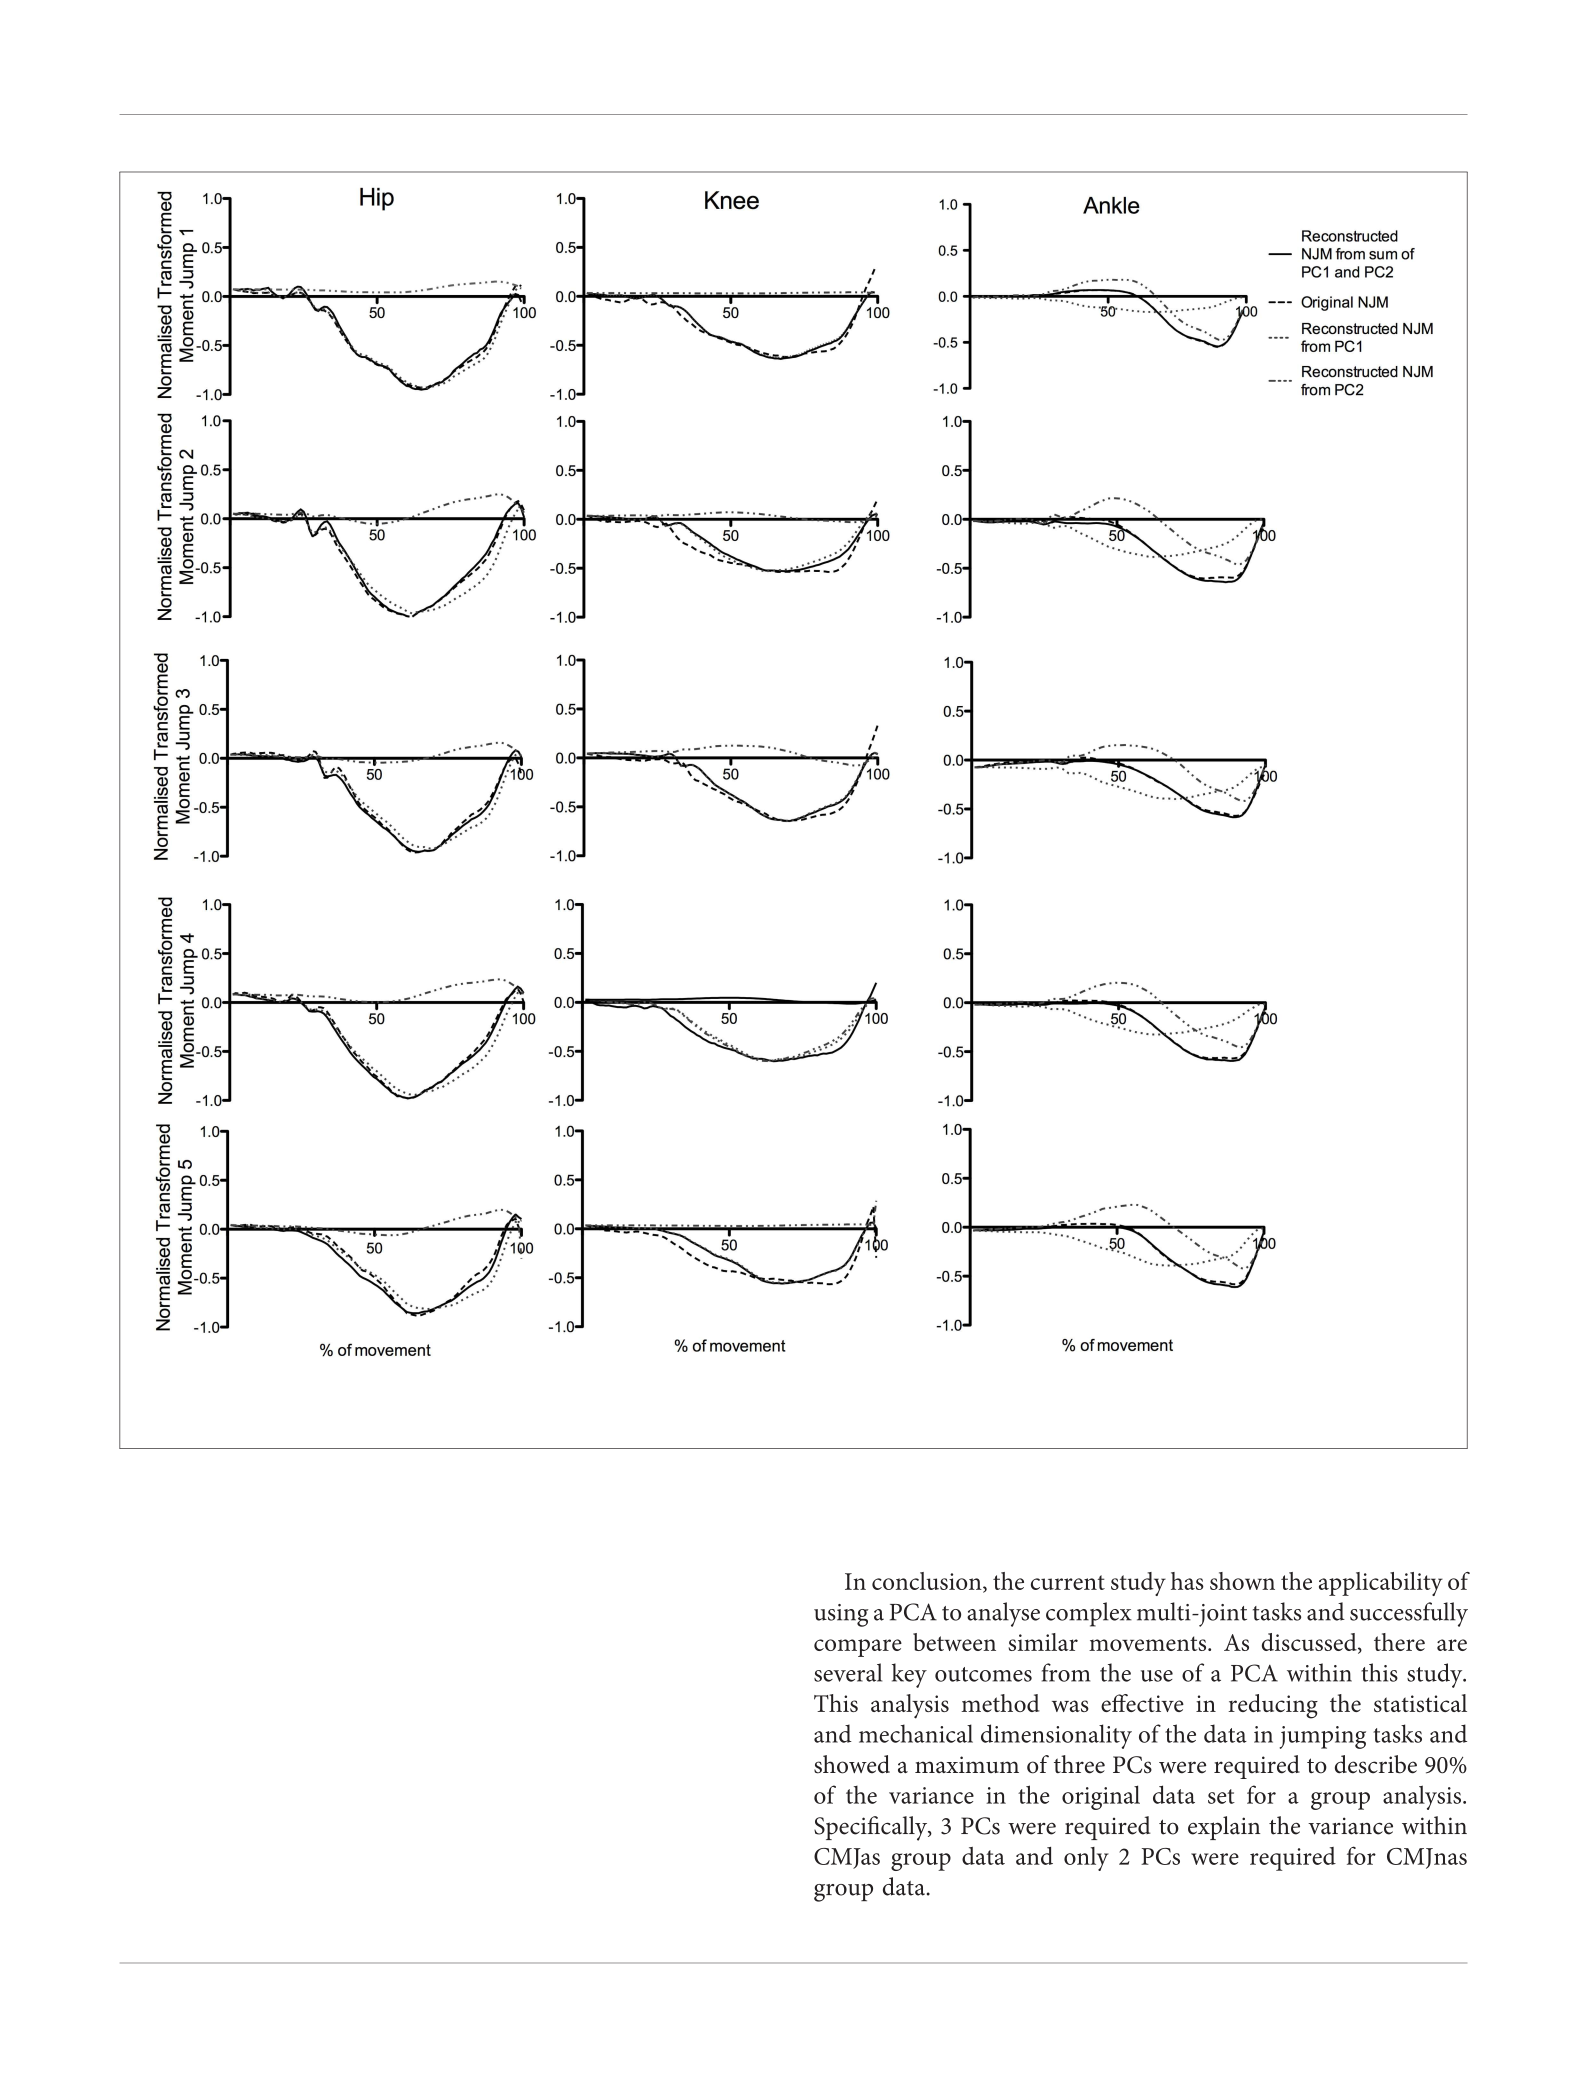
Cushion et al. PCA of Vertical Jumping
FIGURE 7 | Original NJMs (raw data) for a typical CMJnas compared with reconstructed data using only the first two principal components, for a representative
participant across five jump trials.
same PCs were found for both jump types. Having eliminated 3
of the 4 sources of variation, we suggest that the PCs from the
group analysis describe variation in joint moment production.
Of course, this contention has not been “proven” statistically,
but, we argue, is the only reasonable explanation. Furthermore,
Figures 6,7demonstrate the reconstruction of joint moments
from the PCA. This shows the similarity of the reconstructed
curves to the original raw joint moment curves. If variance was
predominantly from individual differences in jumping style, the
ability to so closely reconstruct the moment curves would likely
not occur. In addition, whilst the focus of this research was
on the analysis of the lower limb during jumping, based on
their large contribution to the movement, future research would
benefit from conducting a whole-body analysis to determine the
dimensionality of the system.
In conclusion, the current study has shown the applicability of
using a PCA to analyse complex multi-joint tasks and successfully
compare between similar movements. As discussed, there are
several key outcomes from the use of a PCA within this study.
This analysis method was effective in reducing the statistical
and mechanical dimensionality of the data in jumping tasks and
showed a maximum of three PCs were required to describe 90%
of the variance in the original data set for a group analysis.
Specifically, 3 PCs were required to explain the variance within
CMJas group data and only 2 PCs were required for CMJnas
group data. The first PC has a greater loading for hip and knee
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 9August 2019 | Volume 7 | Article 193
Cushion et al. PCA of Vertical Jumping
joint moments, whereas the second PC has a greater loading
for the ankle joint moment. The results suggest the proximal to
distal extension pattern in the sagittal plane typical of vertical
jumping tasks is governed by only 2 functional DOF rather than
the previously reported 3 mechanical DOF. This study adds to the
motor control literature suggesting that despite the redundancy
within the system coordinated movements are produced based
on task and mechanical constraints. Importantly, the results
suggest vertical jumping is controlled by 2 functional DOF at
both an individual and group level. We suggest the reduction
in dimensionality of the movement may be mechanically driven
by human anatomy.
ETHICS STATEMENT
All subjects gave written informed consent in accordance with the
Declaration of Helsinki. The protocol was approved by the ethics
sub-committee of St Mary’s University.
AUTHOR CONTRIBUTIONS
EC, JN, and DC were involved in the design of the
study. EC carried out all data collection. All authors
were involved in the interpretation and final write
up of the study.
REFERENCES
Balasubramaniam, R., and Turvey, M. T. (2004). Coordination modes in
the multisegmental dynamics of hula hooping. Biol. Cybern. 90, 176–190.
doi: 10.1007/s00422-003-0460-4
Bates, B. T. (1996). Single-subject methodology: an alternative approach. Med. Sci.
Sports. Exerc. 28, 631–638. doi: 10.1249/00005768-199605000-00016
Bernstein, N. A. (1967). The Co-ordination and Regulation of Movements. Oxford:
Pergamon Press.
Blickhan, R., Seyfarth, A., Geyer, H., Grimmer, S., Wagner, H., and Gunther,
M. (2006). Intelligence by mechanics. Phil. Trans. R. Sco. A. 365, 199–220.
doi: 10.1098/rsta.2006.1911
Bobbert, M. F., and van Ingen Schenau, G. J. (1988). Coordination in vertical
jumping. J. Biomech. 21, 249–262. doi: 10.1016/0021-9290(88)90175-3
Borzelli, G., Cappizzon, A., and Papa, E. (1999). Inter and intra
individual variability of ground reaction forces during sit to stand
with principal component analysis. Med. Eng. Phys. 21, 235–240.
doi: 10.1016/S1350-4533(99)00050-8
Button, C., MacLeod, M., Sanders, R., and Coleman, S. (2003). Examining
movement variability in the basketball free-throw action at different skill levels.
Res. Q. Exerc. Sport. 74, 257–269. doi: 10.1080/02701367.2003.10609090
Chiu, L. Z. F., and Salen, G. J. (2010). Pelvic kinematic method for determining
vertical jump height. J. App. Biomech. 26, 508–511. doi: 10.1123/jab.26.4.508
Chow, J. Y., Davids, K., Button, C., and Rein, R. (2008). Dynamics of movement
patterning in learning a discrete multiarticular action. Motor Control 12,
219–240. doi: 10.1123/mcj.12.3.219
Cleather, D. J. (2018). The patella: a mechanical determinant of
coordination during vertical jumping. J. Theor. Biol. 446, 205–211.
doi: 10.1016/j.jtbi.2018.03.013
Cleather, D. J., and Bull, A. M. J. (2015). The development of a segment based
musculoskeletal model of the lower limb: introducing freebody. R. Soc. Open
Sci. 2, 140–449. doi: 10.1098/rsos.140449
Cleather, D. J., Goodwin, J. E., and Bull, A. M. J. (2013). Inter-segmental moment
analysis characterises the partial correspondence of jumping and jerking. J.
Strength. Cond. Res. 27, 89–100. doi: 10.1519/JSC.0b013e31825037ee
Daffertshofer, A., Lamoth, C. J., Meijer, O. G., and Beek, P. J. (2004). PCA in
studying coordination and variability: a tutorial. Clin. Biomech. 19, 415–428.
doi: 10.1016/j.clinbiomech.2004.01.005
Deluzio, K. J., and Astephen, J. L. (2007). Biomechanical features of gait waveform
data associated with knee osteoarthritis an application of principal component
analysis. Gait Posture. 25, 86–93. doi: 10.1016/j.gaitpost.2006.01.007
Deluzio, K. J., Wyss, U. P., Zee, B., Costigan, P. A., and Serbie, C.
(1997). Principal component models of knee kinematics and kinetics:
normal vs. pathological gait patterns. Hum. Movement. Sci. 16, 201–217.
doi: 10.1016/S0167-9457(96)00051-6
Domire, Z. J., and Challis, J. H. (2010). An induced energy analysis to determine
the mechanism for performance enhancement as a result of arm swing during
jumping. Sports. Biomech. 9, 38–46. doi: 10.1080/14763141003692639
Dona, G., Preatoni, E., Cobelli, C., Rodano, R., and Harrison, A. J.
(2009). Application of functional principal component analysis in
race walking: an emerging methodology. Sports. Biomech. 8, 284–301.
doi: 10.1080/14763140903414425
Dufek, J. S., Bates, B. T., Stergiou, N., and James, C. R. (1995). Interactive effects
between group and single-subject response patterns. Hum. Movement Sci, 14,
301–323. doi: 10.1016/0167-9457(95)00013-I
Federolf, P. A., Boyer, K. A., and Andriacchi, T. P. (2013). Application of principal
component analysis in clinical gait research: identification of systematic
differences between healthy and medial knee-osteoarthritic gait. J. Biomech. 46,
2173–2178. doi: 10.1016/j.jbiomech.2013.06.032
Feltner, M. E., Bishop, E. J., and Perez, C. M. (2004). Segmental and kinetic
contributions in vertical jumps performed with and without an arm swing. Res.
Q. Exerc. Sport. 75, 216–230. doi: 10.1080/02701367.2004.10609155
Forner-Cordero, A., Levin, O., Li, Y., and Swinnen, S. P. (2005). Principcal
component analysis of complex multi-joint coordinative movements. Biol.
Cybern. 93, 63–78. doi: 10.1007/s00422-005-0582-y
Hara, M., Shibayama, A., Takeshita, D., and Fukashiro, S. (2006). The effects of
arm swing on lower extremities in vertical jumping. J. Biomech. 39, 2503–2511.
doi: 10.1016/j.jbiomech.2005.07.030
Hristovski, R., Davids, K., Araujo, D., and Button, C. (2006). How boxers decide to
punch a target: emergent behaviour in nonlinear dynamical movement systems.
J. Sports. Sci. Med. 5, 60–73.
James, C. R., Atkins, L. T., Dufek, J. S., and Bates, B. T. (2014). An exploration of
load accommodation strategies during walking with extremity carried weights.
Hum. Movement Sci. 35, 17–29. doi: 10.1016/j.humov.2014.03.012
James, C. R., and Bates, B. T. (1997). Experimental and statistical design
issues in human movement research. Meas. Phys. Educ. Exerc. Sci. 1, 55–69.
doi: 10.1207/s15327841mpee0101_4
James, C. R., Bates, B. T., and Dufek, J. S. (2003). Classification and comparison of
biomechanical response strategies for accommodating landing impact. J. App.
Biomech. 19, 106–118. doi: 10.1123/jab.19.2.106
Jaric, S., and Latash, M. L. (1999). Learning a pointing task with a
kinematically redundant limb: emerging synergies and patterns of final position
variability. Hum. Movement Sci. 18, 819–838. doi: 10.1016/S0167-9457(99)0
0042-1
Jolliffe, I. T. (2002). “Graphical representation of data using principal components,”
in Principal Component Analysis. Springer Series in Statistics, 2nd Edn (New
York, NY: Springer), 78–110.
Jolliffe, I. T., and Cadima, J. (2016). Principal component analysis: a
review and recent development. Phil. Trans. R. Soc. 374:20150202.
doi: 10.1098/rsta.2015.0202
Ketcham, C. J., Seidler, R. D., van Gemmert, A. W. A., and Stelmach, G. E. (2002).
Age related kinematic differences as influenced by task difficulty, target size and
movement amplitude. J. Gerontol. 57, 54–64. doi: 10.1093/geronb/57.1.P54
Kipp, K., Redden, J., Sabick, M., and Harris, C. (2012). Kinematic and kinetic
synergies of the lower extremities during the pull in olympic weightlifting. J.
App. Biomech. 28, 271–278. doi: 10.1123/jab.28.3.271
Kollias, I., Hatzitaki, V., Papaiakovou, G., and Giatsis, G. (2001). Using
principal components analysis to identify individual differences
in vertical jump performance. Res. Q. Exerc. Sport. 72, 63–67.
doi: 10.1080/02701367.2001.10608933
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 10 August 2019 | Volume 7 | Article 193
Cushion et al. PCA of Vertical Jumping
Laffaye, G., Bardy, B. G., and Durey, A. (2007). Principal component structure and
sport specific differences in the running on leg vertical jump. Int. J. Sports. Med.
28, 420–425. doi: 10.1055/s-2006-924507
Lamoth, C. J. C., Daffertshofer, A., Meijer, O. G., and Beek, P. J. (2006). How do
persons with chronic low back pain speed up and slow down? trunk-pelvis
coordination and lumbar erector spinae activity during gait. Gait Posture. 23,
230–239. doi: 10.1016/j.gaitpost.2005.02.006
Latash, M. (2000). There is no motor redundancy in human movements. There is
motor abundance. Motor Control. 4, 259–261. doi: 10.1123/mcj.4.3.259
Latash, M. (2010). Motor synergies and the equilibrium point hypothesis. Motor
Control. 14, 294–322. doi: 10.1123/mcj.14.3.294
Latash, M., Scholz, J. P., and Schoner, G. (2007). Toward a new theory of motor
synergies. Motor Control. 11, 276–308. doi: 10.1123/mcj.11.3.276
Lee, M., Roan, M., and Smith, B. (2009). An application of principal component
analysis for lower body kinematics between loaded and unloaded walking. J.
Biomech. 42, 2226–2230. doi: 10.1016/j.jbiomech.2009.06.052
Lees, A., Vanrenterghem, J., and De Clercq, D. (2004). Understanding how an arm
swing enhances performance in the vertical jump. J. Biomech. 37, 1929–1940.
doi: 10.1016/j.jbiomech.2004.02.021
Majed, L., Heugas, A. M., and Siegler, I. A. (2017). Changes in movement
organization and control strategies when learning a biomechanically
constrained gait pattern, racewalking: a PCA study. Exp. Brain. Res. 235,
931–940. doi: 10.1007/s00221-016-4853-8
Newell, K. M. (1986). “Constraints on the development of coordination,” in Motor
Development in Children: Aspect of Coordination and Control, eds M. G. Wade
and H. T. A. Whiting (Dordrecht: Nijhoff), 341–360.
Nordin, A. D., and Dufek, J. S. (2016a). Neuromechanical synergies in single leg
landing reveal changes in movement control. Hum. Movement Sci. 49, 66–78.
doi: 10.1016/j.humov.2016.06.007
Nordin, A. D., and Dufek, J. S. (2016b). Single leg landing neuromechanical
data following load and land height manipulations. Data Brief 8, 1024–1030.
doi: 10.1016/j.dib.2016.07.011
Nordin, A. D., and Dufek, J. S. (2017). Load accommodation strategies and
movement variability in single leg landing. J. App. Biomech. 33, 241–247.
doi: 10.1123/jab.2016-0097
Nordin, A. D., and Dufek, J. S. (2019). Reviewing the variability-overuse injury
hypothesis: does movement variability relate to landing injuries? Res. Q. Exerc.
Sport. 90, 190–205. doi: 10.1080/02701367.2019.1576837
Nordin, A. D., Dufek, J. S., James, C. R., and Bates, B. T. (2017). Classifying
performer strategies in drop landing activities. J. Sports. Sci. 35, 1858–1863.
doi: 10.1080/02640414.2016.1240876
Orth, D., Davids, K., and Seifert, L. (2018). Constraints representing a meta-
stable regime facilitate exploration during practice and transfer of learning
in a complex multi-articular task. Hum. Movement Sci. 57, 291–302.
doi: 10.1016/j.humov.2017.09.007
Raffalt, P. C., Alkjaer, T., and Simonsen, E. B. (2016). Intra and inter
subject variation in lower limb coordination during countermovement
jumps in children and adults. Hum. Movement Sci. 46, 63–77.
doi: 10.1016/j.humov.2015.12.004
Richter, C., O’Connor, N. E., Marshall, B., and Moran, K. (2014). Comparison
of discrete point vs dimensionality reduction techniques for describing
performance related aspects of maximal vertical jumping. J. Biomech. 47,
3012–3017. doi: 10.1016/j.jbiomech.2014.07.001
Santello, M., Flanders, M., and Soechting, J. F. (1998). Postural
hand synergies for tool use. J. Neurosci. 18, 10105–10115.
doi: 10.1523/JNEUROSCI.18-23-10105.1998
Scholz, J., Schoner, G., and Latash, M. (2000). Identifying the control structure of
multijoint coordination during pistol shooting. Exp. Brain. Res. 135, 382–404.
doi: 10.1007/s002210000540
Scholz, J. P., Reisman, D., and Schoner, G. (2001). Effects of varying task
constraints on solutions to joint coordination in a sit to stand task. Exp. Brain.
Res. 141, 485–500. doi: 10.1007/s002210100878
Scholz, J. P., and Schoner, G. (1999). The uncontrolled manifold concept:
identifying control variables for a functional task. Exp. Brain. Res. 126, 289–306.
doi: 10.1007/s002210050738
Seifert, L., Chollet, D., and Rouard, A. (2007). Swimming constraints
and arm coordination. Hum. Movement Sci. 26, 68–86.
doi: 10.1016/j.humov.2006.09.003
Seifert, L., Leblanc, H., Herault, R., Komar, J., Button, C., and Chollet, D.
(2011). Inter-individual variability in the upper lower limb breaststroke
coordination. Hum. Movement Sci. 30, 550–565. doi: 10.1016/j.humov.201
0.12.003
Soechting, J. F., and Flanders, M. (1997). Flexibility and repeatability of finger
movements during typing: analysis of multiple degrees of freedom. J. Comput.
Neurosci. 4, 29–46. doi: 10.1023/A:1008812426305
St-Onge, N., Duval, N., Yahia, L.’H., and Feldman, A. G. (2004). Interjoint
coordination in lower limbs in patients with a rupture of the anterior cruciate
ligament of the knee joint. Knee. Surg. Sports. Traumatol. Arthrosc. 12, 203–216.
doi: 10.1007/s00167-003-0420-5
Todorov, E., and Ghahramani, Z. (2004). “Analysis of the synergies underlying
complex hand manipulation,” in The 26th Annual International Conference of
the IEEE Engineering in Medicine and Biology Society, Vol. 2 (San Francisco,
CA: IEEE), 4637–4640. doi: 10.1109/IEMBS.2004.1404285
Troje, N. F. (2002). Decomposing biological motion: a framework for analysis and
synthesis of human gait patterns. J. Vis. 2:2. doi: 10.1167/2.5.2
Verrel, J., Pologe, S., Manselle, W., Lindenberger, U., and Woollacott,
M. (2013). Coordination of degrees of freedom and stabilization of
task variables in a complex motor skill: expertise-related differences in
cello bowing. Exp. Brain. Res. 224, 323–334. doi: 10.1007/s00221-012-
3314-2
Winter, D. A. (2005). Biomechanics and Motor Control of Human Movement. 3rd
ed. Hoboken, NJ; John Wiley & Sons, Inc.
Witte, K., Ganter, N., Baumgard, C., and Peham, C. (2010). Applying a principal
component analysis to movement coordination in sport. MCMDS 16, 477–488.
doi: 10.1080/13873954.2010.507079
Witte, K., Schobesberger, H., and Peham, C. (2009). Motion pattern analysis of
gait in horseback riding by means of principal component analysis. Hum.
Movement Sci. 28, 394–405. doi: 10.1016/j.humov.2009.04.002
Wootten, M. E., Kadaba, M. P., and Cochran, G. V. B. (1990). Dynamic
electromyography. I. Numerical representation using principal
component analysis. J. Orthop. Res. 8, 247–258. doi: 10.1002/jor.11000
80214
Zago, M., Pacifici, I., Lovecchio, N., Galli, M., Federolf, P. A., and Sforza,
C. (2017). Multi-segmental movement patterns reflect juggling complexity
and skill level. Hum. Movement Sci. 54, 144–153. doi: 10.1016/j.humov.201
7.04.013
Conflict of Interest Statement: The authors declare that the research was
conducted in the absence of any commercial or financial relationships that could
be construed as a potential conflict of interest.
Copyright © 2019 Cushion, Warmenhoven, North and Cleather. This is an open-
access article distributed under the terms of the Creative Commons Attribution
License (CC BY). The use, distribution or reproduction in other forums is permitted,
provided the original author(s) and the copyright owner(s) are credited and that the
original publication in this journal is cited, in accordance with accepted academic
practice. No use, distribution or reproduction is permitted which does not comply
with these terms.
Frontiers in Bioengineering and Biotechnology | www.frontiersin.org 11 August 2019 | Volume 7 | Article 193

1
EXSC: 550 (Article Review) PCA Vertical Jumping
Student’s Name
Institutional Affiliation

2
I. Cushion, E., Warmenhoven, J., North, J., & Cleather, D. (2019). Principal Component
Analysis Reveals the Proximal to Distal Pattern in Vertical Jumping Is Governed by
Two Functional Degrees of Freedom. Frontiers in Bioengineering and
Biotechnology, 7(193), 1-11. https://doi.org/10.3389/fbioe.2019.00193
Although the article was published in 2019, it was submitted to Biomechanics, a
section of the journal Frontiers in Bioengineering and Biotechnology, in 2018.
The article was peer-reviewed by Francesco Travascio from the University of
Miami, United States; and Andrew D. Nordin from the University of Florida,
United States. It was edited by Veronica Cimolin, from Politecnico di Milano,
Italy.
II.
a. Objectives
According to the authors, people usually find it easy to perform daily activities
like walking or climbing a flight of stairs. Oblivious to them is the complex
coordination and control and control of the multiple degrees of freedom
(DOF) that occurs with each motor movement. Based on these notions, the
authors were motivated to perform a study to determine the fundamentals of
motor skills in vertical jumping. In this study, the authors aimed to complete a
comparative analysis of emerging coordination strategies individuals use in
vertical jumping in the face of two task restraints “countermovement jump
(CMJ) with arm swing-CMJas and no arm swing-CMJnas” (p. 1). The authors
argued that identifying these movement features helps develop people's
understanding of the control strategies for motor movements that are used to
control movements under different task limitations.
b. Methods

3
The study involved 24 males and 14 females, totaling 38 individuals who
volunteered to be part of the study. The authors did not include the
specifications of the race or religion of the participants. However, the
participants had a median age of 27 ± 5 years; height = 174.4 ± 9.0 cm, and
body mass 78.1 ± 14.1 kg. They had no musculoskeletal injuries and signed
informed consent after being provided with details regarding the study. The
authors collected kinematic data using a Vicon motion capture system with 14
LED cameras that tracked the reflective markers at a sampling frequency of
200 Hz. To collect the kinetic data, the authors used force plates positioned
flush to the laboratory floor (Kistler Type 9287BA, Bioware 3.24 software,
Kistler Instruments Ltd, Hampshire, UK), at a rate of 1,000 Hz and
synchronized with the Vicon system. The authors used 5th order Woltring
filter with a cut-off frequency of 10 Hz to filter all the data. Data analysis was
based on the propulsive phase of the vertical jump. Cushion, Warmenhoven,
North, & Cleather (2019) used PCA to extract common patterns of moment
production during the vertical jump under two task constraints. They argued
that this approach effectively retained the spatiotemporal pattern in the time
series data while detecting coordination patterns both within and between
individuals. Cushion et al. (2019) used an independent sample t-test to assess
the group differences between PC1, PC2, and the sum of PC1 and PC2.
c. Results
The primary outcome of the study was that based on all the comparisons taken
into consideration in the study, “90% of the variance in the raw data could be
described by at most 3 PCs, and in many cases by 2” (p. 6). The results
indicate that the PCs in the current study defines the variance in joint moments

4
during jumping, showing that joint moment production both between and
within individuals and within each task has the same structural patterns. The
authors found that the “dimensionality of sagittal plane lower limb extension
in some forms of vertical jumping can be reduced to only two functional
DOF” (p. 6). Cushion et al. (2019) argued that this finding was significant
because it shows that offering the individuals a simple task constraint such as
“jump as high as you can” produces an evidently similar pattern.
d. Summary
The authors based their study on the idea that motor movements include a
series of coordination and control of the multiple degrees of freedom (DOF)
that accompanies each movement. They argued that while several studies have
been conducted on the same, they used the PCA analysis because it has the
benefit of holding the spatiotemporal pattern in the time series data whilst
sensing patterns of coordination both between and within individuals. The
results indicated a significant conclusion; offering the individuals a simple
task constraint evidently produces a similar pattern.
e. Critique
While the authors focus on establishing the significance of PCA in analyzing
multi-factor analysis, the more important finding in this study is the
significance of coordination and control of the multiple degrees of freedom.
Such findings indicate a better opportunity for increased awareness of the
importance of understanding the foundations of motor movements. In line
with this argument, 2 Corinthians 9:8 states that “And God can make all grace
abound to you, so that having all sufficiency in all things at all times, you may
abound in every good work.”

5
III. Question/Application
Question: How do individuals control the lower limbs' multiple degrees of freedom
(DF) in producing the oscillations?
Facts:
Individuals can be motivated to improve their motor movement performance,
vertical jumping by simple constraints.
Understanding the control and coordination mechanism for the DF is essential
in physical training.

6
Reference
Cushion, E., Warmenhoven, J., North, J., & Cleather, D. (2019). Principal Component
Analysis Reveals the Proximal to Distal Pattern in Vertical Jumping Is Governed by
Two Functional Degrees of Freedom. Frontiers in Bioengineering and
Biotechnology, 7(193), 1-11. https://doi.org/10.3389/fbioe.2019.00193

